Chapter 6: Evolution
In December 1938, a fishing trawler hauled up an unusual catch off the coast of East London, South Africa. Among the ordinary fish lay a heavy, steel-blue creature nearly one and a half metres long, with thick limb-like fins and hard scales unlike anything the crew had ever seen. A young museum curator named Marjorie Courtenay-Latimer was called to examine it. She could not name it, but she sensed it was important and worked hard to preserve the strange specimen. When the fish expert J. L. B. Smith finally studied it, he was astonished. This was a coelacanth — a fish known until then only from fossils, believed to have disappeared from the Earth more than sixty million years ago, long before the last dinosaurs died out. Yet here it was, alive.
The discovery stunned the world. A “living fossil” had been swimming quietly in the deep ocean all this time, almost unchanged, while entire groups of animals appeared, ruled the planet, and vanished around it. The coelacanth is a living reminder that the history of life is astonishingly long, deeply connected, and still full of surprises. In this chapter we trace that history — from the birth of the universe and the very first cell, through the branching descent of countless species, all the way to the appearance of human beings.
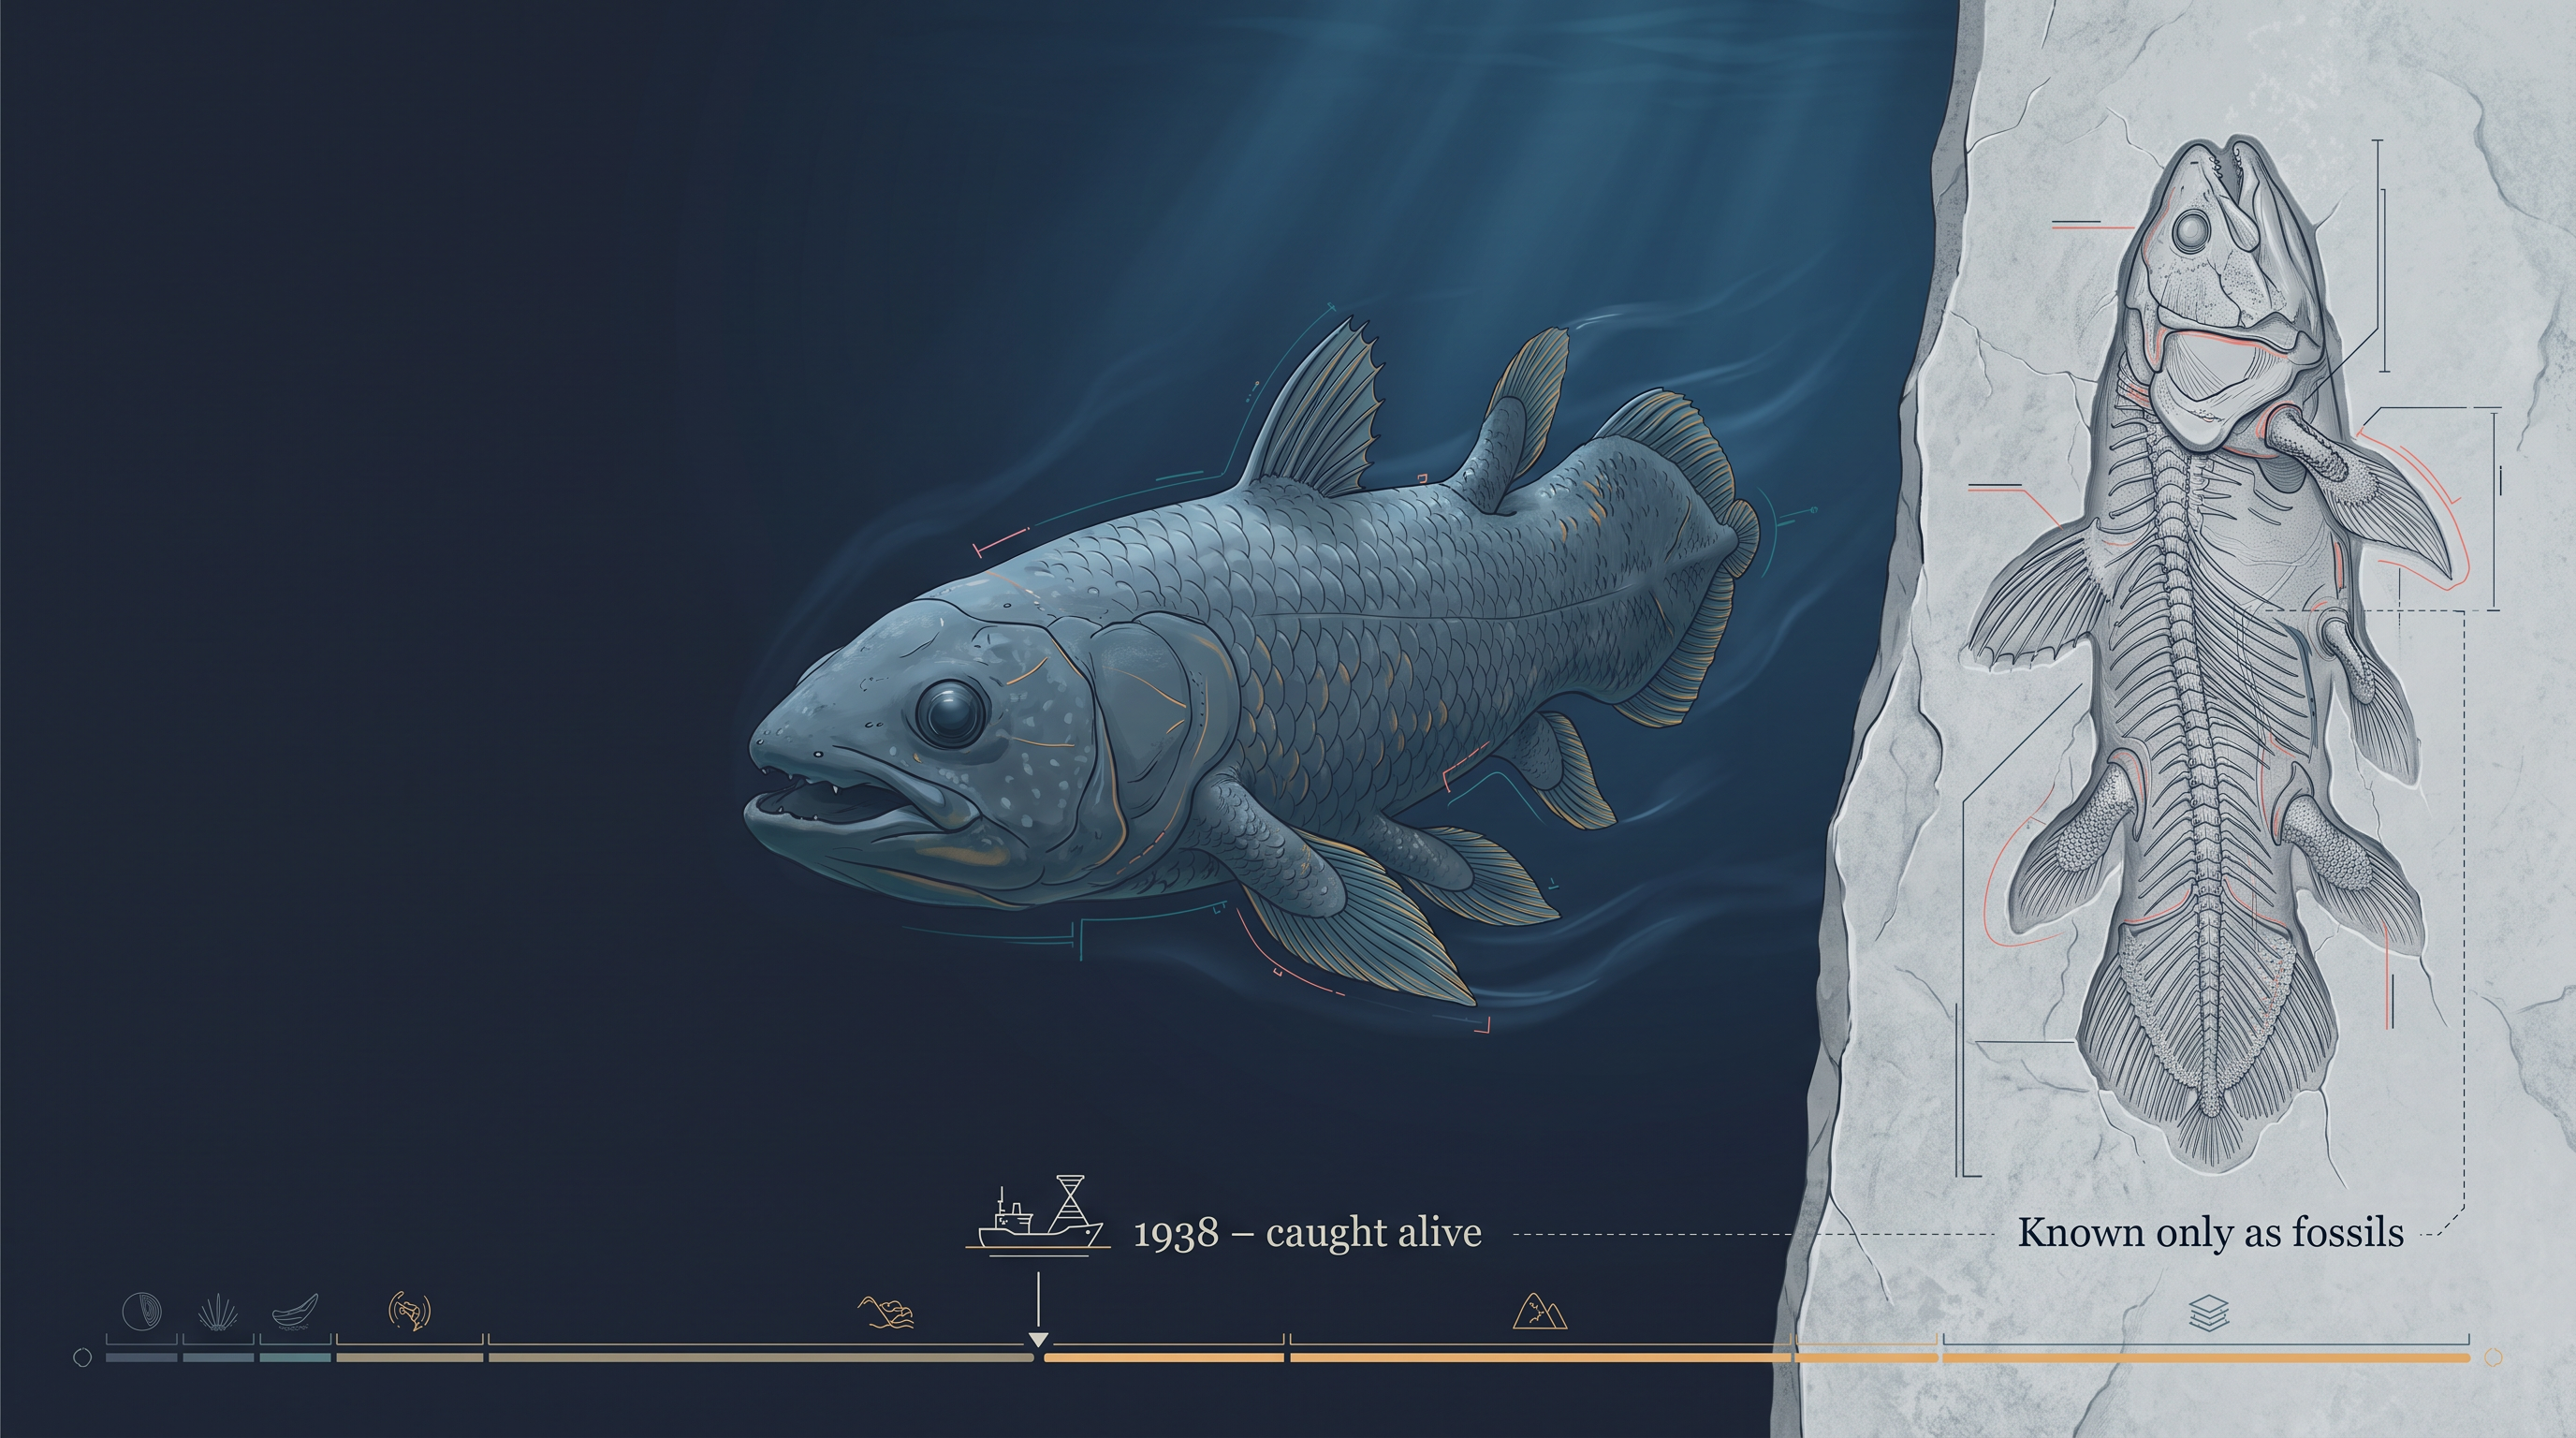
Fig. 6.0 – The coelacanth: a living fossil.
By the end of this chapter, you will be able to answer each of these questions for yourself.
6.1 Origin of Life
Evolutionary biology is the study of the history of life forms on Earth — how living things have changed and diversified over enormous spans of time. But before we can understand how life changed, we must first ask a deeper question: how did life begin at all? To answer that, we have to step back even further and think about the origin of the Earth, the stars, and indeed the whole universe. The story that follows is one of the longest stories ever told, pieced together from clues rather than eyewitness accounts — the story of how life and its rich diversity came to exist on our planet.
Looking Back in Time
When we gaze at stars on a clear night, we are, in a strange way, looking into the past. Distances between stars are so vast that they are measured in light years — the distance light travels in one year. The light entering your eye from a distant star began its journey millions of years ago, from trillions of kilometres away, and is only reaching you now.
Objects near us are different. When we look at things around us, the light reaches our eyes almost instantly, so we see them in the present moment. But when we look at faraway stars, we are seeing them as they were long ago. In this sense, studying the sky is a way of peeping into the deep past — the same deep past in which life first appeared.
Birth of the Universe and the Earth
The origin of life is considered a unique event in the history of the universe. The universe is unimaginably vast, and against its size the Earth is almost only a speck. Scientists estimate the universe to be about 13.8 billion years old. It is made of huge clusters of galaxies, and each galaxy contains stars along with clouds of gas and dust.
The Big Bang theory attempts to explain how the universe began. It proposes a single, enormous explosion — an event impossible to picture in ordinary physical terms. After this explosion the universe expanded, and as it expanded it cooled down. As temperatures fell, the gases hydrogen and helium formed. Under the pull of gravity these gases condensed to form the galaxies of the present-day universe.
Within the solar system of our Milky Way galaxy, the Earth is thought to have formed about 4.5 billion years ago. The early Earth had no atmosphere like ours today. Instead, its surface was covered by water vapour, methane (\(CH_4\)), carbon dioxide (\(CO_2\)) and ammonia (\(NH_3\)) released from the molten, semi-liquid mass of the young planet.
Ultraviolet (UV) rays from the Sun then broke up water into hydrogen and oxygen. We can represent this splitting simply as:
\[2H_2O \xrightarrow{\text{UV}} 2H_2 + O_2\]
The lighter hydrogen gas (\(H_2\)) escaped into space, while oxygen combined with ammonia and methane to form water, carbon dioxide and other compounds. Over time the ozone layer formed. As the Earth cooled further, the water vapour condensed and fell as rain, filling all the depressions on the surface to form the oceans. Life appeared about 500 million years after the Earth formed — that is, roughly four billion years ago.
The sequence of these grand events, from the Big Bang to the first appearance of life, is summarised in FC 6.1.
Flowchart
FC 6.1 – Origin sequence: Big Bang (~13.8 billion yrs ago) → universe expands and cools → hydrogen and helium form → gases condense under gravity → galaxies form → Earth forms (~4.5 billion yrs ago) → molten Earth releases water vapour, CH4, CO2, NH3 → UV splits water, H2 escapes, ozone layer forms → Earth cools, rain forms oceans → life appears (~4 billion yrs ago)
Did Life Come From Outer Space?
Some scientists have wondered whether life did not begin on Earth at all, but arrived from somewhere else. Early Greek thinkers imagined that tiny units of life, called spores, were carried between planets, including Earth. This idea — that life came from space — is called panspermia, and it remains a favourite notion for some astronomers even today.
From Non-living to Living: Competing Ideas
For a long time, many people believed that life could arise directly out of decaying and rotting matter such as straw or mud. This was the theory of spontaneous generation — the notion that living things spring up on their own from non-living material.
Careful experiments finally dismissed this idea. Louis Pasteur showed, through controlled experiments, that life comes only from pre-existing life. In flasks that had been sterilised beforehand, no new life appeared from killed yeast; but in a flask left open to the air, new living organisms did appear. Spontaneous generation was thus rejected once and for all.
Pasteur’s work, however, left one big question unanswered: if life only comes from earlier life, then how did the very first life form ever appear?
Chemical Evolution: The Oparin–Haldane Idea
An answer to Pasteur’s unanswered question was proposed by Oparin of Russia and Haldane of England. They suggested that the first form of life could have come from pre-existing non-living organic molecules — such as RNA and proteins — and that the appearance of life was preceded by chemical evolution. Chemical evolution means the gradual formation of diverse organic molecules from simpler inorganic substances.
The conditions on the early Earth were very different from today. There was high temperature, frequent volcanic storms, and a reducing atmosphere rich in gases such as methane (\(CH_4\)) and ammonia (\(NH_3\)), with almost no free oxygen.
Miller’s Experiment
Could such chemistry really happen? In 1953, an American scientist named S. L. Miller recreated the conditions of the early Earth on a laboratory scale, as shown in Fig. 6.1.
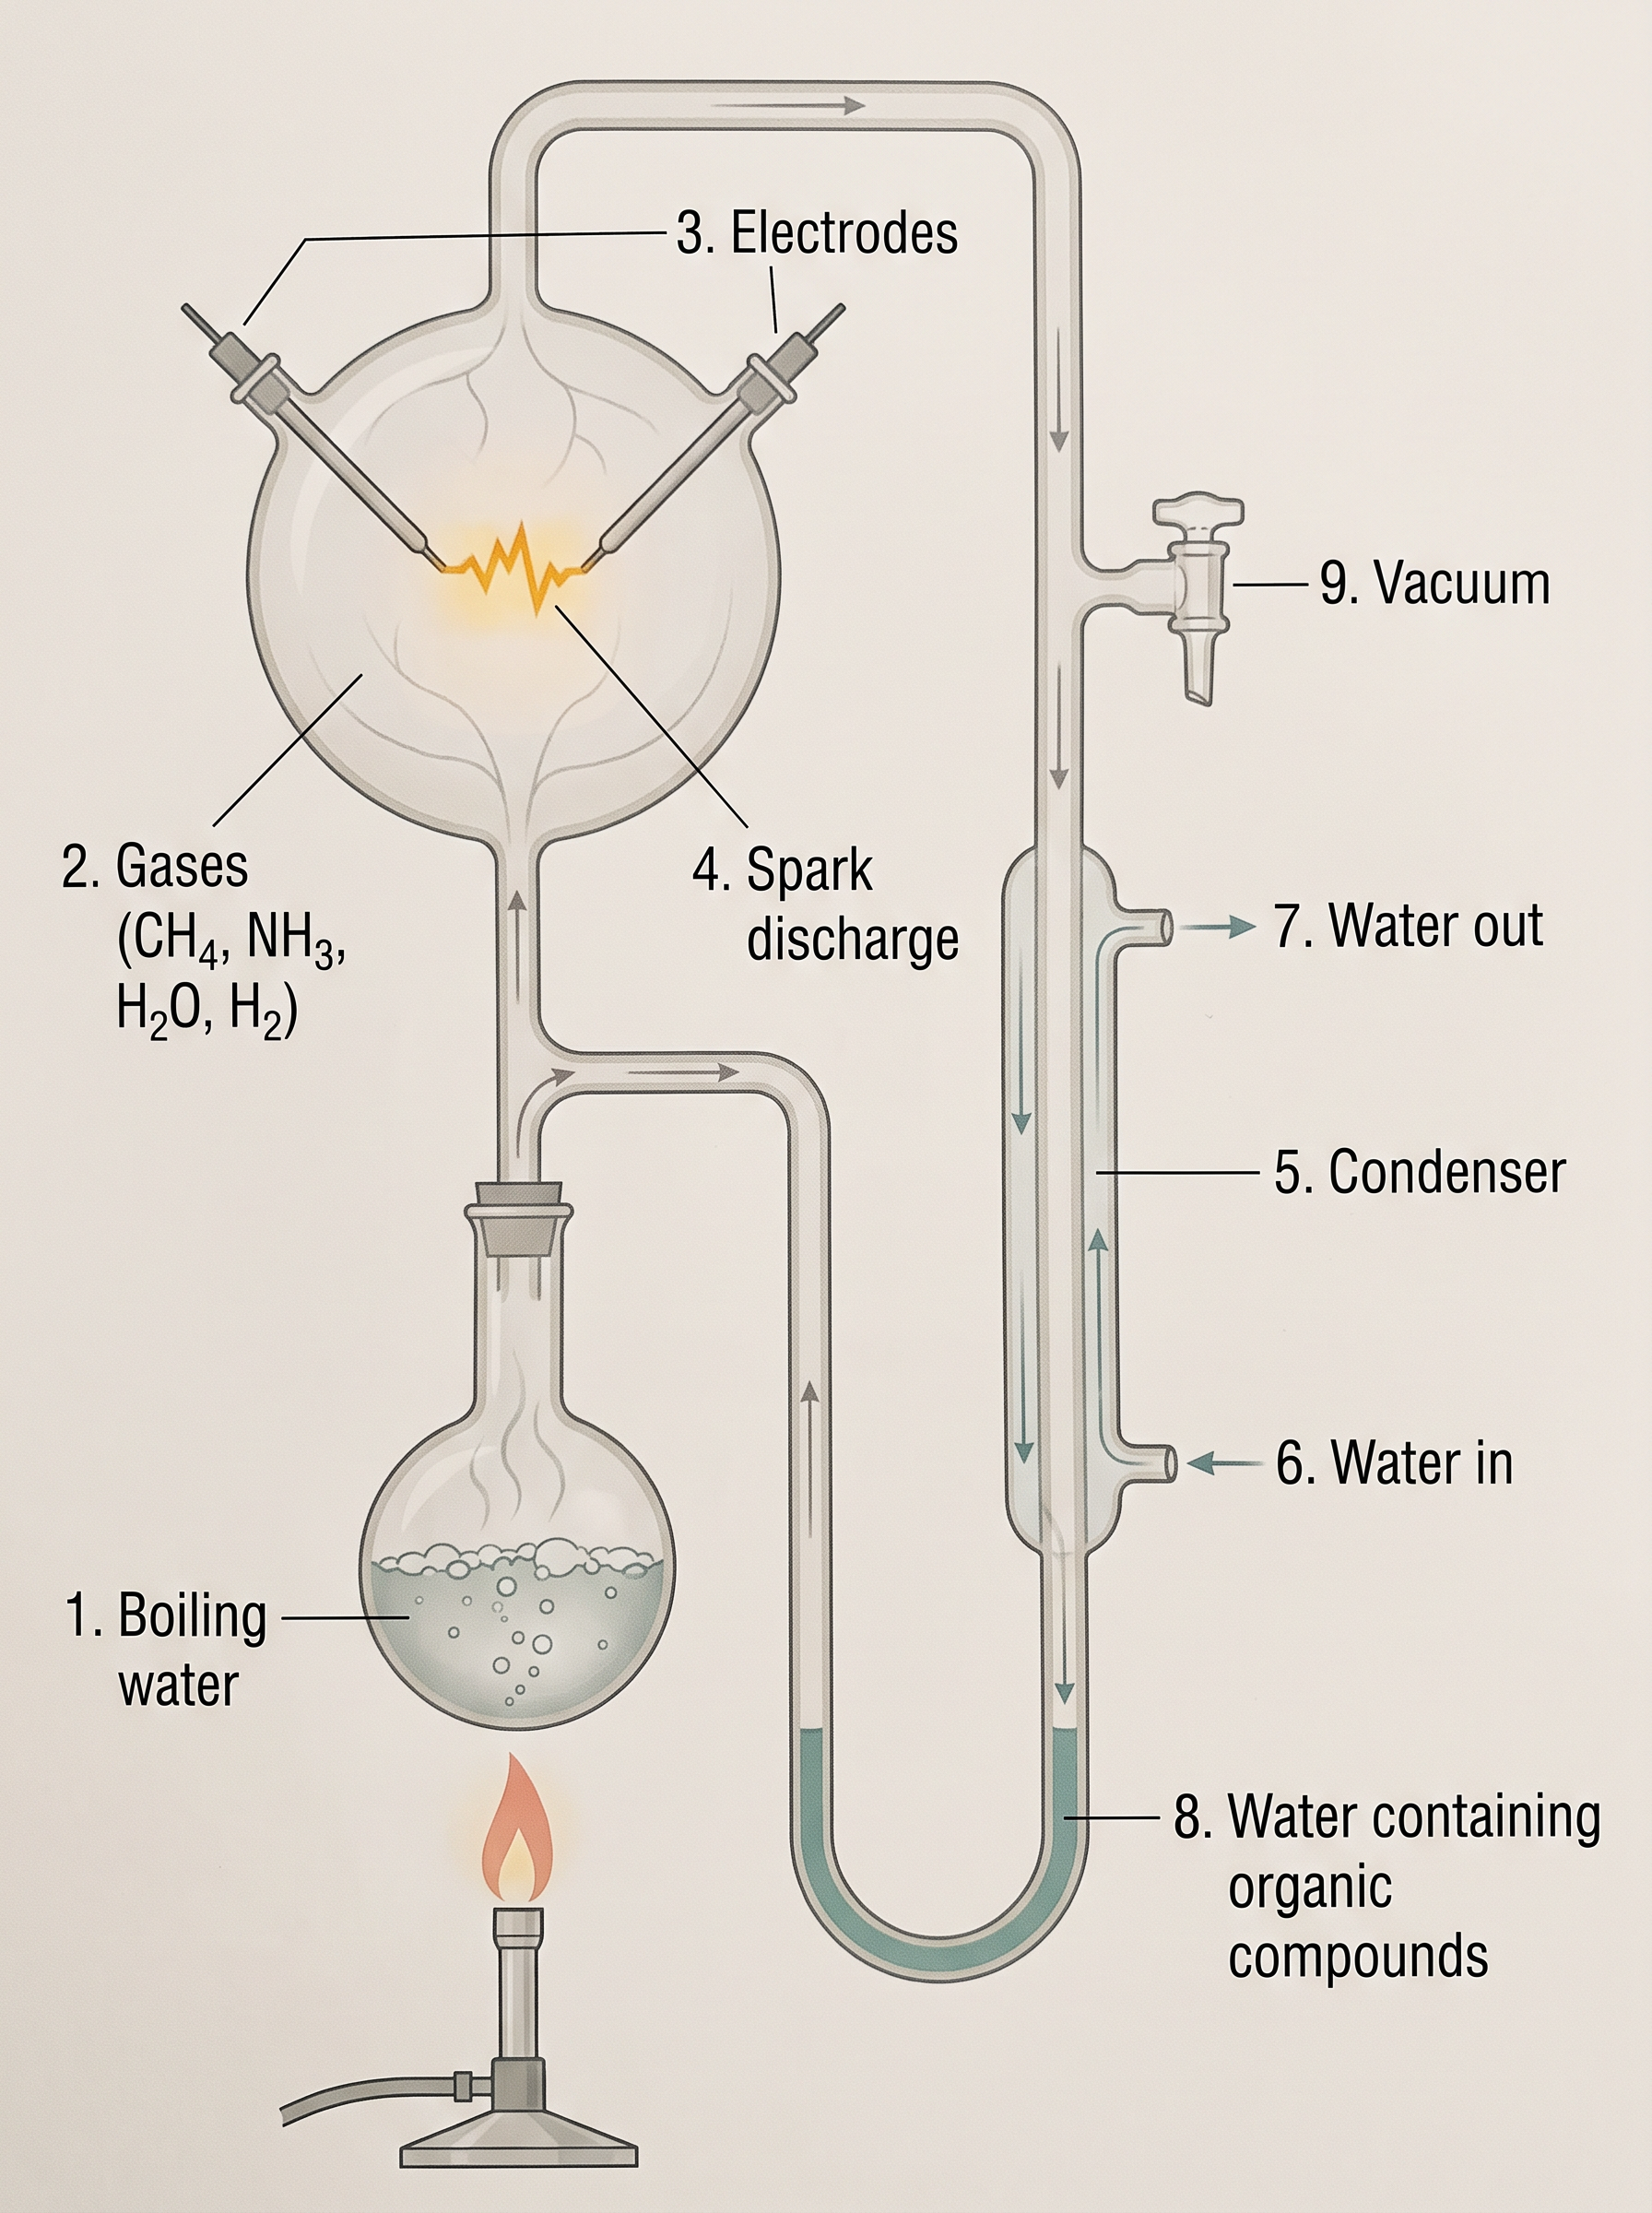
Fig. 6.1 – Miller’s spark-discharge apparatus.
Miller passed an electric discharge (to mimic lightning) through a closed flask containing methane (\(CH_4\)), hydrogen (\(H_2\)), ammonia (\(NH_3\)) and water vapour at \(800^\circ C\). After running the experiment, he observed the formation of amino acids — the building blocks of proteins.
In similar experiments, other scientists observed the formation of sugars, nitrogen bases, pigments and fats. Even the analysis of meteorite material revealed similar compounds, suggesting that such chemical processes are also occurring elsewhere in space. With this limited but striking evidence, the first part of the conjectured story — chemical evolution — became more or less accepted.
The First Life Forms
We still have no clear idea of exactly how the first self-replicating, metabolising capsule of life arose. The first non-cellular forms of life could have originated about 3 billion years ago. These would have been giant molecules — such as RNA, proteins and polysaccharides — and these capsules were perhaps able to reproduce their own molecules.
The first cellular form of life did not appear until about 2000 million years ago. These earliest cells were probably single-celled, and all life at this stage existed only in water. This version of biogenesis — the idea that the first form of life arose slowly, through natural evolutionary forces, from non-living molecules — is accepted by most scientists today.
Once the first cells had formed, a new and fascinating question opened up: how could these simple cellular forms of life have evolved into the enormous, complex biodiversity we see around us today? That is the story explored in the sections that follow.
6.2 Evolution of Life Forms – A Theory
Where did the great variety of living things come from? Long before modern biology, people already had answers to this question. The most influential of these was the idea of special creation, and it was only in the nineteenth century that a very different explanation began to take its place.
The Idea of Special Creation
Conventional religious literature described the origin of life through the theory of special creation. This theory carries three main ideas, or connotations.
First, that all the living organisms — every species or type — that we see today were created exactly as they are now. Second, that the diversity of life has always been the same since the moment of creation, and will remain the same in the future. Third, that the Earth itself is only about 4000 years old.
All three of these ideas were strongly challenged during the nineteenth century, as scientists began to gather evidence pointing to a very different picture of life’s history.
Darwin and the Voyage of the Beagle
The most powerful challenge came from Charles Darwin. His conclusions grew out of careful observations made during a long sea voyage around the world aboard a sailing ship called H.M.S. Beagle.
Darwin concluded that existing living forms share similarities — to varying degrees — not only with one another, but also with life forms that existed millions of years ago. Many of those ancient forms no longer exist. Over the long history of the Earth, there had been repeated extinctions of some life forms, even as new forms arose at different periods. In other words, life has undergone gradual evolution.
Variation, Fitness and Natural Selection
Darwin observed that any population has a built-in variation in its characteristics — no two individuals are exactly alike. Some of these characteristics allow certain individuals to survive better under natural conditions such as climate, availability of food, and other physical factors. Those better-suited individuals out-reproduce the others that are less well-endowed to survive.
Darwin described this success using the word fitness. Importantly, fitness for Darwin refers ultimately and only to reproductive fitness — that is, how many surviving offspring an individual leaves behind, not merely its physical strength.
So, individuals that are better fit in a given environment leave more progeny, survive in greater numbers, and are effectively “chosen” by nature. Darwin called this process natural selection and proposed it as the mechanism of evolution. The overall logic is shown in FC 6.2.
Flowchart
FC 6.2 – Logic of natural selection: population has built-in variation → some variants survive better in the environment → these fitter individuals leave more surviving offspring → their favourable traits become more common in the next generation → over many generations population characteristics change → new forms of life appear
It is worth remembering that Darwin was not entirely alone in this insight. Alfred Wallace, a naturalist working in the Malay Archipelago, arrived at very similar conclusions at around the same time.
Common Ancestry and an Ancient Earth
In due course of time, new types of organisms become recognisable. All existing life forms share similarities with one another, and share common ancestors. These ancestors, however, lived at different points in the Earth’s long history — spread across its many epochs, periods and eras.
The geological history of the Earth closely matches its biological history: as the planet’s rocks and conditions changed over time, so did its life forms. A common and reasonable conclusion drawn from all this is that the Earth is very old — not just thousands of years, as once believed, but billions of years old.
6.3 What are the Evidences for Evolution?
If evolution really happened, we should be able to find its fingerprints in the living and non-living world around us. In fact, evidence that evolution has taken place on Earth comes from many different quarters — from rocks, from embryos, from body structures, from molecules, and even from changes we can watch happening today.
Evidence from Fossils (Palaeontology)
Fossils are the remains of the hard parts of ancient life-forms, preserved in rocks. To understand how they help us, we need to think about how rocks form. Over long periods, layers of sediment settle one on top of another, and a cross-section of the Earth’s crust shows these sediments stacked in order — the oldest at the bottom, the youngest at the top.
Rock sediments of different ages contain fossils of different life-forms, which probably died during the formation of that particular layer. Some of these fossils look similar to organisms alive today, while others represent extinct organisms such as the dinosaurs, as shown in Fig. 6.2.
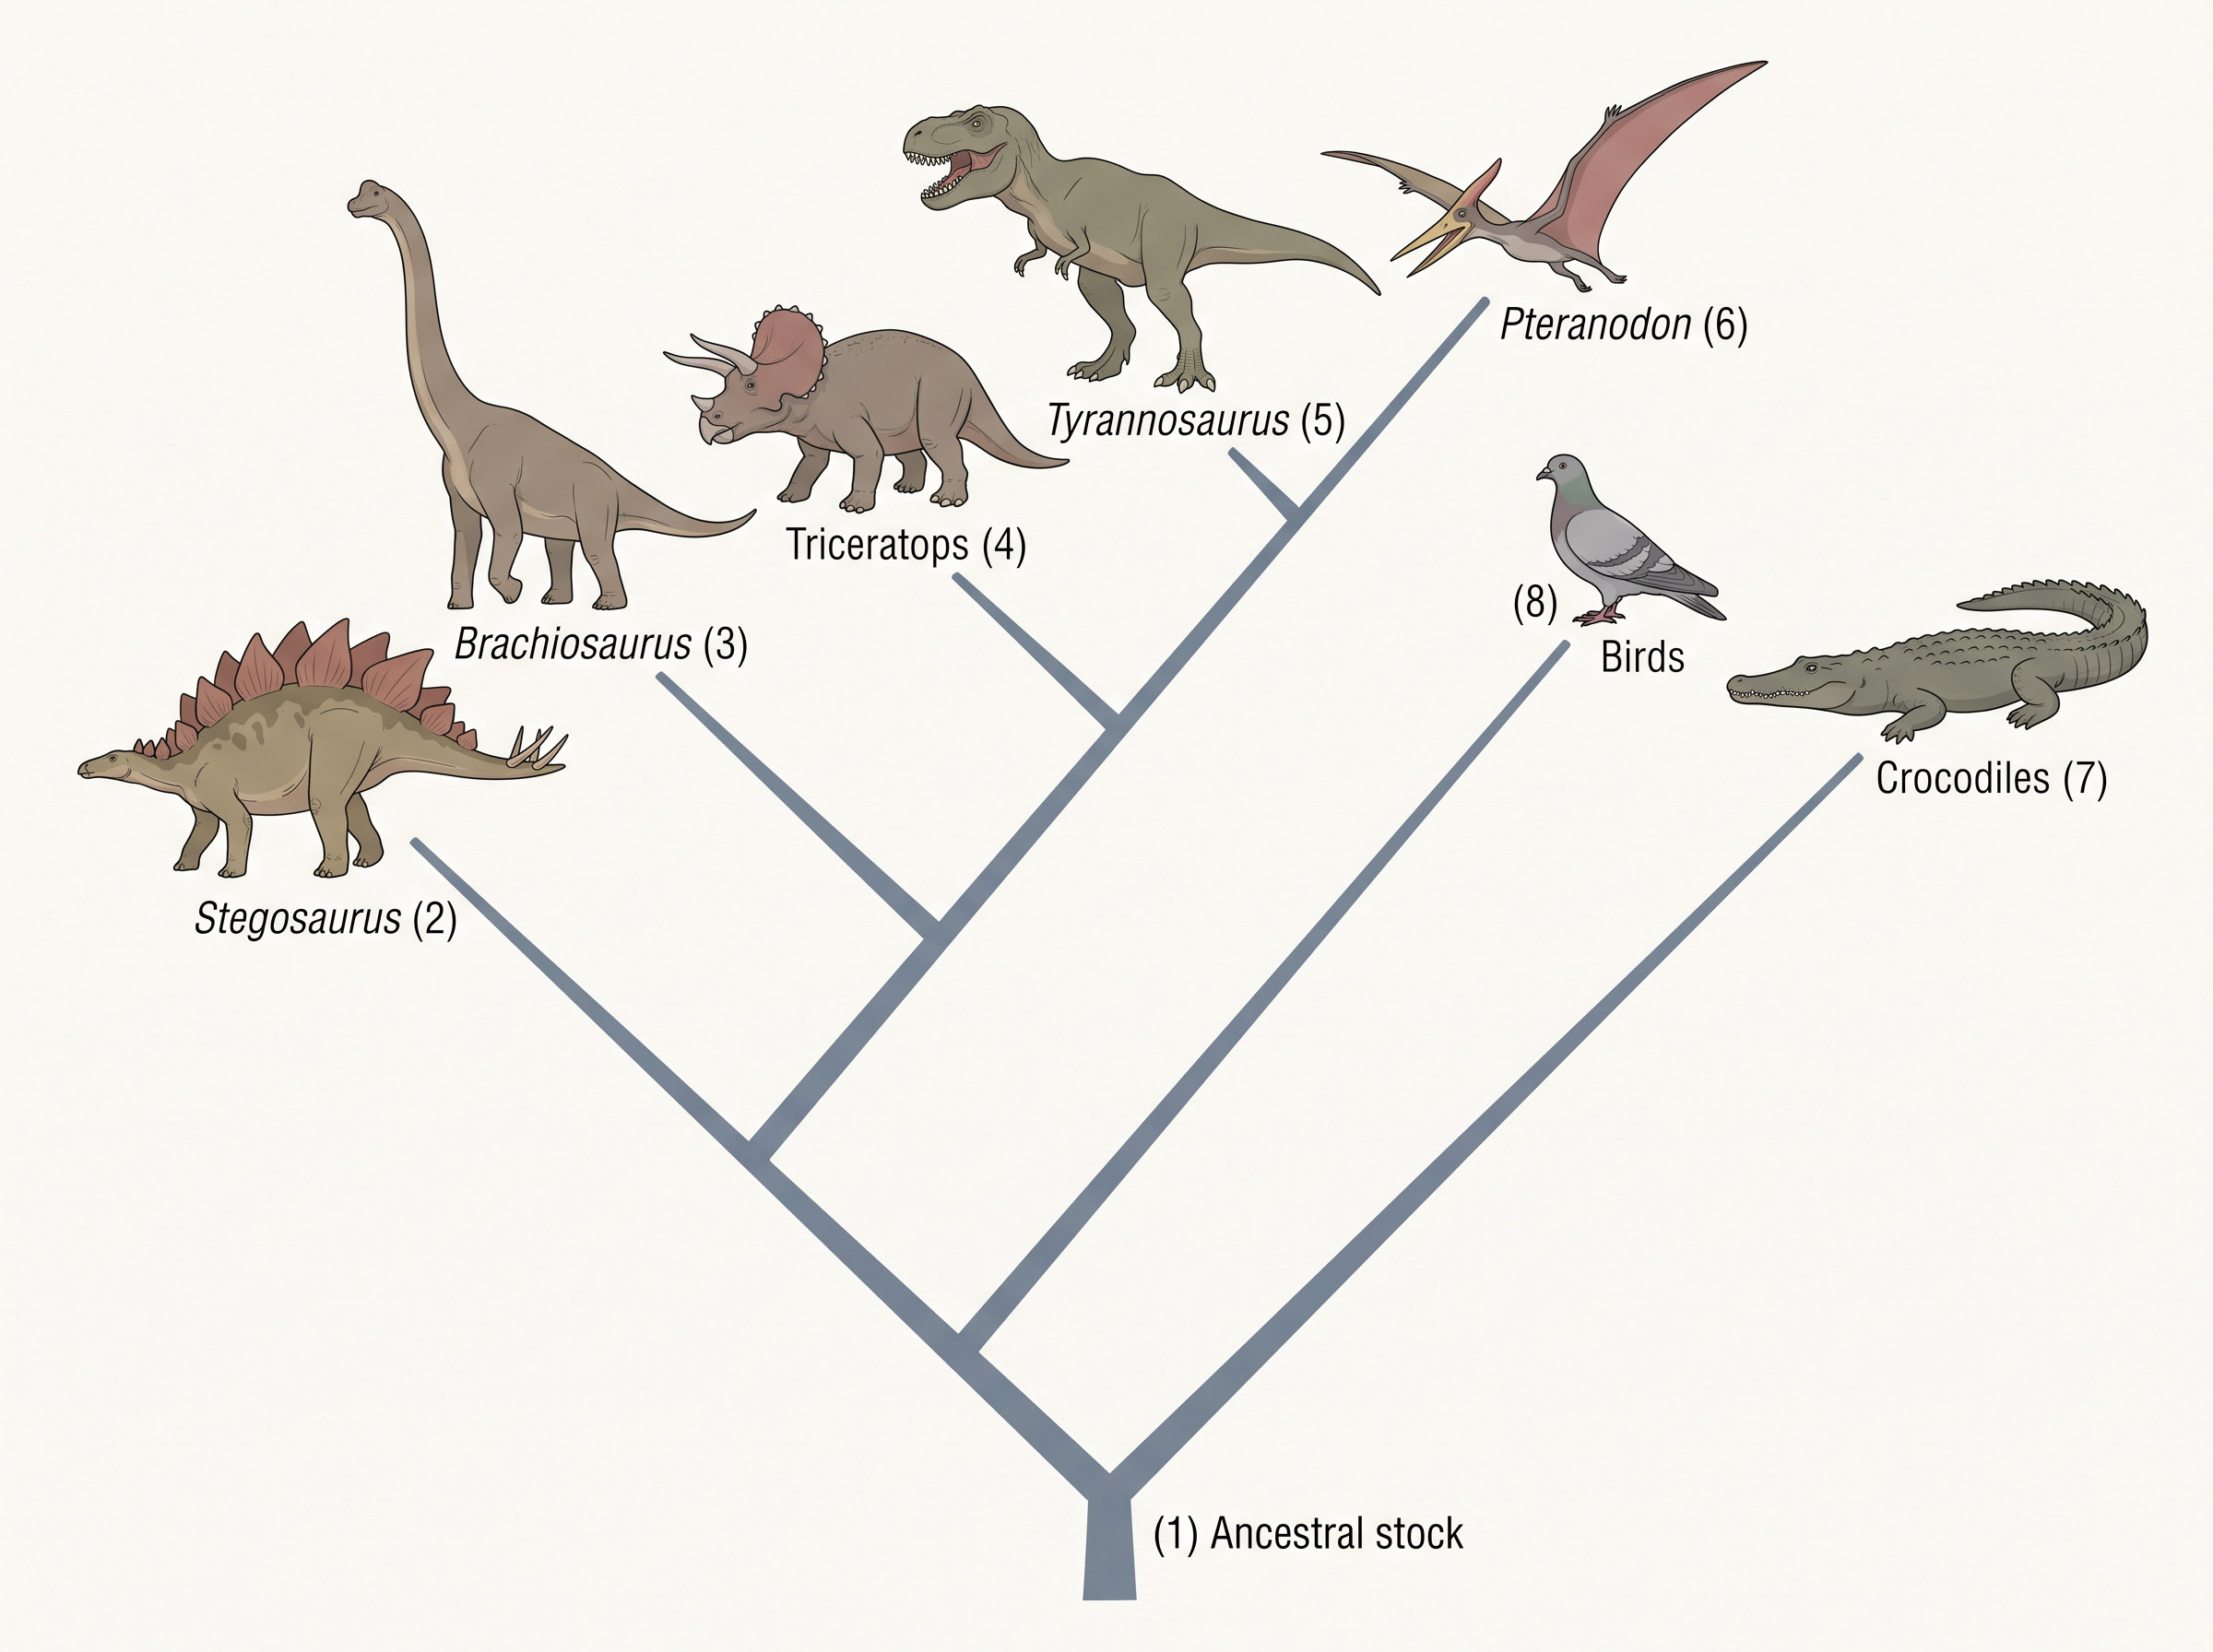
Fig. 6.2 – Family tree of dinosaurs and their living relatives.
By studying which fossils appear in which sedimentary layers, scientists can work out the geological period in which each life-form existed. Such studies show that life-forms have varied over time, and that certain life-forms are restricted to certain geological time-spans. This tells us that new forms of life have arisen at different times in the Earth’s history. All of this together is called palaeontological evidence.
But how do we know the age of a fossil? This is done using radioactive dating. Certain elements in the rock decay at a known, fixed rate, so by measuring how much of a radioactive element remains, scientists can estimate how long ago the fossil was buried.
Evidence from Embryology
Another line of support once came from embryology — the study of embryos. It was proposed by Ernst Haeckel, based on the observation that certain features appear during the embryonic stage of all vertebrates but are absent in the adult.
For example, the embryos of all vertebrates, including human beings, develop a row of vestigial gill slits just behind the head. In fish these gill slits become functional organs, but in other adult vertebrates they are not found, as illustrated in Fig. 6.3c.
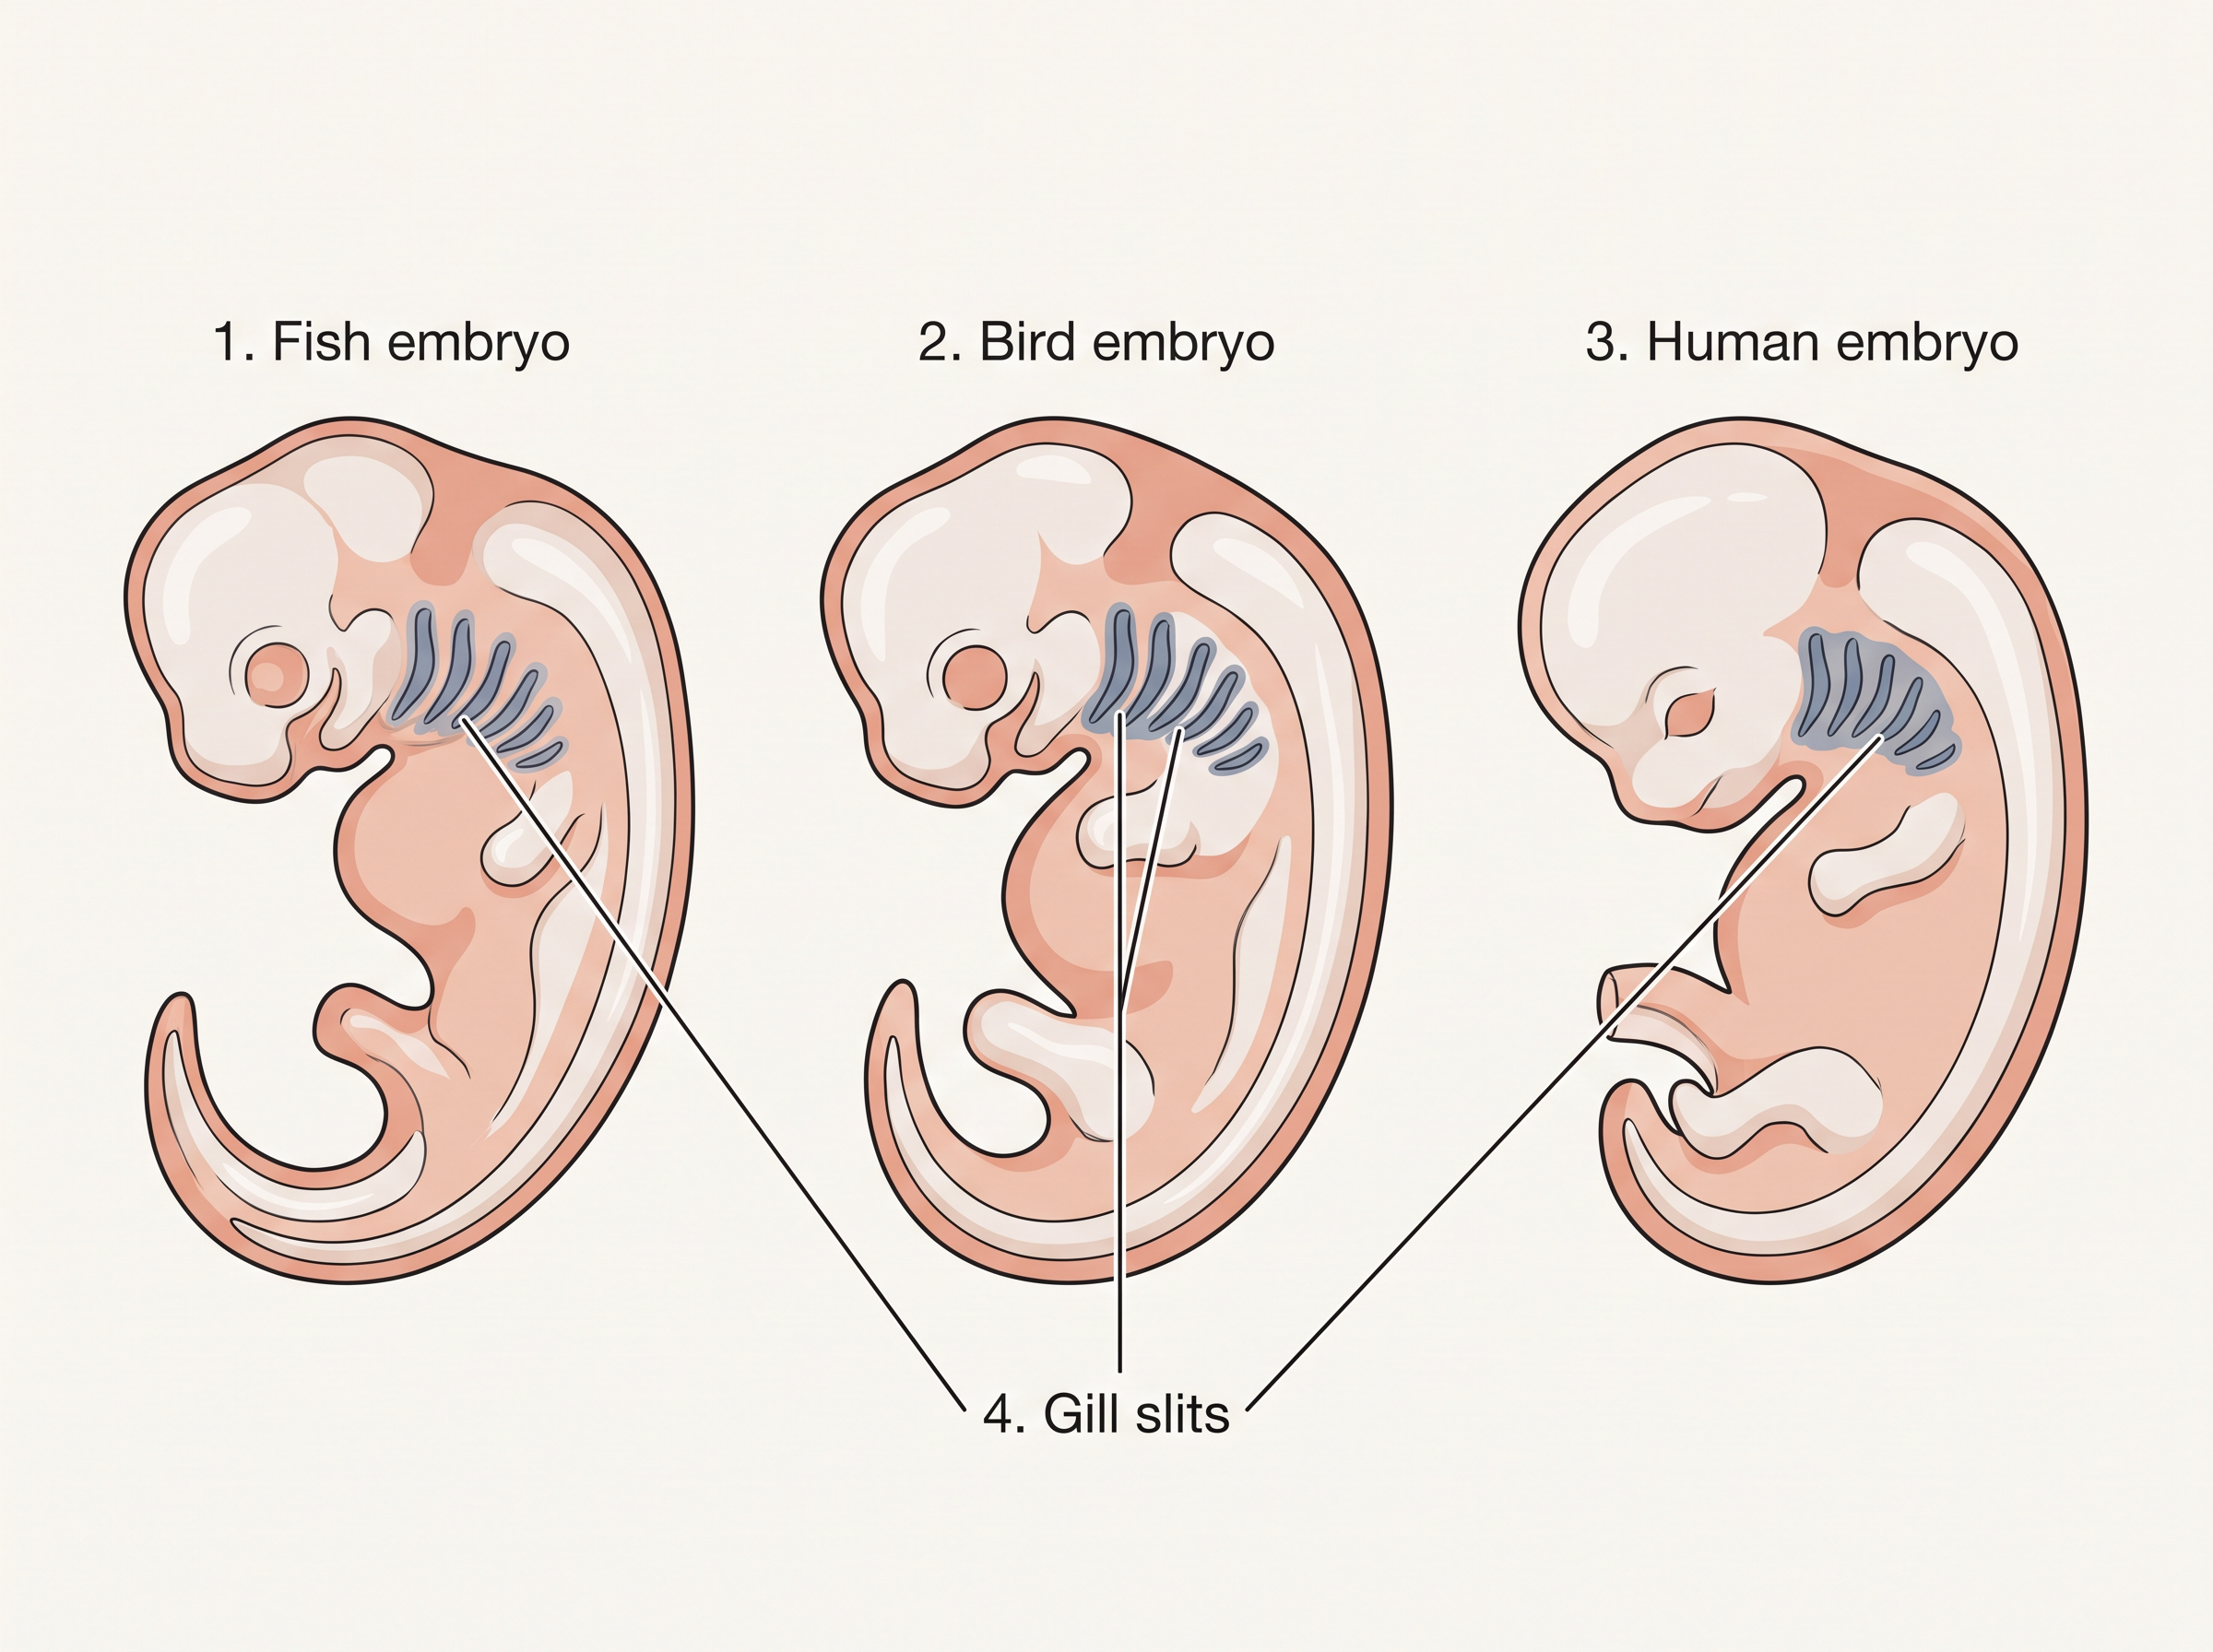
Fig. 6.3c – Vestigial gill slits in vertebrate embryos.
However, this embryological proposal was later disapproved after careful study by Karl Ernst von Baer. He noted that embryos never pass through the adult stages of other animals — an embryo does not, for instance, become an adult fish on its way to becoming a human.
Evidence from Comparative Anatomy and Morphology
Comparative anatomy and morphology look at the similarities and differences among organisms living today and those that existed long ago. Such comparisons can tell us whether different organisms shared a common ancestor or not.
Consider the forelimbs of whales, bats, the cheetah and humans — all of which are mammals. Although these forelimbs perform very different functions (swimming, flying, running, grasping), they share the same basic anatomical plan, as seen in Fig. 6.4b. Each contains the same set of bones: humerus, radius, ulna, carpals, metacarpals and phalanges.
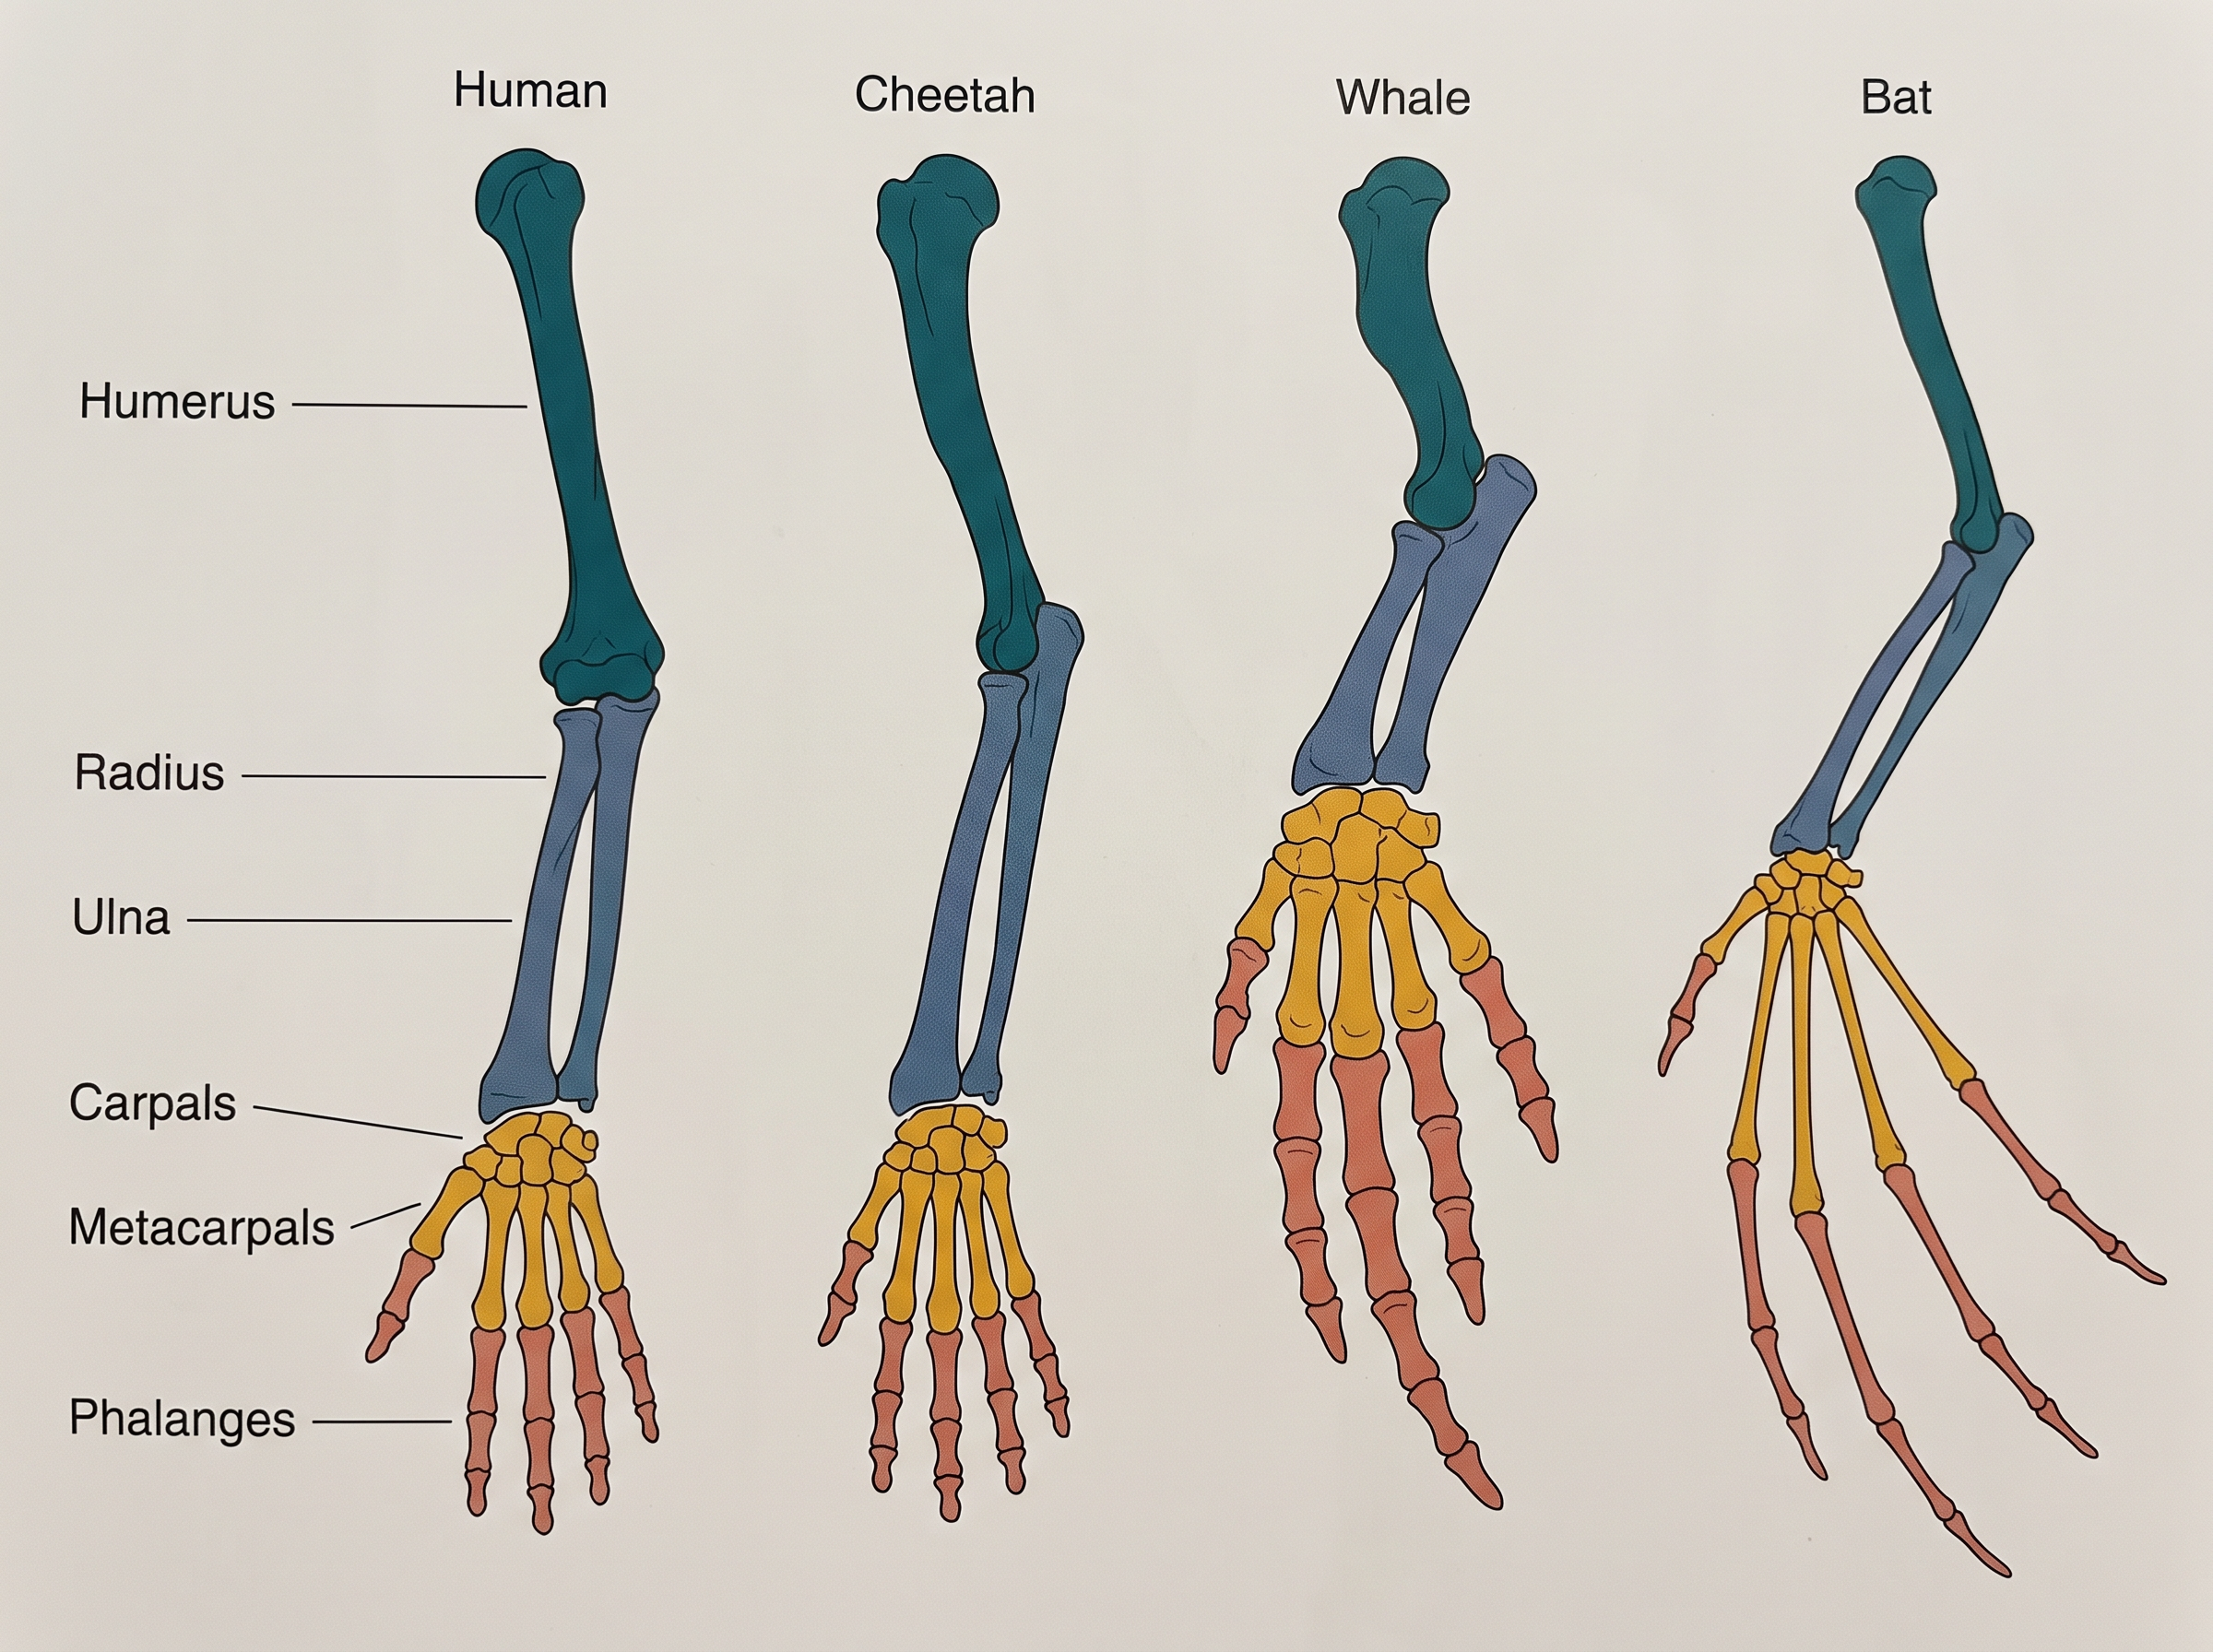
Fig. 6.4b – Homologous forelimbs of mammals.
Here, the same underlying structure has developed along different directions because each animal became adapted to a different need. This is called divergent evolution, and structures that arise this way are said to be homologous. Homology indicates common ancestry. Other examples of homologous organs are the hearts and brains of different vertebrates.
Homology is not limited to animals. In plants, the thorn of Bougainvillea and the tendril of Cucurbita are homologous — both are modified from the same basic structure but serve different purposes, as shown in Fig. 6.5a.
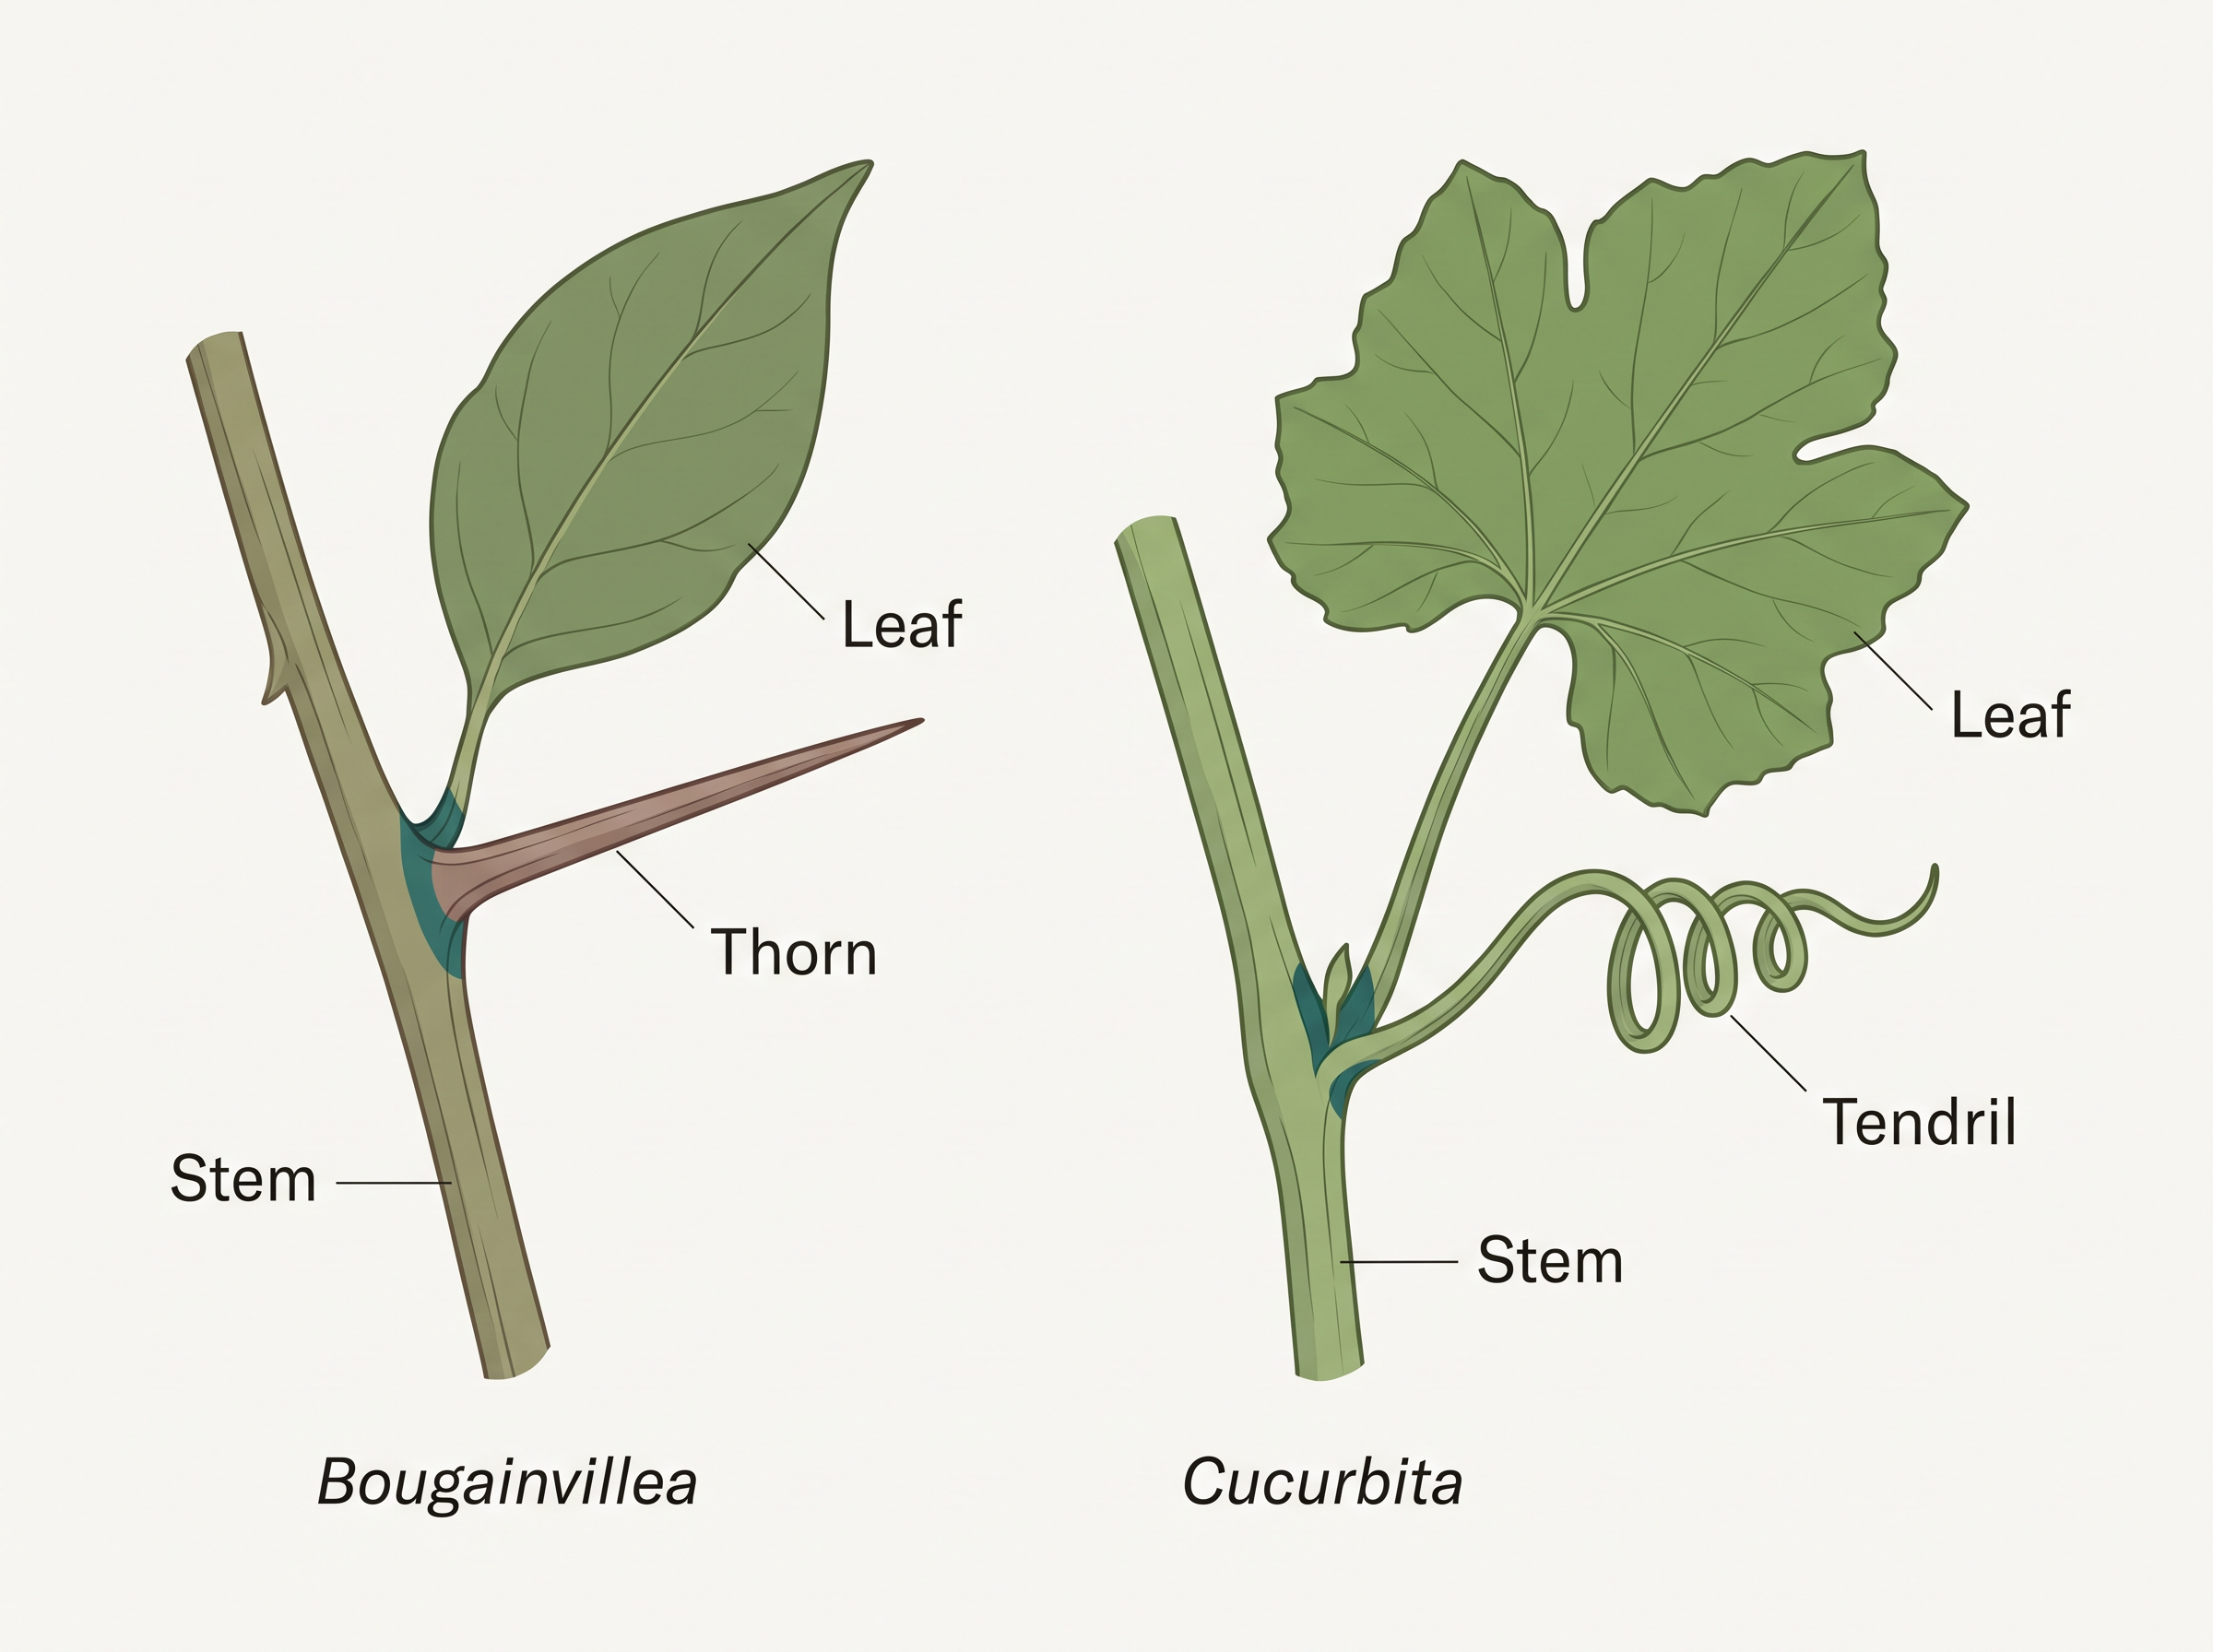
Fig. 6.5a – Homologous structures in plants.
Analogy refers to exactly the opposite situation. The wings of a butterfly and the wings of a bird look alike and perform a similar function (flight), yet they are not anatomically similar structures at all. Such analogous structures are the result of convergent evolution — different structures evolving toward the same function and thereby coming to resemble one another.
Other examples of analogy include the eye of the octopus and the eye of mammals, and the flippers of penguins and dolphins. In each case, it is the similar habitat that has led to the selection of similar adaptive features in unrelated groups of organisms, serving the same function. In plants, the sweet potato (a modified root) and the potato (a modified stem) look and function similarly and are another example of analogy.
Evidence from Molecular Biology
Evidence for common ancestry is also written into the molecules of life. When diverse organisms carry out the same function using very similar proteins and genes, this points to shared ancestry. These biochemical similarities support the same conclusion as structural similarities: that organisms which resemble one another at the molecular level share a common evolutionary origin.
Evidence from Artificial Selection
Humans themselves have provided a striking demonstration of how selection can reshape living things. For agriculture, horticulture, sport and security, people have carefully bred selected plants and animals, and have domesticated many wild species and crops.
This intensive breeding has produced many different breeds — for example, the enormous variety of dog breeds — that differ greatly from one another yet still belong to the same group. The argument follows naturally: if human beings could create so many new breeds within just a few hundred years, could nature not have brought about far greater change over millions of years?
Evidence from Natural Selection: Moths and Industrial Melanism
One of the most famous observations supporting evolution by natural selection comes from England. In a collection of moths made in the 1850s, before industrialisation, there were more white-winged moths on trees than dark-winged, or melanised, moths. But in a collection made from the same area after industrialisation, in 1920, the situation had reversed — dark-winged moths were now more common.
The explanation offered was that predators spot a moth more easily against a contrasting background. During the post-industrial period, tree trunks became dark due to industrial smoke and soot. Against these dark trunks, white-winged moths stood out and were eaten by predators, while dark-winged (melanised) moths were camouflaged and survived, as shown in Fig. 6.6.
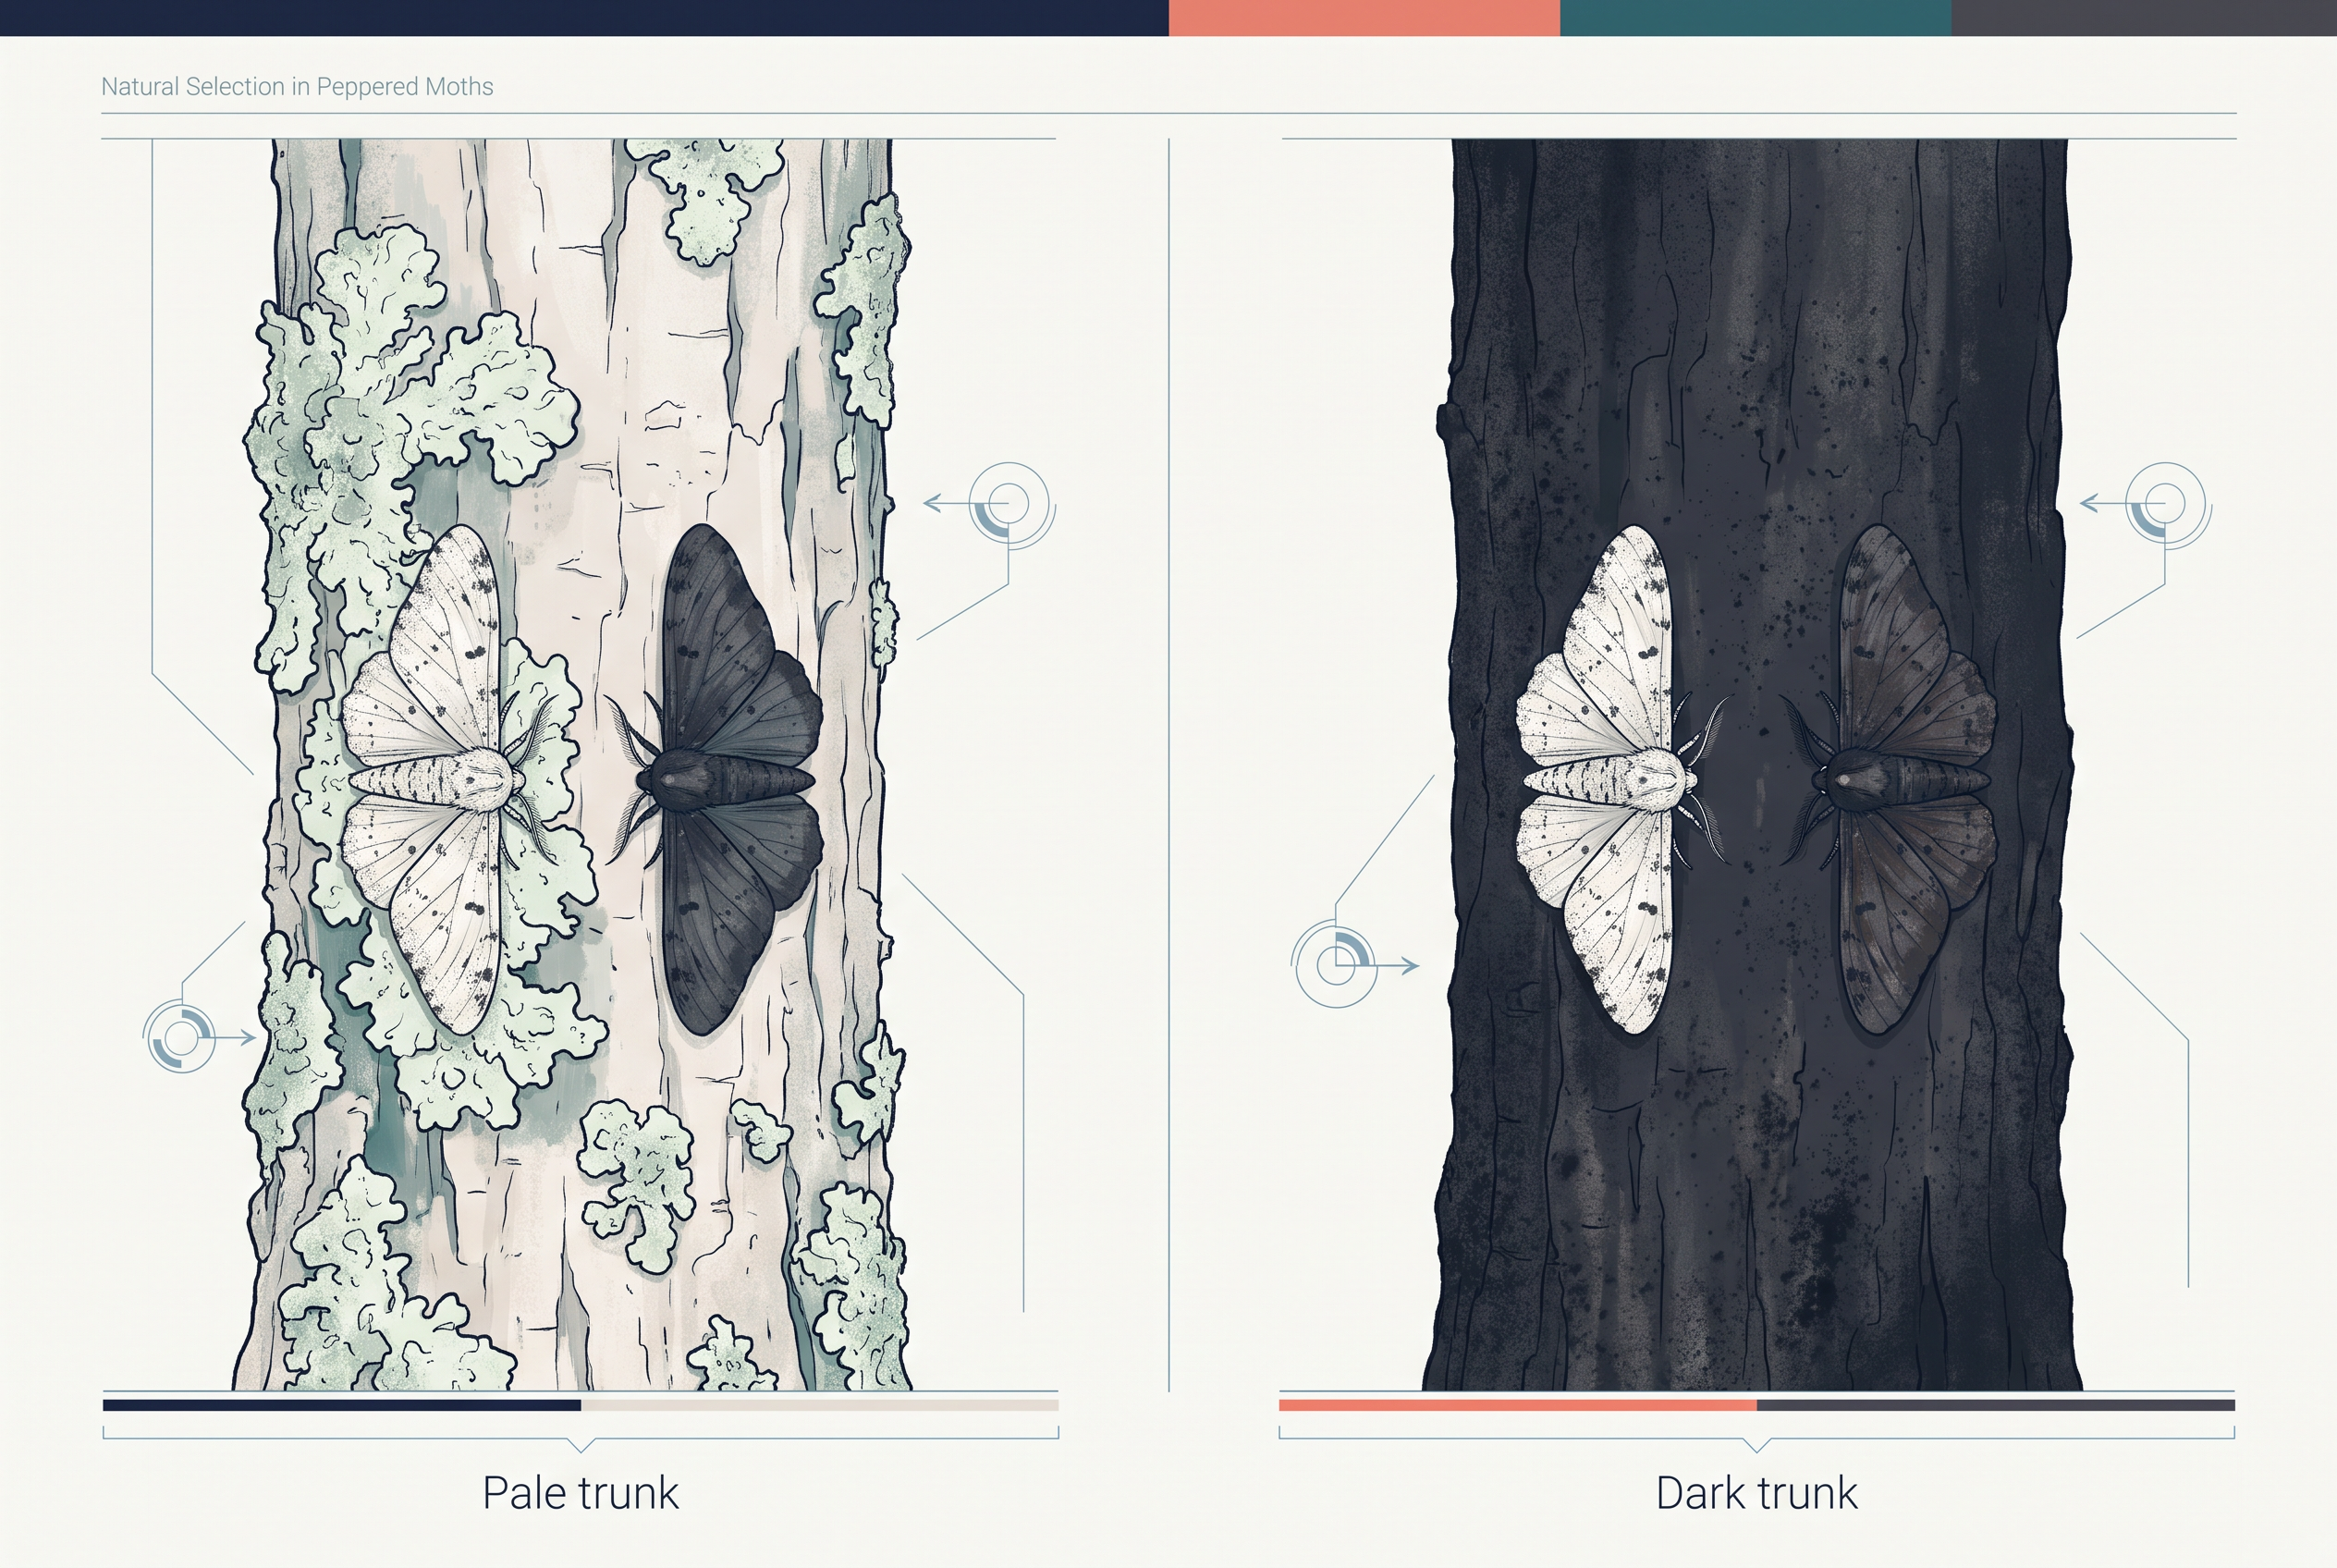
Fig. 6.6 – Industrial melanism in peppered moths.
Before industrialisation, a thick growth of almost white-coloured lichen covered the trees. Against this pale background the white-winged moth was well hidden, while the dark-coloured moths were picked out by predators. So in each period, the moths that could camouflage themselves — blend into the background — were the ones that survived.
This understanding is supported by another fact: in rural areas where industrialisation did not occur, the count of melanic (dark) moths remained low. In a mixed population, then, those that can better adapt to the surroundings survive and increase in number. Importantly, no variant is completely wiped out — the rarer form still persists.
Evolution by Anthropogenic Action
The same principle can be seen wherever human activity puts populations under sudden pressure. The excessive use of herbicides and pesticides has led, in a much shorter time, to the selection of resistant varieties of weeds and pests. The same is true of microbes against which we use antibiotics, and of drugs used against eukaryotic organisms or cells.
Because these organisms reproduce so rapidly, resistant forms appear within a timescale of months or years, not centuries. These are examples of evolution by anthropogenic (human-caused) action.
These observations also carry a deeper lesson: evolution is not a directed process in the sense of following a predetermined plan. It is a stochastic (chance-driven) process, based on chance events in nature and chance mutations in organisms. The environment simply selects among whatever variations happen to exist.
6.4 What is Adaptive Radiation?
Some of the most convincing evidence for evolution comes from what happens when a group of organisms reaches a new, isolated place with many empty habitats. Darwin himself witnessed a beautiful example of this during his travels.
Darwin’s Finches
During his journey, Darwin visited the Galapagos Islands, where he observed an amazing diversity of creatures. Of particular interest were small black birds, later called Darwin’s Finches, which greatly amazed him. He realised that there were many different varieties of these finches on the same island.
Darwin conjectured that all these varieties had evolved on the island itself, from a single starting stock. From the original seed-eating finches, many other forms with altered beaks arose, allowing some to become insectivorous (insect-eating) and vegetarian, as shown in Fig. 6.7.
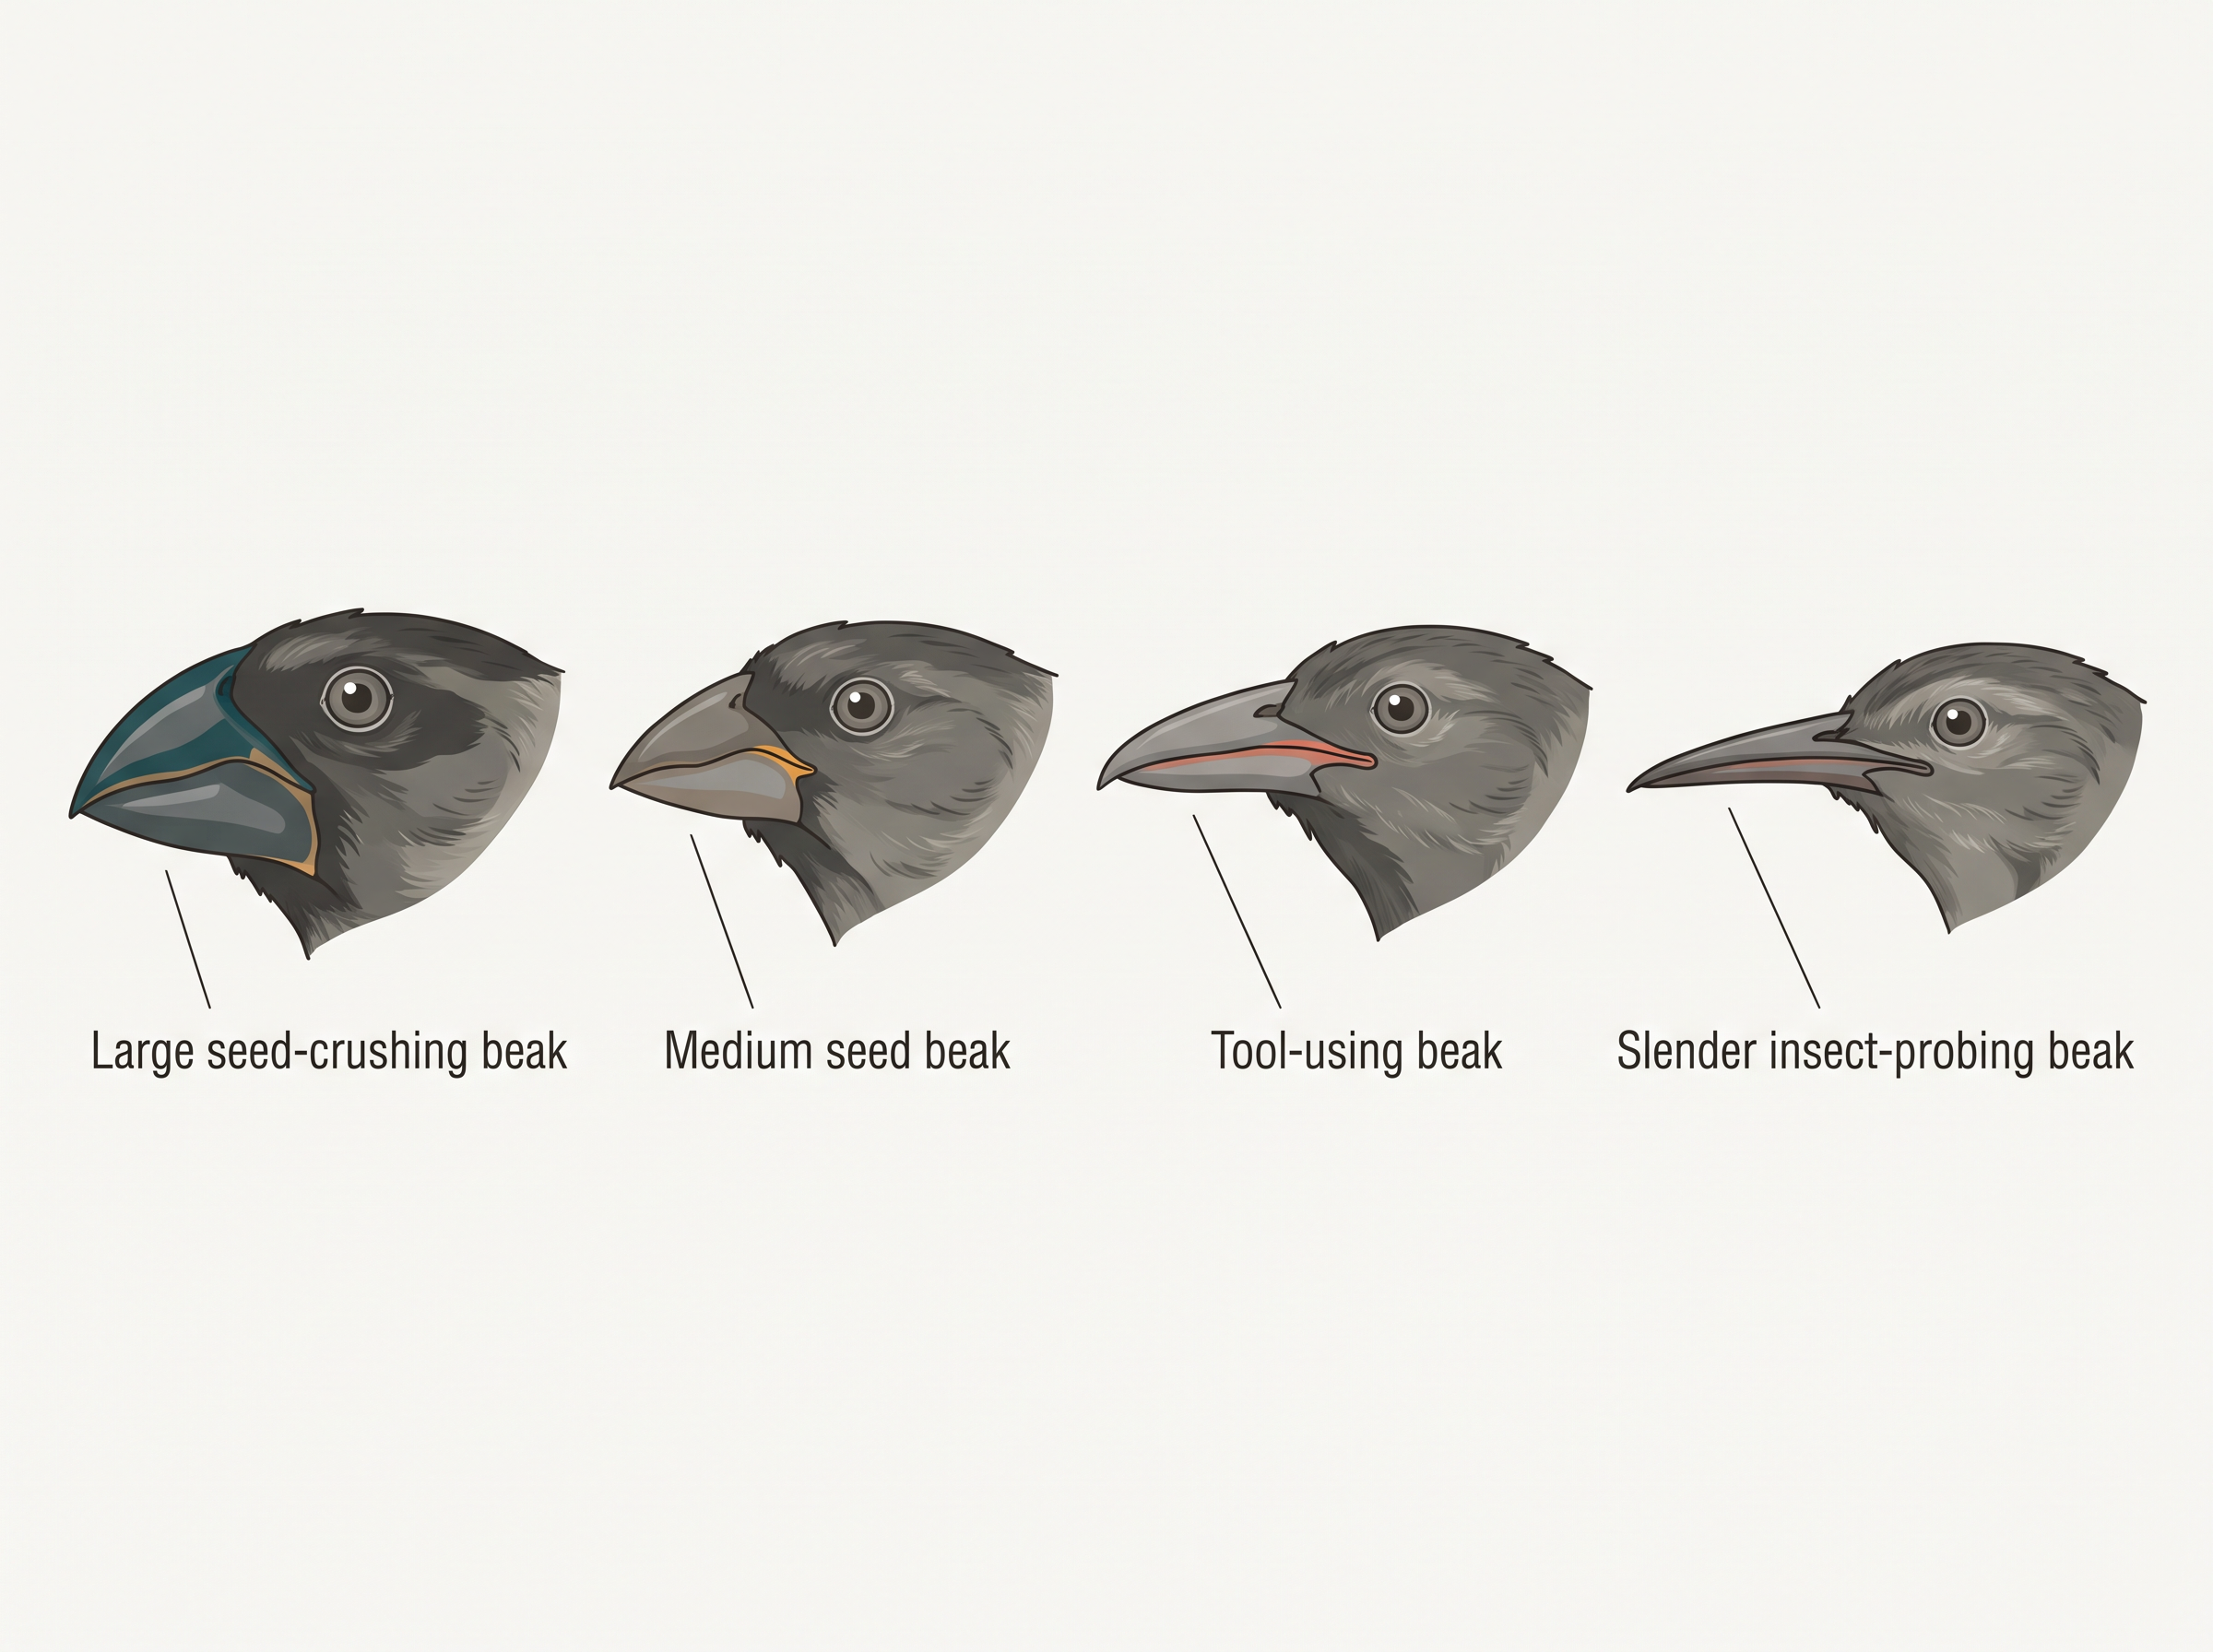
Fig. 6.7 – Beak variation in Darwin’s finches.
The beak is the key to this story. Each beak shape suits a particular kind of food, so a change in beak shape opens up a new way of life.
This process — where different species evolve in a given geographical area, starting from a single point and literally radiating out into other habitats — is called adaptive radiation. Darwin’s finches are one of the best examples of this phenomenon. The way one ancestral stock fans out into many forms is summarised in FC 6.3.
Flowchart
FC 6.3 – Adaptive radiation of finches: ancestral seed-eating finch reaches the islands → radiates into several forms → seed-eating finch (heavy beak) / insectivorous finch (slender beak) / vegetarian finch (adapted beak), each occupying a different habitat and food niche
Australian Marsupials
Another classic example of adaptive radiation is seen in the Australian marsupials — pouched mammals. A large number of marsupials, each different from the others, evolved from a single ancestral stock, but all within the isolated Australian island continent, as shown in Fig. 6.8.
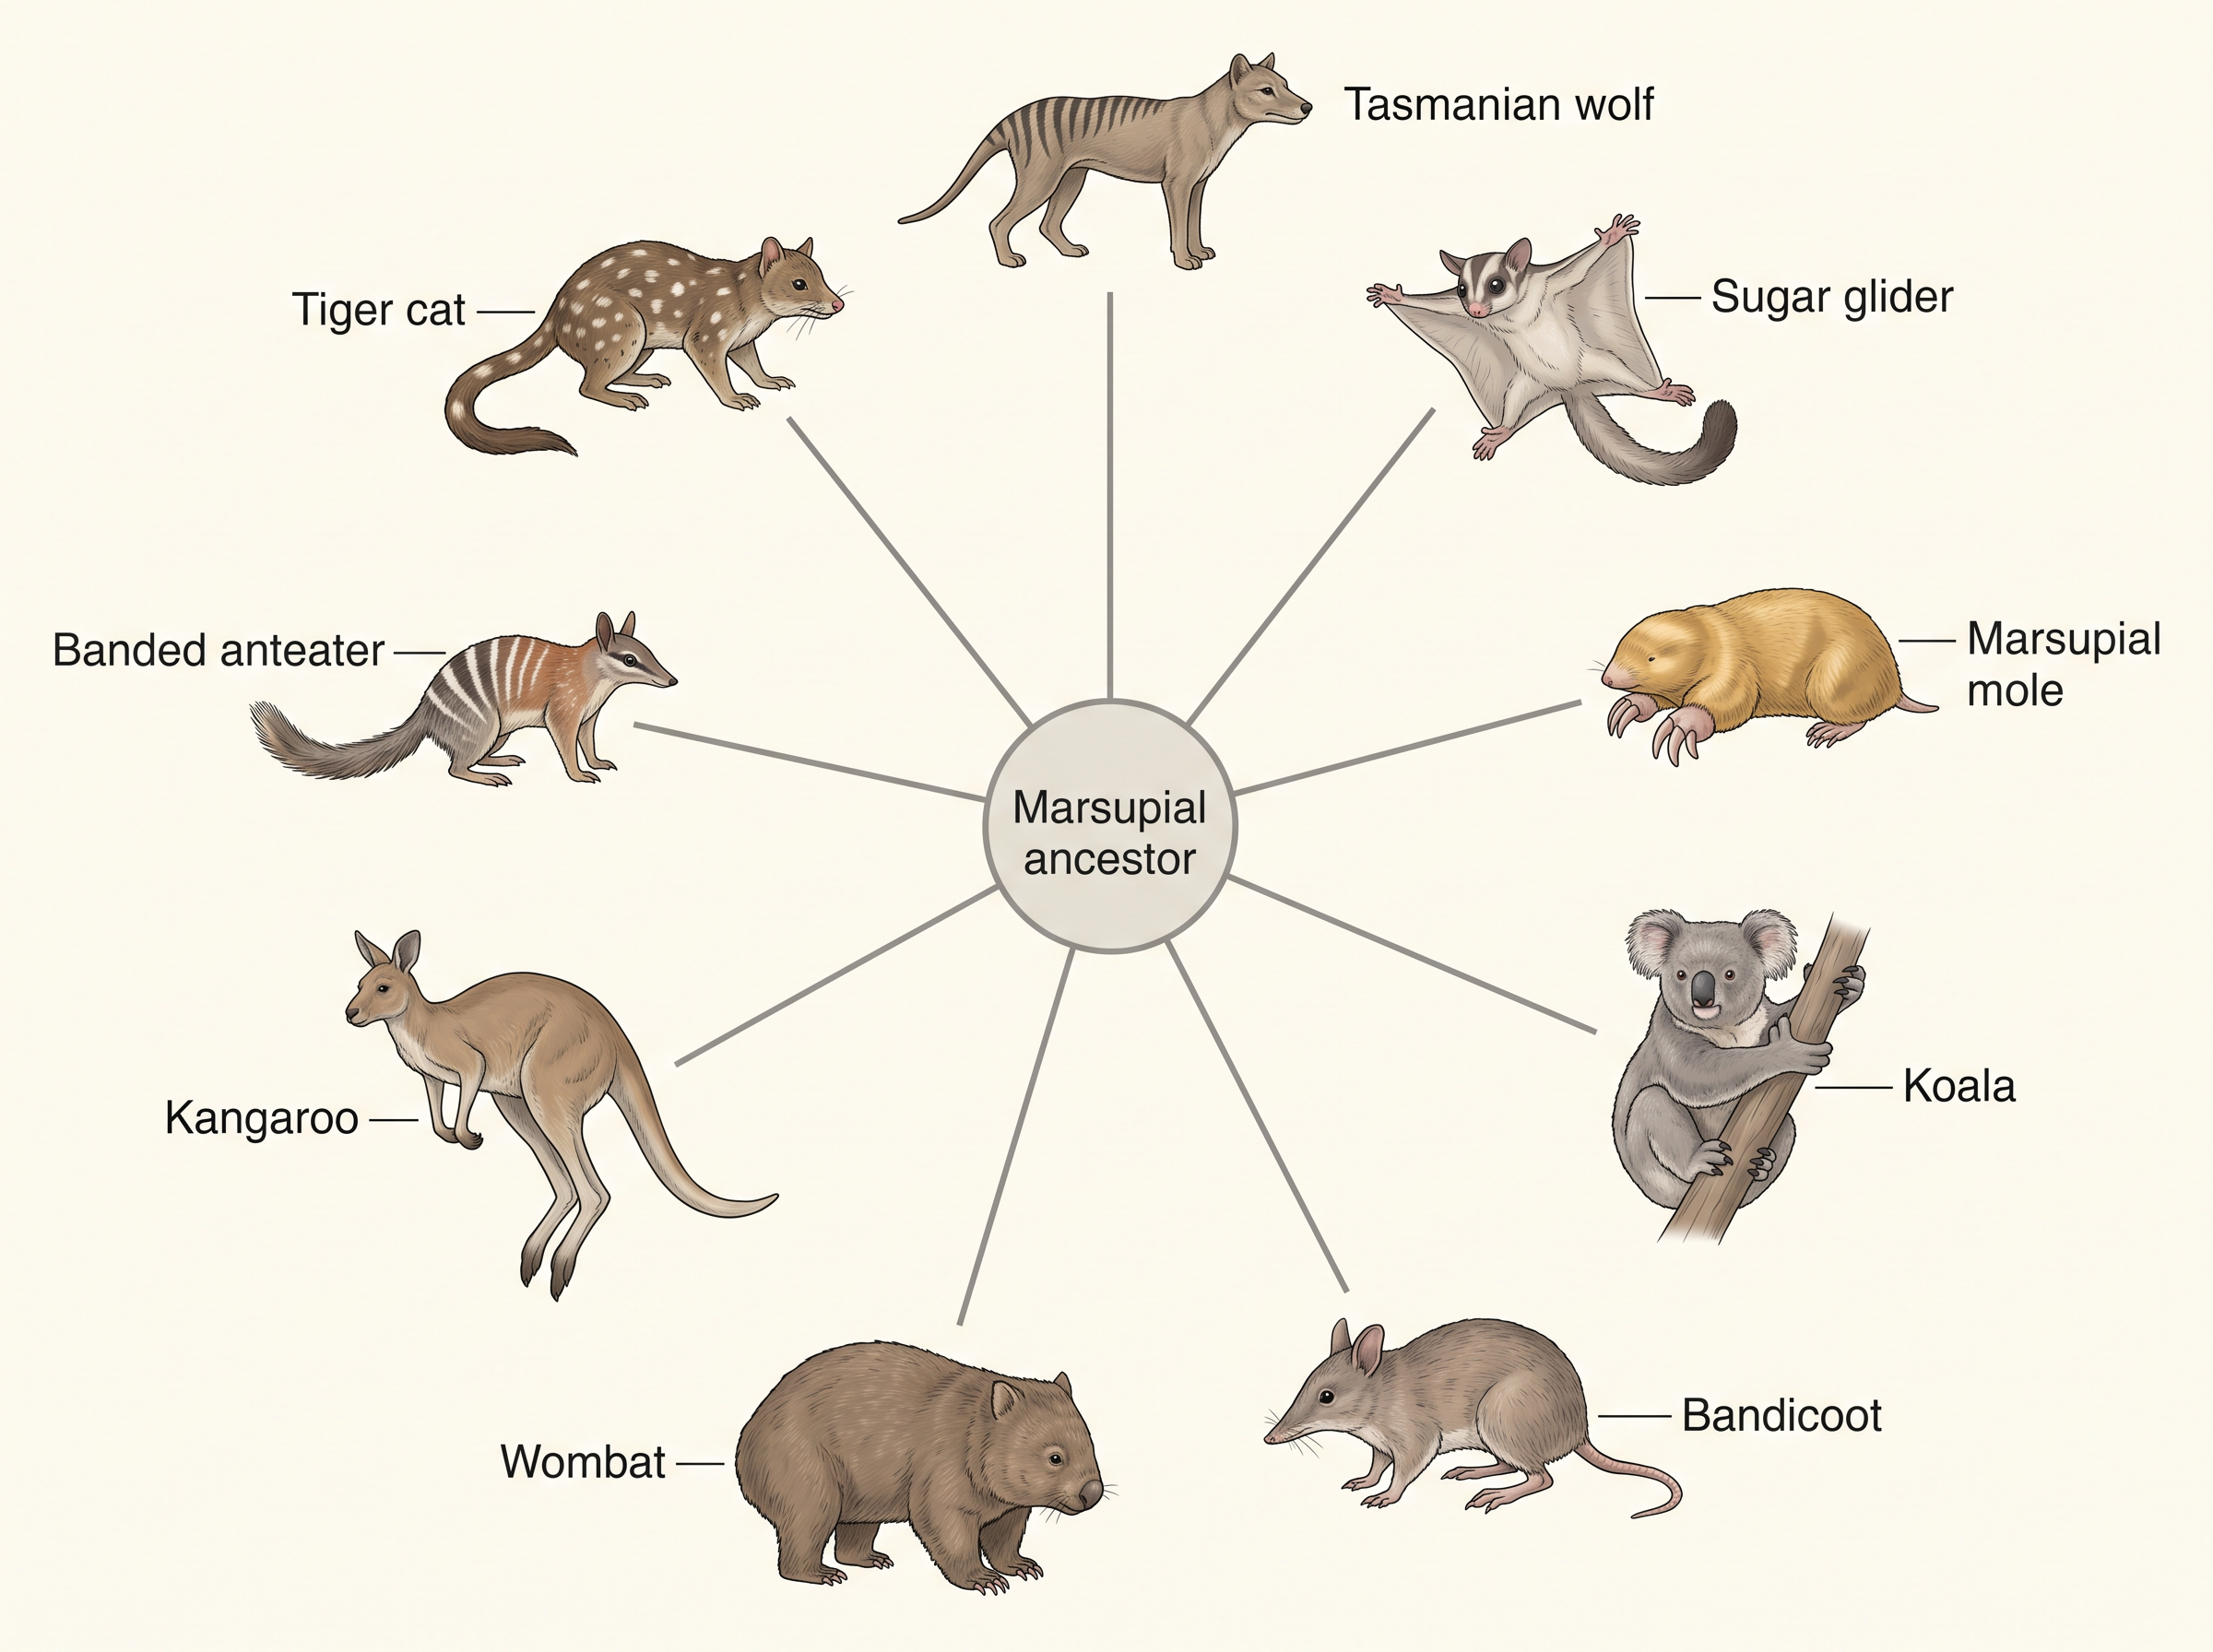
Fig. 6.8 – Adaptive radiation of Australian marsupials.
Interestingly, more than one adaptive radiation can occur in the same isolated area. Placental mammals elsewhere in the world also underwent adaptive radiation, evolving into varieties in which each form comes to resemble a corresponding Australian marsupial — for example, the placental wolf and the Tasmanian wolf (a marsupial), as shown in Fig. 6.9. When two separate radiations produce such look-alike forms, this resemblance is an example of convergent evolution, the same idea we met in Section 6.3 (analogous structures evolving toward the same function).
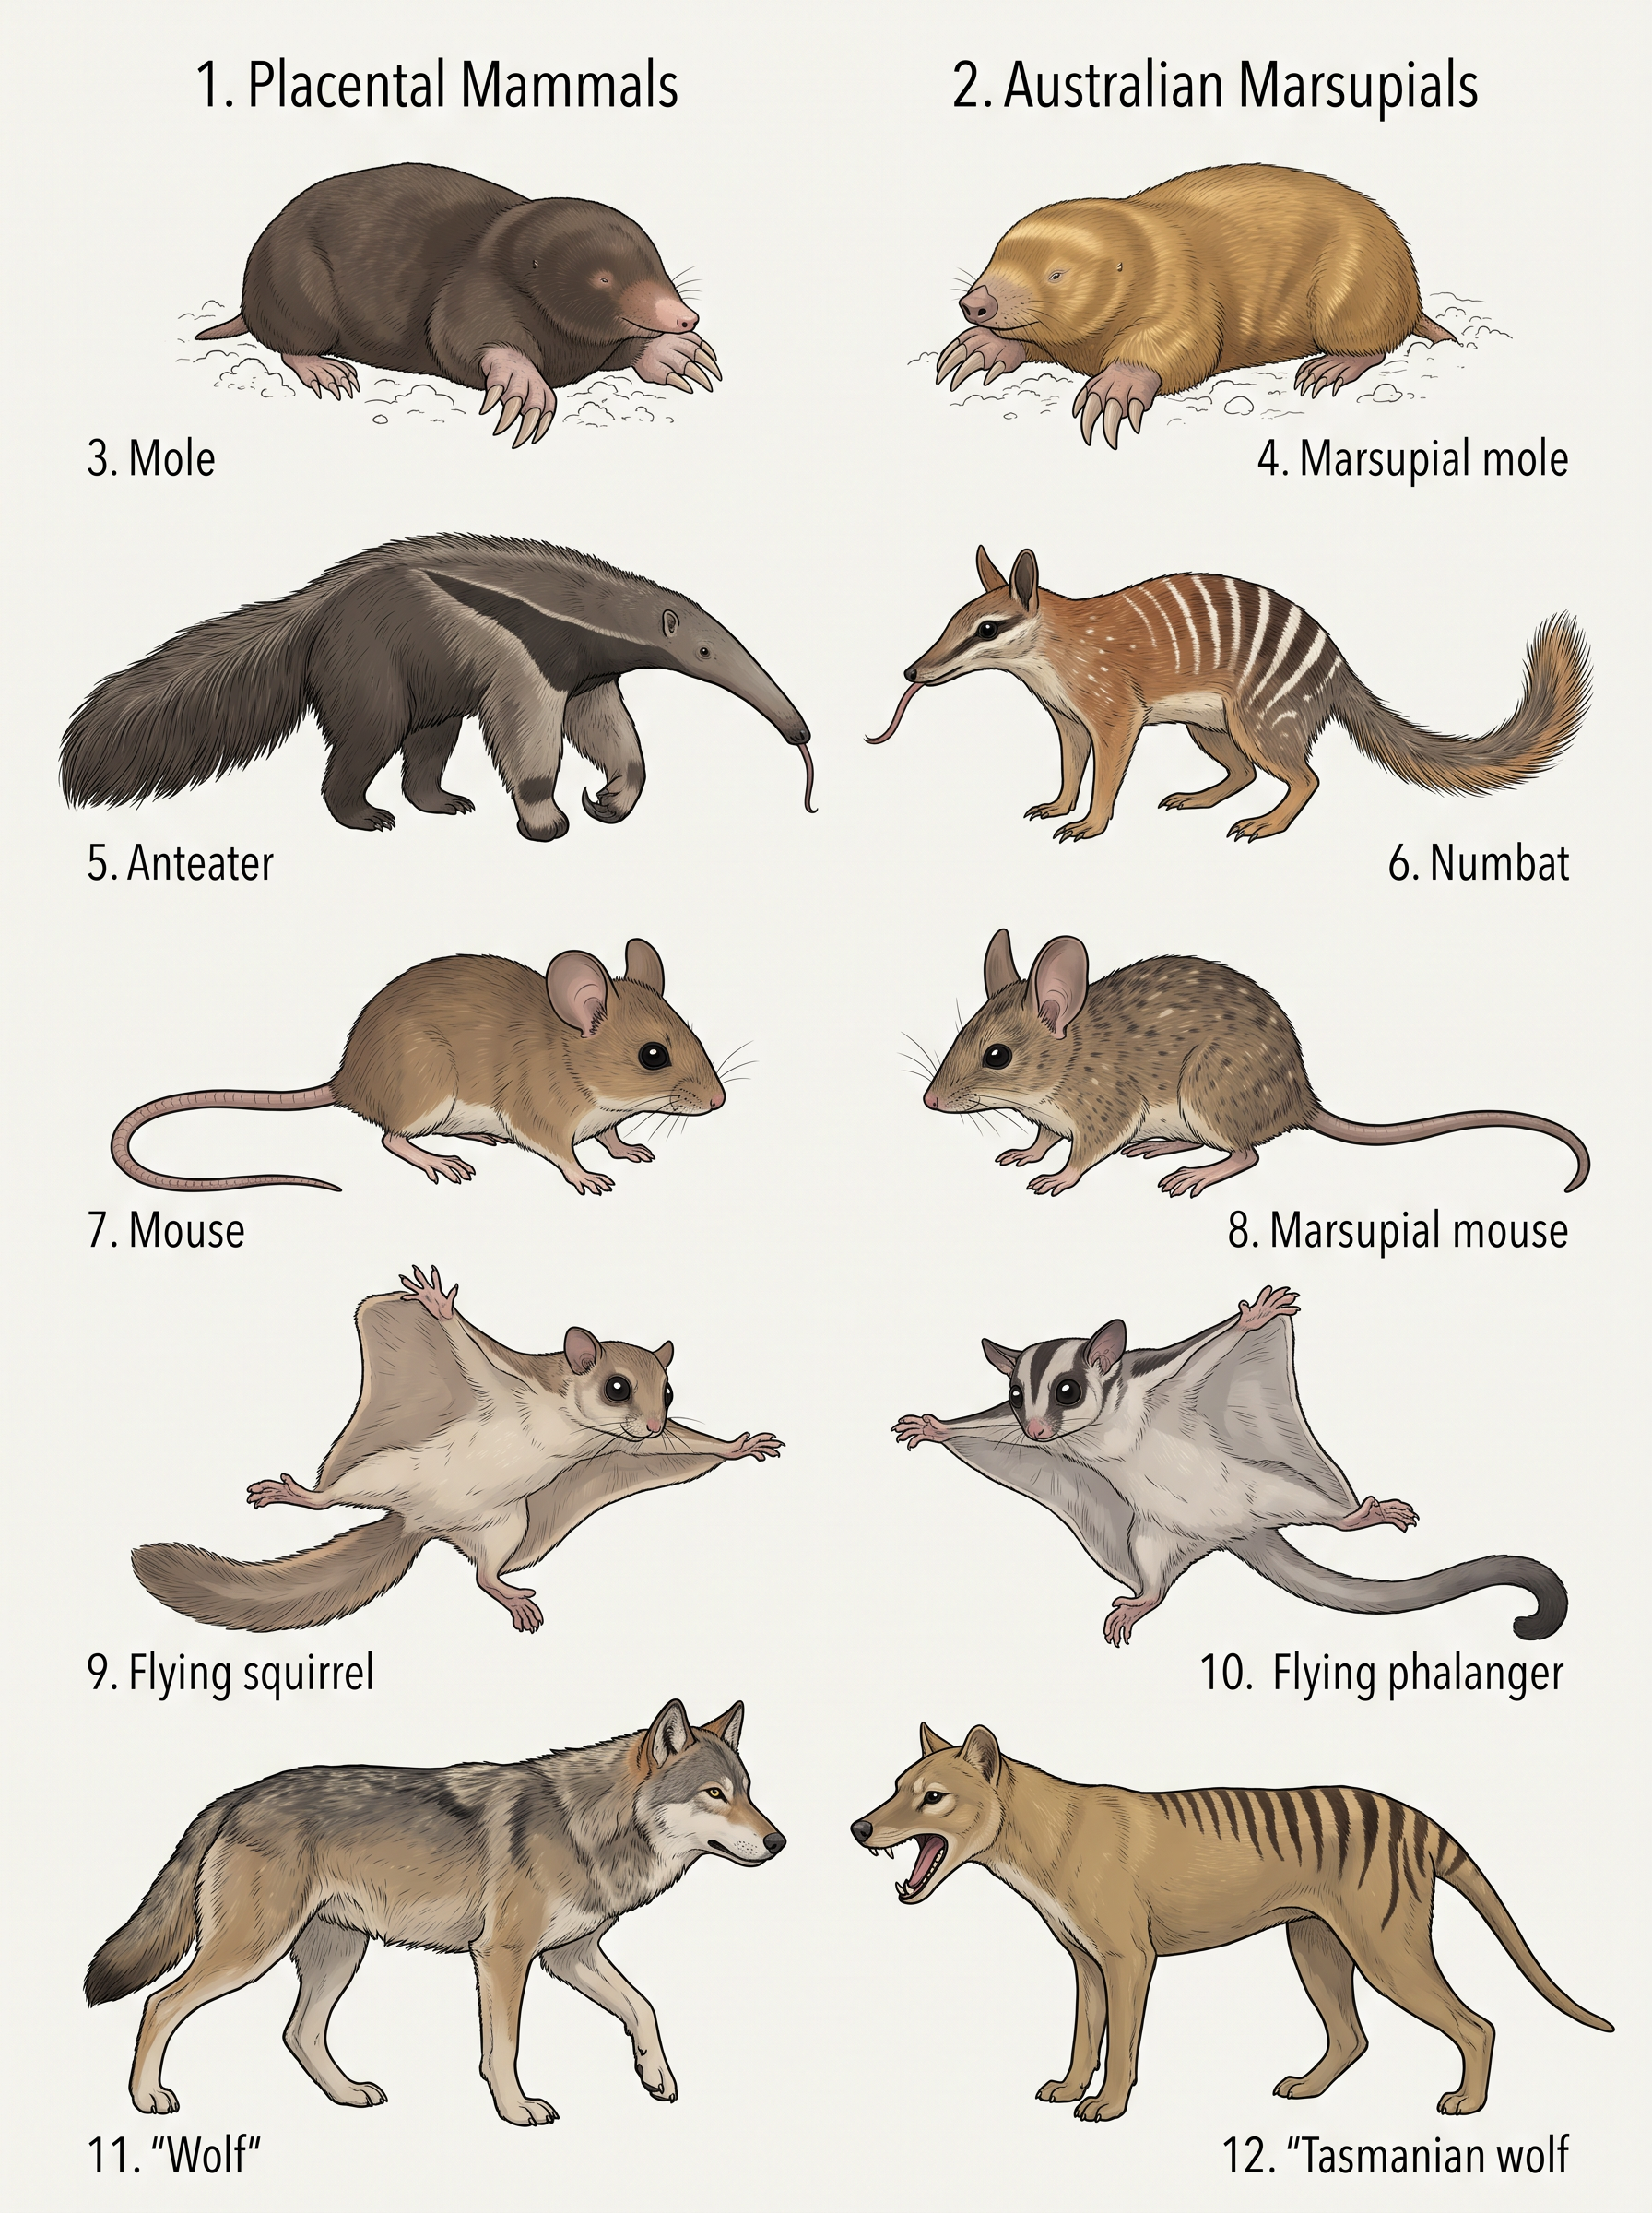
Fig. 6.9 – Convergent evolution in placental and marsupial mammals.
6.5 Biological Evolution
In a true sense, evolution by natural selection would have begun only when cellular forms of life, differing in their metabolic capabilities, first appeared on Earth. Once there were cells that were not all identical, nature had something to “choose” between. The very essence of Darwinian theory is this idea of natural selection, which we first met in Section 6.2.
Why Fast-breeding Organisms Evolve Faster
The rate at which new forms appear is closely linked to an organism’s life cycle and life span. Microbes that divide rapidly can multiply into millions of individuals within hours, so evolution in them can be very fast.
Consider a colony of bacteria — call it population A — growing on a given medium. This colony already has built-in variation: individuals differ in their ability to use a particular feed component. Now suppose the composition of the medium is changed. Only that part of the population — call it B — which can survive under the new conditions will grow.
In due course, this variant population B outgrows the others and appears as a new species. Remarkably, this can happen within days. For the same change to occur in a fish or a fowl would take millions of years, because the life spans of these animals are measured in years, not hours.
Here we say that under the new conditions, the fitness of B is better than that of A. Nature selects for fitness. But it is vital to remember that this fitness is based on characteristics that are inherited. There must therefore be a genetic basis for an organism to be selected and to evolve.
Put another way, some organisms are simply better adapted to survive in an otherwise hostile environment. This adaptive ability is inherited — it has a genetic basis. Fitness, then, is the end result of an organism’s inherited ability to adapt and be selected by nature.
The Two Pillars: Branching Descent and Natural Selection
Two key concepts hold up the Darwinian Theory of Evolution: branching descent and natural selection. Branching descent means that new species branch off from common ancestral stocks — like limbs branching from a tree trunk — which is why related organisms share similarities. This branching pattern is what we saw earlier in the marsupial and placental radiations of Fig. 6.9, while the different ways natural selection can act on a population are shown later in Fig. 6.10.
Lamarck’s Idea of Use and Disuse
Even before Darwin, a French naturalist named Lamarck proposed that evolution had occurred, but he explained it differently — through the use and disuse of organs. According to Lamarck, an organ that is used more develops further, while one that is not used shrinks, and these changes acquired during life are then passed on to the offspring.
His famous example was the giraffe. Lamarck suggested that giraffes, straining to reach leaves on tall trees, stretched and elongated their necks, and that this acquired long neck was passed on to succeeding generations, so that over the years giraffes came to have long necks. This particular conjecture — the inheritance of acquired characters — is no longer believed by anyone today.
Is Evolution a Process or a Result?
There is an interesting question to pause on: is evolution a process, or the result of a process? The world we see around us — living and non-living — is really only the collection of evolution’s success stories. When we describe this world, we treat evolution as a process. But when we describe the story of life on Earth, we treat evolution as the consequence of a process called natural selection. Even now, biologists are not entirely settled on whether to regard evolution and natural selection as processes in themselves or as the end results of deeper, unknown processes.
Darwin, Malthus and the Struggle for Existence
It is likely that the work of Thomas Malthus on human populations influenced Darwin’s thinking. Natural selection rests on a set of factual observations. First, natural resources are limited. Second, populations tend to remain stable in size, apart from seasonal fluctuations. Third, the members of a population vary in their characteristics — in fact, no two individuals are exactly alike, even if they look superficially similar. Fourth, most of these variations are inherited.
From these facts follows a powerful argument. In theory, a population would grow exponentially if every individual reproduced to the maximum — something clearly seen in a rapidly growing bacterial population. Yet in reality, population sizes stay limited. This gap means there must be competition for resources: only some individuals survive and flourish, while others do not.
Darwin’s brilliant and original insight was this: variations that are heritable, and that help a few individuals use resources better (that is, adapt better to their habitat), will allow only those individuals to reproduce and leave more progeny. This chain of reasoning is summarised in FC 6.4.
Flowchart
FC 6.4 – Darwin’s reasoning (influenced by Malthus): organisms can reproduce exponentially → but resources are limited and populations stay stable → so there is competition (struggle for existence) → individuals vary, and most variation is heritable → those with favourable heritable variations survive and reproduce more → their traits become common over many generations → population characteristics change → new forms appear to arise
So, over a period of time and across many generations, the survivors leave more progeny, the characteristics of the population shift, and new forms appear to arise. This gradual change in populations, driven by natural selection acting on inherited variation, is the heart of biological evolution.
6.6 Mechanism of Evolution
Natural selection acts on variation — but where does this variation come from in the first place, and how exactly do new species form (a process called speciation)? Interestingly, Gregor Mendel had already spoken of inheritable “factors” (what we now call genes) that influence an organism’s phenotype — its observable characteristics. Yet Darwin either ignored these observations or stayed silent about them, so the source of variation remained an open question in his theory.
deVries and the Idea of Mutation
An answer came in the first decade of the twentieth century. Working on the evening primrose (Oenothera), Hugo deVries put forward the idea of mutations — large differences that arise suddenly in a population, rather than building up slowly.
deVries believed that it was mutation, and not the minor heritable variations that Darwin had emphasised, which actually caused evolution. He pointed out a key difference: mutations are random and directionless, whereas the variations Darwin described are small and directional.
There was also a difference in pace. For Darwin, evolution was gradual, occurring through the slow accumulation of small variations. For deVries, mutation could cause speciation in a single large step, which he called saltation. Later studies in population genetics helped bring some clarity by combining both ideas — showing how mutation supplies new variation while natural selection then acts upon it.
6.7 Hardy–Weinberg Principle
So far we have talked about evolution in words. But can we actually measure whether a population is evolving? The Hardy–Weinberg principle lets us do exactly that, using simple algebra.
In any given population, we can work out the frequency (proportion) of each allele of a gene, at a particular locus (position on a chromosome). The Hardy–Weinberg principle states that, under certain conditions, this frequency stays fixed and remains the same through the generations — and it captures this idea in the form of algebraic equations.
Allele Frequencies and Genetic Equilibrium
The principle says that allele frequencies in a population are stable and constant from generation to generation. The gene pool — the total of all genes and their alleles in a population — remains constant. This unchanging state is called genetic equilibrium. The sum total of all the allele frequencies is 1.
Individual allele frequencies are given letters such as \(p\) and \(q\). In a diploid organism (one with two sets of chromosomes), let \(p\) be the frequency of allele \(A\) and \(q\) the frequency of allele \(a\). Since these are the only two alleles, \(p + q = 1\).
Now think about how these alleles combine in individuals. The frequency of \(AA\) individuals in the population is simply \(p^2\). Why? Because the probability that an allele \(A\), with frequency \(p\), appears on both chromosomes of a diploid individual is the product of the two probabilities, that is \(p \times p = p^2\). In the same way, the frequency of \(aa\) individuals is \(q^2\), and the frequency of heterozygous \(Aa\) individuals is \(2pq\) (the factor of 2 appears because \(Aa\) can form in two ways — \(A\) from one parent and \(a\) from the other, or the reverse).
Adding up all the genotype frequencies gives:
\[p^2 + 2pq + q^2 = 1\]
This is simply the binomial expansion of \((p+q)^2\). Here \(p\) is the frequency of the dominant allele, \(q\) the frequency of the recessive allele; \(p^2\), \(2pq\) and \(q^2\) are the expected frequencies of the \(AA\), \(Aa\) and \(aa\) genotypes respectively (all are proportions, so they have no units).
The real power of this principle lies in what happens when it fails. When the frequencies actually measured in a population differ from the values expected from the equation, that difference — and its direction — reveals the extent of evolutionary change. In other words, any disturbance of the genetic (Hardy–Weinberg) equilibrium, meaning a change in allele frequencies in a population, is interpreted as evolution taking place.
Five Factors that Disturb the Equilibrium
Five factors are known to disturb Hardy–Weinberg equilibrium: gene migration (gene flow), genetic drift, mutation, genetic recombination, and natural selection.
When a section of a population migrates to another place and joins a different population, gene frequencies change both in the original population and in the new one. New genes or alleles are added to the new population and are lost from the old one. If this movement of genes (gene migration) happens repeatedly, we call it gene flow.
If a similar change in allele frequency happens purely by chance, rather than through migration, it is called genetic drift. Sometimes the change in allele frequency in a small new sample of a population is so different that these individuals become a different species altogether. When such a drifted group starts a new population, the individuals become the “founders,” and this outcome is called the founder effect.
How Selection Reshapes a Population
Microbial experiments show that when pre-existing advantageous mutations are selected, new phenotypes appear; over a few generations, this can lead to speciation. Natural selection, as we have seen, is a process in which heritable variations that enable better survival allow those individuals to reproduce and leave a greater number of progeny.
A careful analysis leads us to a clear picture. Variation arising from mutation, from recombination during gametogenesis (the formation of gametes), or from gene flow and genetic drift, all change the frequency of genes and alleles in future generations. When this changed variation is coupled with enhanced reproductive success through natural selection, the population ends up looking like a different one.
Natural selection can act on a trait in three different ways, shown in Fig. 6.10. It can lead to stabilisation, in which more individuals come to have the mean (average) character value; to directional change, in which more individuals acquire a value away from the mean; or to disruption, in which more individuals acquire the extreme values at both ends of the distribution curve.
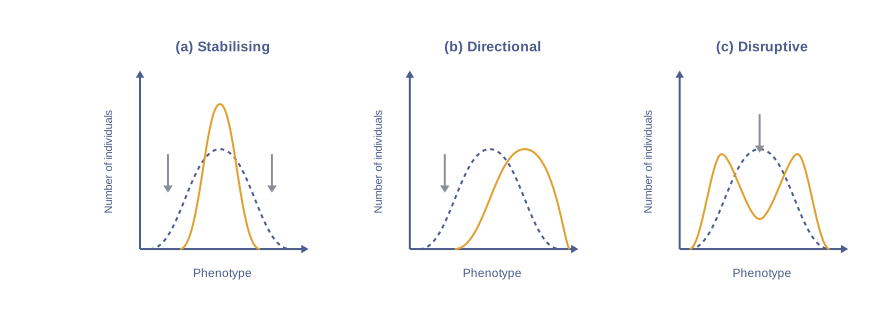
Fig. 6.10 – Three modes of natural selection.
6.8 A Brief Account of Evolution
Having seen how evolution works, let us now take a quick walk through the actual history of life on Earth — a story that unfolds over billions of years and is sketched on a geological scale in Fig. 6.11 (for plants) and Fig. 6.12 (for vertebrates).
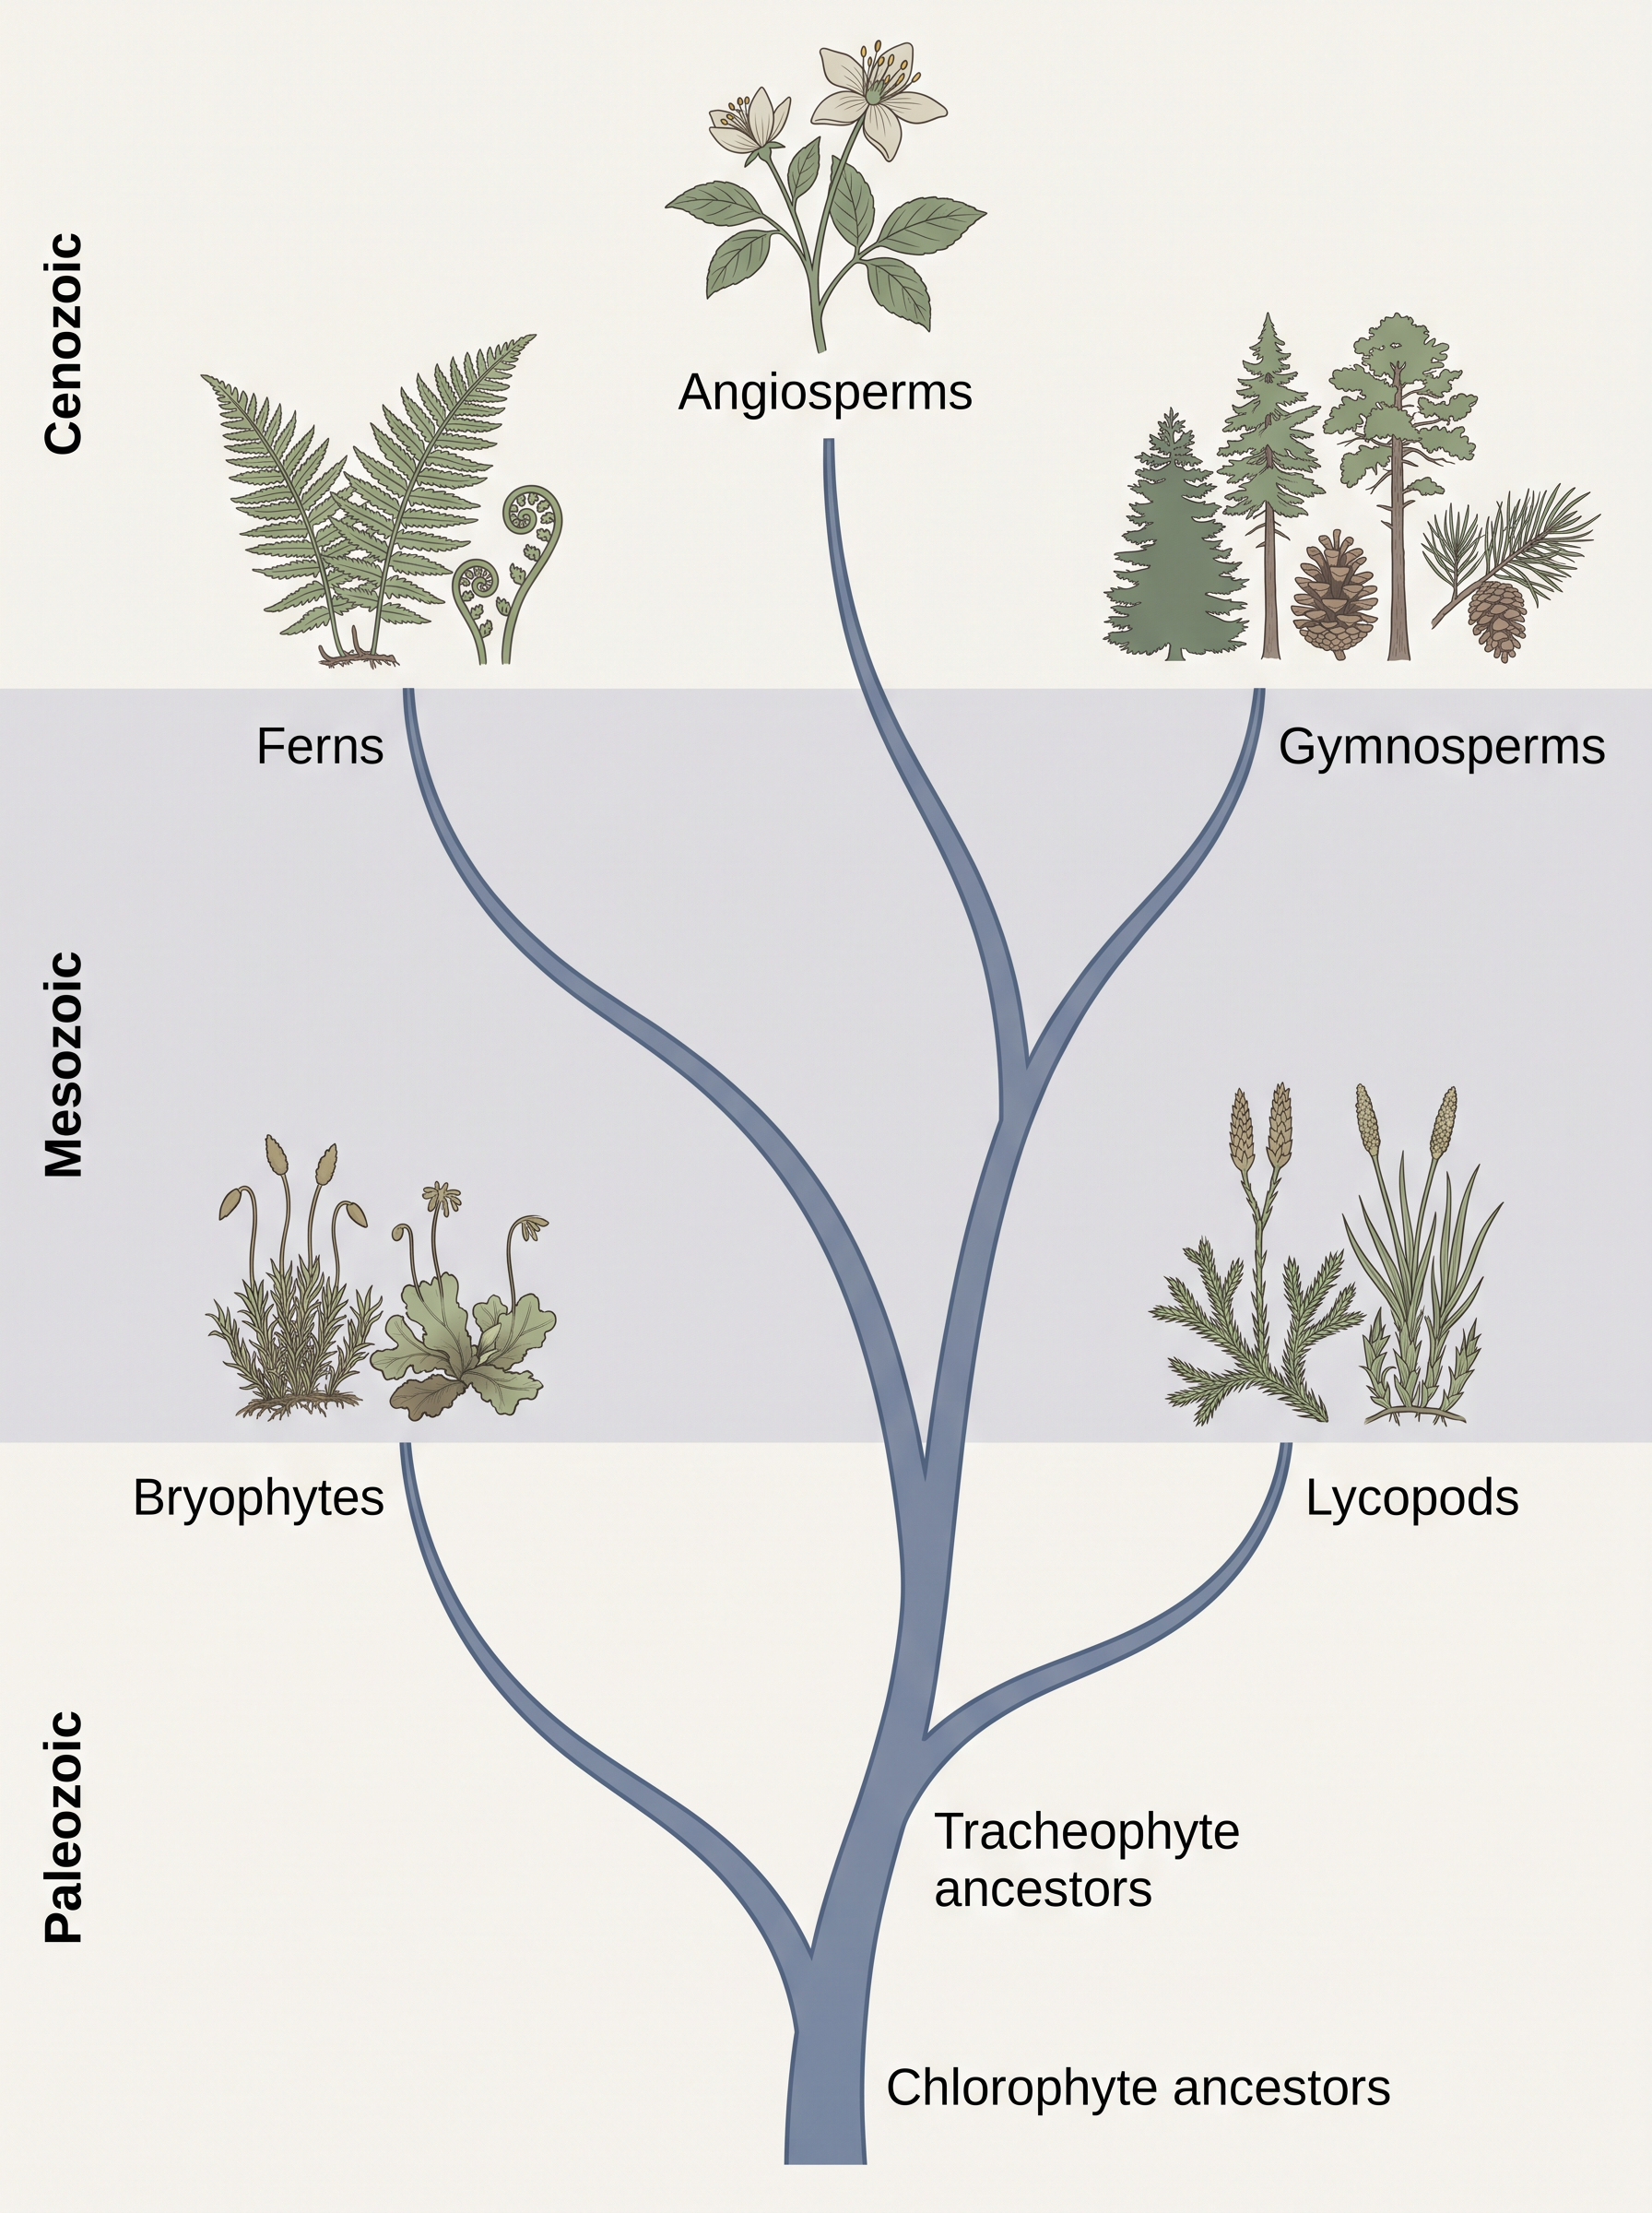
Fig. 6.11 – Evolutionary history of plants.
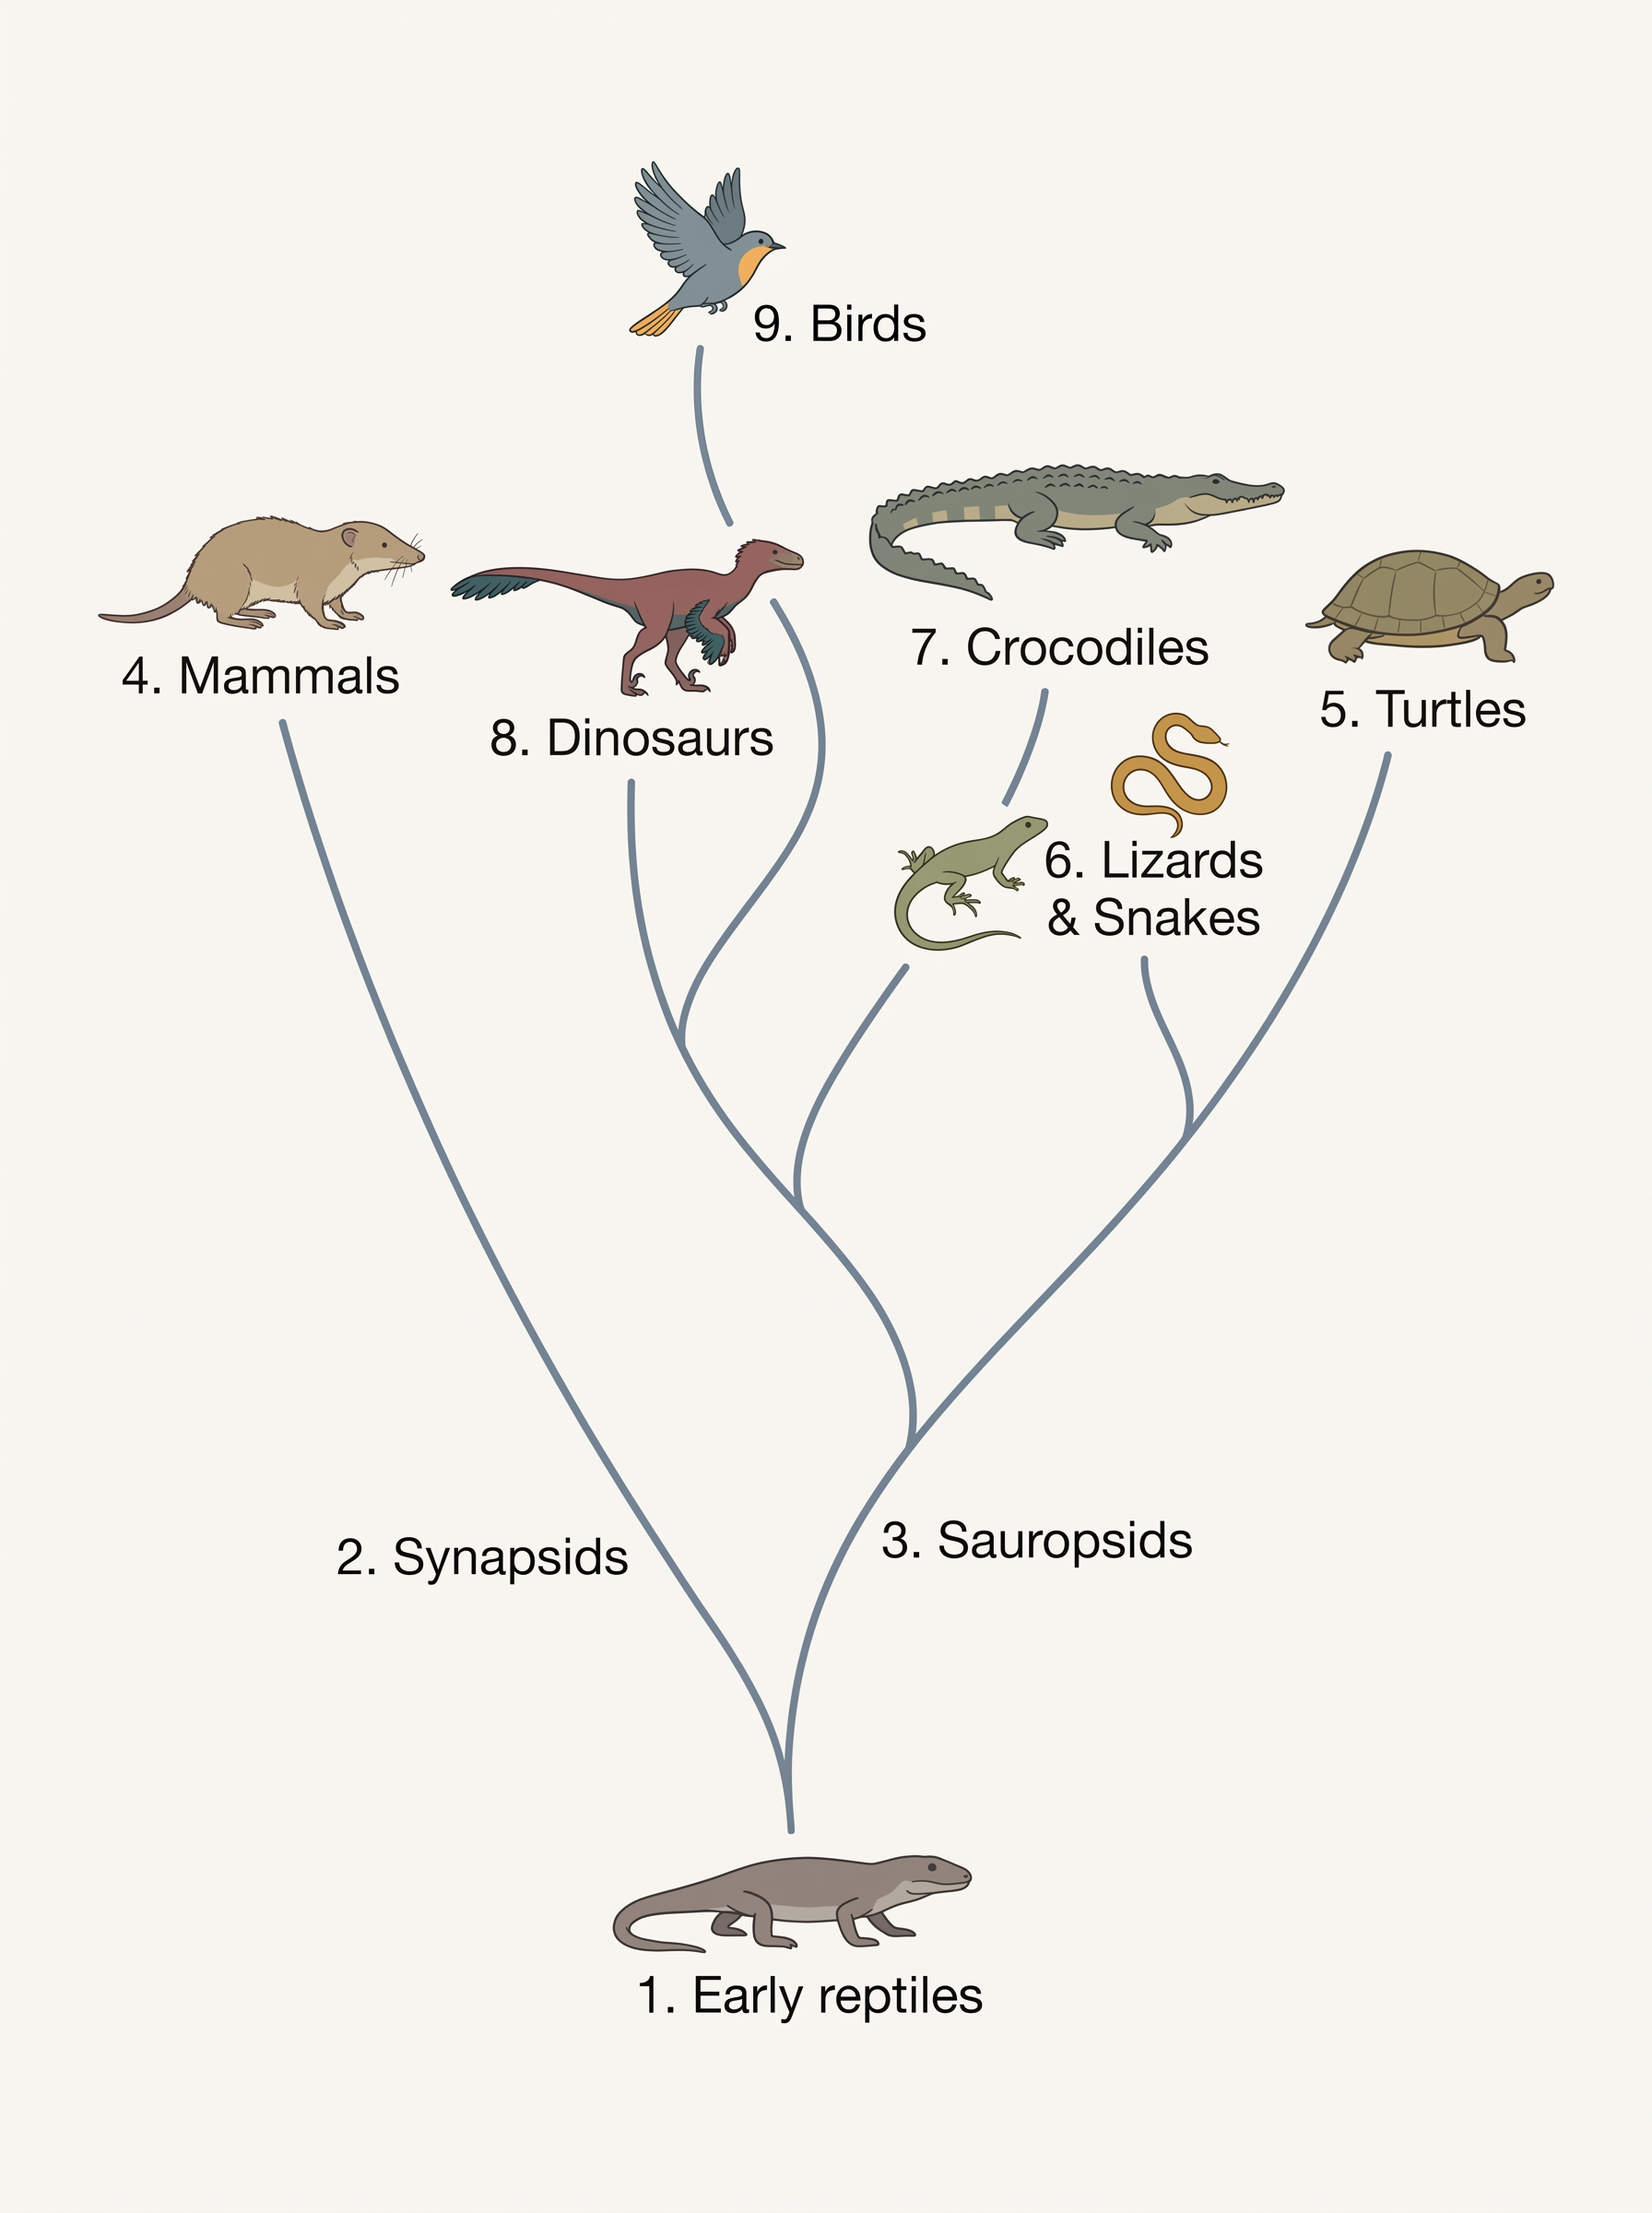
Fig. 6.12 – Evolutionary tree of vertebrates.
From First Cells to Multicellular Life
About 2000 million years ago (mya), the first cellular forms of life appeared on Earth. Exactly how non-cellular aggregates of giant macromolecules evolved into cells with a membranous envelope is still not known.
Some of these early cells had the ability to release oxygen (\(O_2\)). The reaction responsible could have been similar to the light reaction of photosynthesis, in which water is split using solar energy that is captured and channelled by suitable light-harvesting pigments. Slowly, single-celled organisms gave rise to multicellular life forms.
Life Invades the Land
By about 500 mya, invertebrates (animals without a backbone) had formed and become active. Jawless fish probably evolved around 350 mya. Seaweeds and a few plants existed probably around 320 mya.
We are told that the first organisms to invade the land were plants. They had already spread widely across the land by the time animals moved onto it. Meanwhile, fish with stout, strong fins could move onto land and return to water; this was about 350 mya.
As we saw in the chapter opener, in 1938 a coelacanth — a fish thought to have been extinct for millions of years — was caught alive off South Africa. Such fish, called lobefins, evolved into the first amphibians, animals able to live both on land and in water. No specimens of these earliest amphibians survive, but they were the ancestors of modern-day frogs and salamanders.
The Age of Reptiles
The amphibians, in turn, evolved into reptiles. A crucial advance was the reptilian egg: reptiles lay thick-shelled eggs that do not dry up in the sun, unlike the eggs of amphibians. Today we see only their modern descendants — the turtles, tortoises and crocodiles.
Over the next 200 million years or so, reptiles of many different shapes and sizes dominated the Earth. Giant ferns (pteridophytes — the non-flowering plants with true roots, stems and leaves) grew abundantly, but over time they fell and slowly formed today’s coal deposits.
Some of these land reptiles returned to the water and evolved into fish-like reptiles, probably around 200 mya — for example, the Ichthyosaurs. The land reptiles were, of course, the dinosaurs. The biggest of them, Tyrannosaurus rex, stood about 20 feet in height and had huge, fearsome, dagger-like teeth.
Then, about 65 mya, the dinosaurs suddenly disappeared from the Earth. The true reason is not known. Some suggest climatic changes killed them; others believe most of them evolved into birds. The truth may lie somewhere in between. Small-sized reptiles of that era still exist today.
The Rise of Mammals
The first mammals were shrew-like, and their fossils are small-sized. Mammals were viviparous — they gave birth to live young and protected their unborn offspring inside the mother’s body. They were also, at the very least, more intelligent at sensing and avoiding danger. So when the reptiles declined, mammals took over the Earth.
The movements of continents played a part in this story too. Continental drift is the very slow shifting of the Earth’s continents over geological time. In South America there were mammals resembling the horse, hippopotamus, bear and rabbit. Due to continental drift, when South America joined North America, these animals were overridden by the North American fauna. The same continental drift, however, allowed the pouched mammals (marsupials) of Australia to survive, because they faced no competition from other mammals there.
We should not forget that some mammals returned to live wholly in water — whales, dolphins, seals and sea cows are examples. The evolution of the horse, elephant and dog are each special stories that you will study in higher classes. But the most remarkable story of all is the evolution of human beings, with their language skills and self-consciousness.
The whole sweep of this history, from the first cell to modern mammals, is summarised in FC 6.5.
Flowchart
FC 6.5 – Timeline of life: first cellular life (~2000 mya) → single cells become multicellular → invertebrates (~500 mya) → jawless fish (~350 mya) → seaweeds and early plants (~320 mya) → plants invade land, then animals → lobefins move onto land (~350 mya) → first amphibians (frogs, salamanders) → reptiles (thick-shelled eggs) → dinosaurs dominate; some return to water as Ichthyosaurs (~200 mya) → dinosaurs disappear (~65 mya) → mammals take over → evolution of humans
6.9 Origin and Evolution of Man
Of all the stories of evolution, the one that fascinates us most is our own — the origin and evolution of human beings, with our language and self-consciousness. Piecing it together from fossils, we can trace a path from ape-like ancestors to modern humans.
Early Ape-like Ancestors
About 15 mya, primates called Dryopithecus and Ramapithecus were living on Earth. They were hairy and walked much like today’s gorillas and chimpanzees. Of the two, Ramapithecus was more man-like, while Dryopithecus was more ape-like.
Walking Upright in Africa
A few fossils of man-like bones have been discovered in Ethiopia and Tanzania. Studying features such as these (compare the skulls in Fig. 6.13), scientists came to believe that about 3–4 mya, man-like primates walked in eastern Africa. They were probably not taller than 4 feet, but importantly, they walked upright.
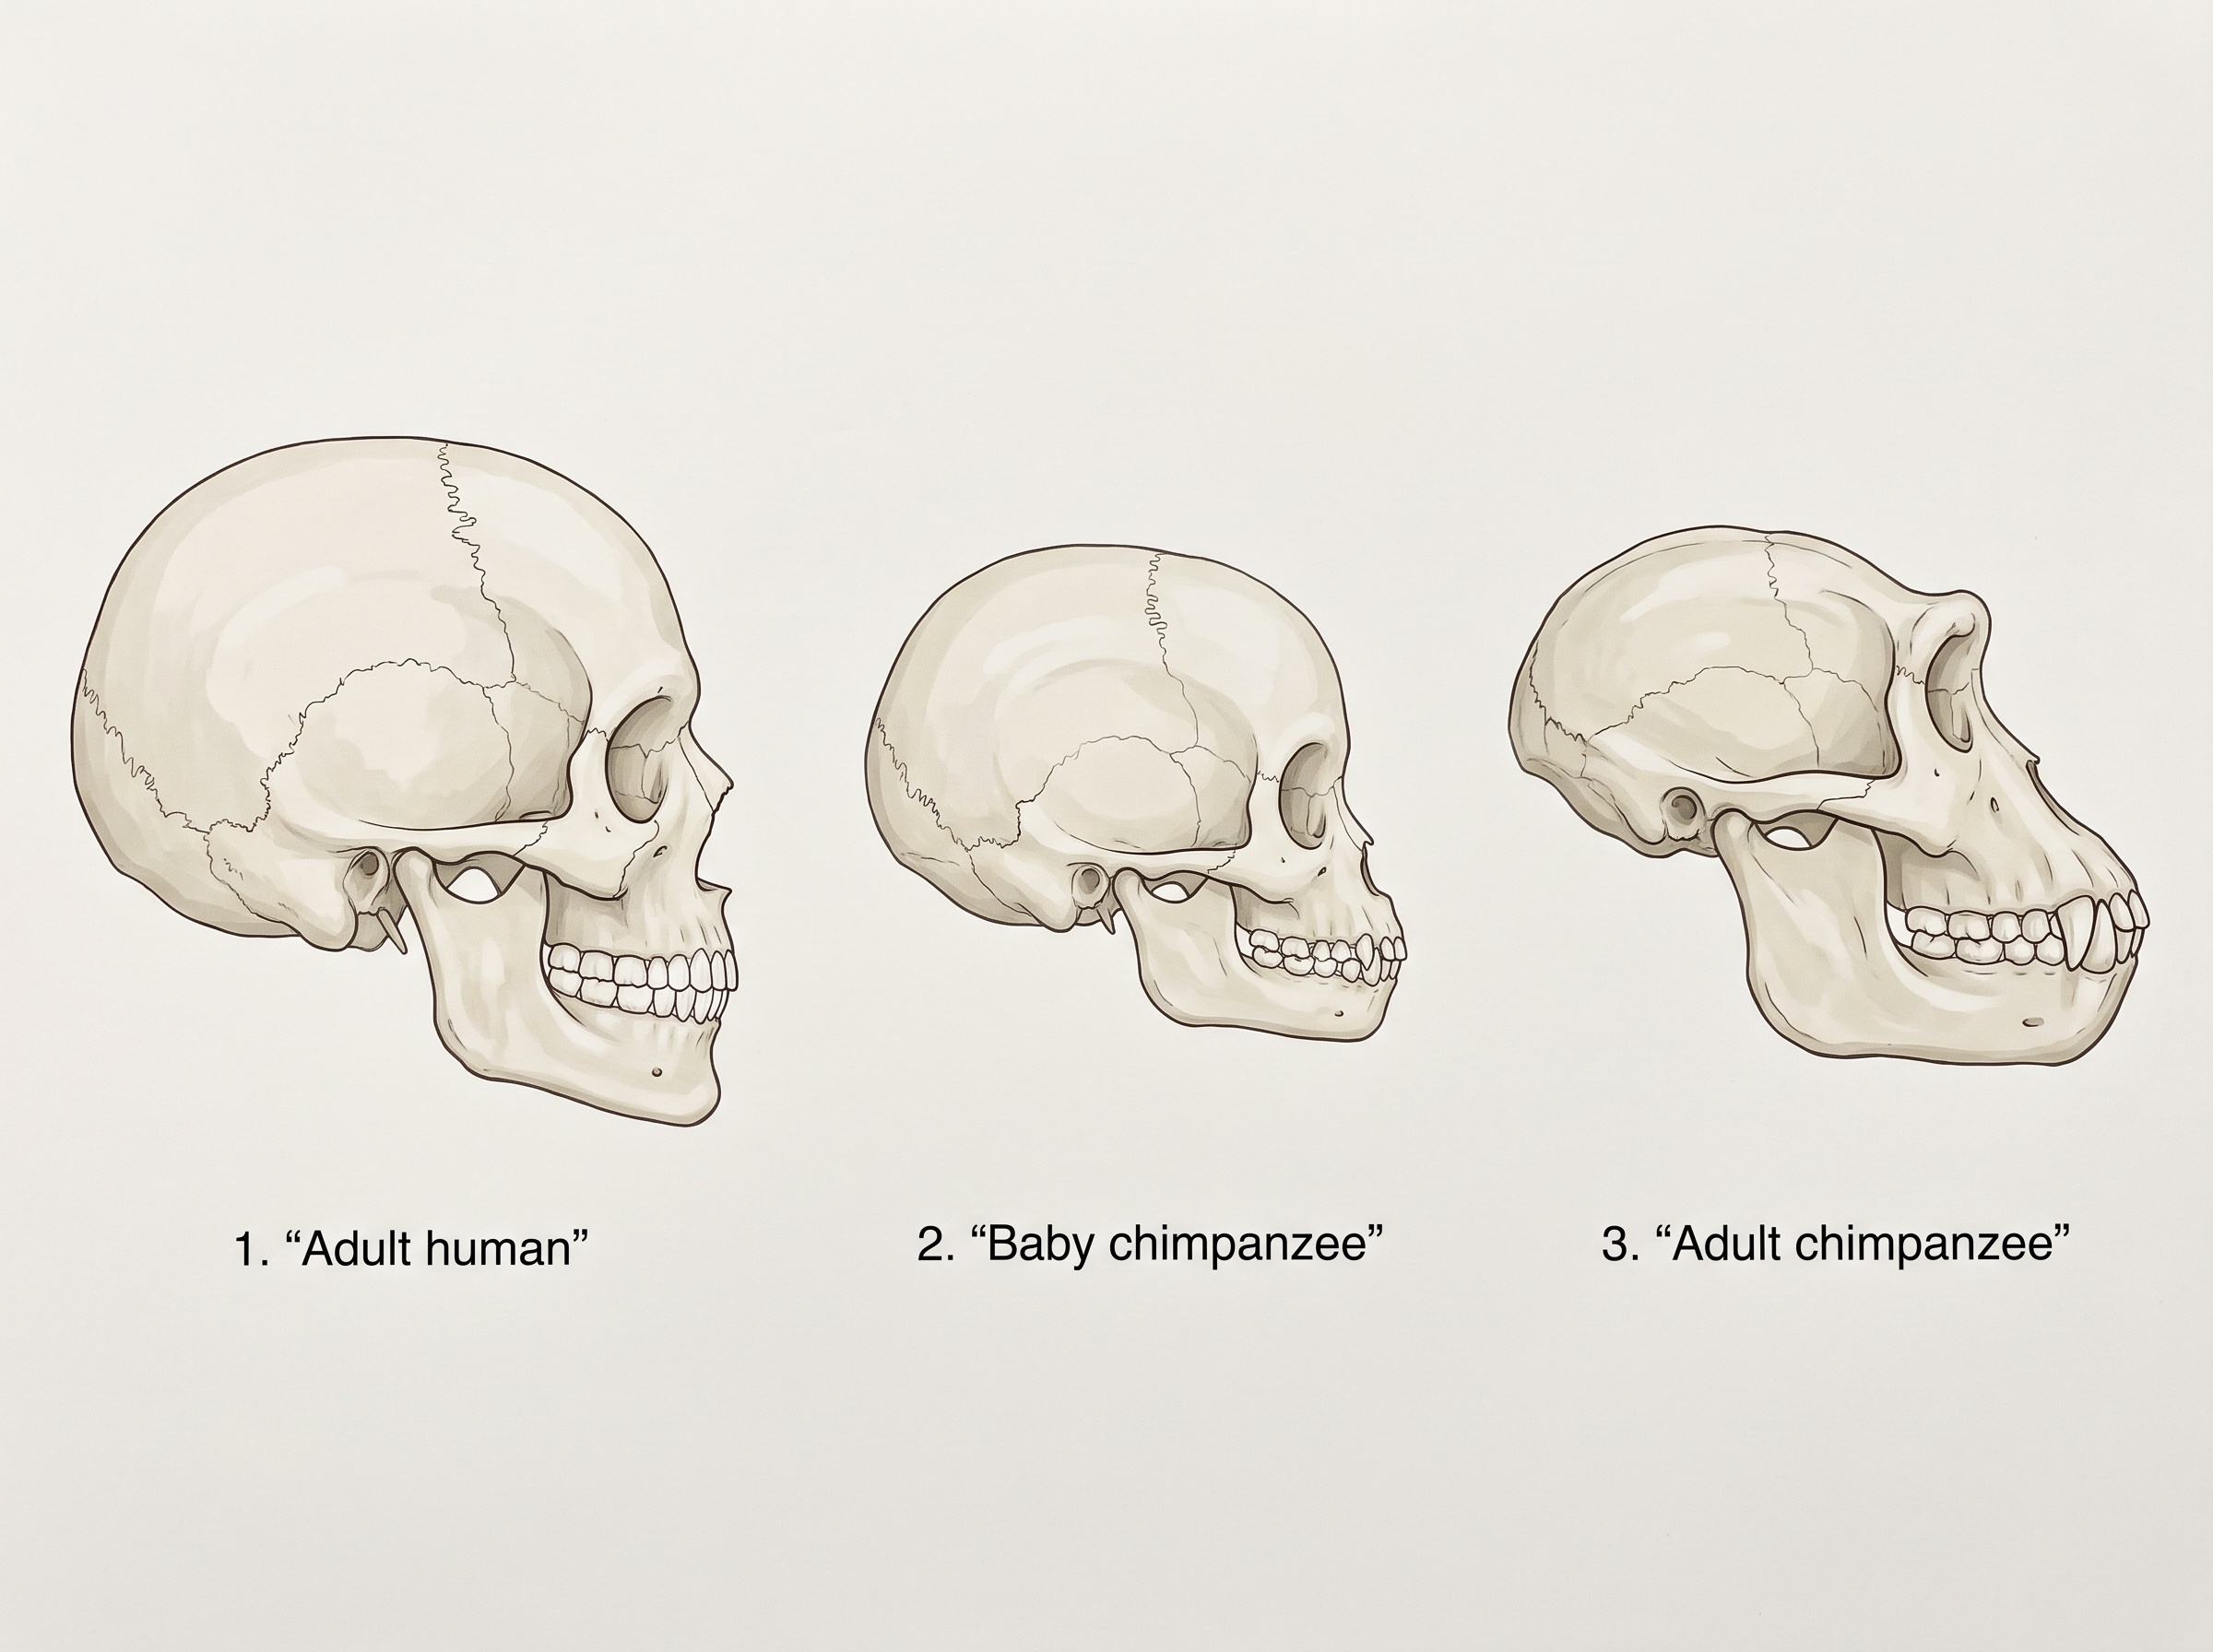
Fig. 6.13 – Comparison of human and chimpanzee skulls.
Around 2 mya, the Australopithecines probably lived in the East African grasslands. Evidence suggests they hunted with stone weapons, but essentially ate fruit.
The Genus Homo
Among the fossils discovered, some bones were clearly different. This creature was regarded as the first human-like being — the hominid — and was named Homo habilis. Its brain capacity was between 650 and 800 cc, and it probably did not eat meat.
The next stage was revealed by fossils discovered in Java in 1891: Homo erectus, living about 1.5 mya. Homo erectus had a larger brain, around 900 cc, and probably did eat meat.
Later came the Neanderthal man, with a brain size of about 1400 cc, who lived in the near east and central Asia between 1,00,000 and 40,000 years ago. Neanderthals used animal hides to protect their bodies and buried their dead — a sign of complex behaviour.
Finally, Homo sapiens — our own species — arose in Africa, moved across the continents, and developed into distinct races. During the ice age, between 75,000 and 10,000 years ago, modern Homo sapiens arose.
From Cave Art to Civilisation
Pre-historic cave art developed about 18,000 years ago. One such set of cave paintings, made by pre-historic humans, can be seen at the Bhimbetka rock shelters in the Raisen district of Madhya Pradesh.
Agriculture came around 10,000 years ago, and with it human settlements began. The rest of what followed is part of the human history of the growth and decline of civilisations. The full path of our lineage is summarised in FC 6.6.
Flowchart
FC 6.6 – Human evolution: Dryopithecus & Ramapithecus (~15 mya) → man-like primates in eastern Africa (~3–4 mya, walked upright) → Australopithecus (~2 mya) → Homo habilis (650–800 cc) → Homo erectus (~1.5 mya, 900 cc) → Neanderthal man (1400 cc, 1,00,000–40,000 yrs ago) → modern Homo sapiens (75,000–10,000 yrs ago) → cave art (~18,000 yrs) → agriculture and settlements (~10,000 yrs)
6.10 Summary
The origin of life on Earth can be understood only against the background of the origin of the universe, and especially of the Earth itself.
Most scientists believe that chemical evolution — the formation of biomolecules from simpler inorganic substances — came first, before the appearance of the first cellular forms of life.
What happened next, to the first forms of life, is a conjectured (reconstructed) story built on Darwin’s ideas of organic evolution by natural selection.
The diversity of life forms on Earth has been changing continuously over millions of years, as some forms went extinct and new ones arose.
It is generally believed that the variations present within a population result in variable fitness — some individuals are better able to survive and reproduce than others.
Other phenomena, such as habitat fragmentation and genetic drift, can strengthen these variations, leading to the appearance of new species and hence to evolution.
Homology (the sharing of the same basic structure by different organisms) is explained by the idea of branching descent from common ancestors.
Evidence for evolution comes from several fields: comparative anatomy and morphology, the fossil record, and comparative biochemistry.
Among all the individual stories of evolution, the evolution of modern human beings is the most interesting, and it appears to run in parallel with the evolution of the human brain and of language.
Flowchart
FC 6.7 – Chapter overview: origin of universe and Earth → chemical evolution (biomolecules from inorganic matter) → first cellular life → variation + natural selection + branching descent → diversity of life forms → evidence from fossils, comparative anatomy and biochemistry → mechanisms (mutation, genetic drift, gene flow, selection; Hardy–Weinberg equilibrium) → history of life through geological time → evolution of modern man, brain and language
6.11 Points to Ponder
Louis Pasteur showed that life comes only from pre-existing life, and yet the very first life must have come from non-living matter. Is this really a contradiction, or do the two ideas simply apply to different conditions? What must have been true of the early Earth for non-living molecules to give rise to life?
Evolution is described as a stochastic, chance-driven process with no fixed direction. If we could rewind the history of life and let it run all over again, do you think human beings — or anything like us — would appear a second time?
For Darwin, “fitness” means reproductive success, not physical strength or intelligence. Can you imagine a situation in which the strongest or cleverest individual is actually the least fit in the Darwinian sense?
Homologous organs point to common ancestry, while analogous organs arise from similar environments acting on unrelated groups. If you discovered a completely new organism, how would you go about deciding whether one of its structures is homologous or analogous to a structure in a familiar animal?
The Hardy–Weinberg principle describes a population that is not evolving. Since no real population perfectly satisfies all of its conditions, does it follow that every real population is always evolving, even if only very slightly?
The chapter admits that the sudden disappearance of the dinosaurs is still not fully explained, and that “the truth may lie in between.” How should a scientist live with a question that has several competing answers and no firm conclusion?
The story of human evolution appears to run in parallel with the growth of the brain and of language. Does a larger brain necessarily make a species “more evolved,” or is that an idea we should treat with caution?
Lamarck’s explanation of evolution was rejected, yet the questions he was trying to answer were genuine. What was it about Darwin’s explanation that made it more convincing than Lamarck’s?
6.12 NCERT Questions
Explain antibiotic resistance in bacteria in the light of Darwin’s theory of natural selection.
Find out, from newspapers and popular science articles, any recent fossil discoveries or controversies about evolution.
Attempt to give a clear definition of the term “species”.
Try to trace the various components of human evolution (hint: brain size and function, skeletal structure, dietary preference, etc.).
Using the internet and popular science articles, find out whether animals other than humans show self-consciousness.
List 10 modern-day animals and, using internet resources, link each to a corresponding ancient fossil. Name both.
Practise drawing various animals and plants.
Describe one example of adaptive radiation.
Can we call human evolution an example of adaptive radiation?
Using resources such as your school library, the internet, and discussions with your teacher, trace the evolutionary stages of any one animal — for example, the horse.
6.13 Check Your Concepts
How did Louis Pasteur’s experiment disprove the theory of spontaneous generation? Explain what his sealed (pre-sterilised) and open flasks each showed.
Miller’s 1953 experiment is regarded as strong support for the idea of chemical evolution. Which gases did he place in his flask, and why was it important that the flask contained no free oxygen?
Assertion–Reason. Assertion (A): The wings of a butterfly and the wings of a bird are analogous organs. Reason (R): They have the same basic anatomical structure inherited from a common ancestor. State whether A and R are true, and whether R correctly explains A.
Match the pairs in Column I with the correct term in Column II.
| Column I | Column II |
|---|---|
| a. Forelimbs of whale and bat | i. Homology in plants |
| b. Wings of butterfly and bird | ii. Analogy in plants |
| c. Thorn of Bougainvillea and tendril of Cucurbita | iii. Homology in animals |
| d. Sweet potato and potato | iv. Analogy in animals |
Explain how the change in the proportion of pale and dark peppered moths in industrial England supports evolution by natural selection.
What happens to a bacterial population when an antibiotic is introduced, and why do resistant strains appear so rapidly? Relate your answer to Darwinian selection.
Distinguish between divergent and convergent evolution, giving one example of each.
Why is the embryological evidence originally proposed by Ernst Haeckel no longer accepted as he stated it? What did Karl Ernst von Baer observe?
Arrange the following in correct sequence of appearance, oldest first: reptiles, jawless fish, first cellular life, amphibians, mammals, invertebrates.
Assertion–Reason. Assertion (A): Adaptive radiation and convergent evolution are the same process. Reason (R): In both, a single ancestral stock diversifies within one geographical area. Evaluate whether A and R are true and whether R explains A.
How do Darwin’s finches illustrate adaptive radiation? Explain the role played by beak shape.
Compare Lamarck’s and Darwin’s explanations for the long neck of the giraffe. Why is Lamarck’s explanation rejected today?
What is saltation? How did deVries’s view of the role of mutation in evolution differ from Darwin’s view of variation?
State the Hardy–Weinberg principle, including its conditions, and list the five factors that can disturb genetic equilibrium.
Why does a population that exactly obeys \(p^2 + 2pq + q^2 = 1\) in every generation indicate that no evolution is taking place?
Differentiate between gene flow and genetic drift. What is meant by the founder effect?
With the help of labelled bell-shaped curves, distinguish between stabilising, directional and disruptive natural selection.
Trace the change in brain size from Homo habilis through Homo erectus to the Neanderthals, and comment on what this trend suggests about their behaviour.
Why were reptiles able to colonise dry land more successfully than amphibians? Relate your answer to the structure of the reptilian egg.
“Evolution is not a directed process but a stochastic one.” Explain what this statement means, using an example from the chapter.
Draw and label a diagram of Miller’s apparatus, marking the electrodes, the spark discharge, the mixture of gases, the condenser, and the trap that collects the organic compounds.
6.14 Practice With Numericals
In a population of 2000 individuals living in Hardy–Weinberg equilibrium, 320 individuals show the recessive trait (genotype \(aa\)). Calculate the frequency of the recessive allele (\(q\)), the frequency of the dominant allele (\(p\)), and the number of heterozygous (\(Aa\)) individuals.
In a randomly mating population at Hardy–Weinberg equilibrium, the frequency of the dominant allele \(A\) is \(p = 0.7\). Find the expected percentages of the \(AA\), \(Aa\) and \(aa\) genotypes.
In a large population at equilibrium, 4% of individuals express a recessive genetic disorder. Assuming Hardy–Weinberg equilibrium, what fraction of the population are carriers (heterozygotes)?
In a plant population at Hardy–Weinberg equilibrium, the frequency of allele \(T\) is \(0.9\) and that of allele \(t\) is \(0.1\). Calculate the expected genotype frequencies of \(TT\), \(Tt\) and \(tt\).
A sample of 500 individuals contains 45 individuals with the genotype \(aa\). Assuming Hardy–Weinberg equilibrium, verify whether the frequency of the recessive allele is \(0.3\).