Chapter 13: Plant Growth and Development
High in the White Mountains of California grows a bristlecone pine known as Methuselah. It is not tall or grand to look at — twisted, gnarled, half its wood bleached silver by the wind. Yet this single tree has been alive for nearly five thousand years. It was already an old tree when the pyramids were being built. Not far away, in another Californian forest, stand the giant sequoias, trees so massive that a car could once be driven through a tunnel cut in one trunk.
What is astonishing is not just their size or their age, but that they are still growing. Every year, at the very tips of their branches and roots, and in a thin sleeve of tissue wrapped around their trunk, new cells are still being born. A human body stops growing in the late teens. A tree, it seems, never truly finishes.
And yet the same tree that grows for thousands of years drops all its needles and grows new ones on a far shorter cycle. One part of the plant grows without limit; another is renewed again and again. How can a single living thing hold both of these patterns at once? What decides when a plant grows, where it grows, and what shape it takes? These are the questions this chapter sets out to answer.
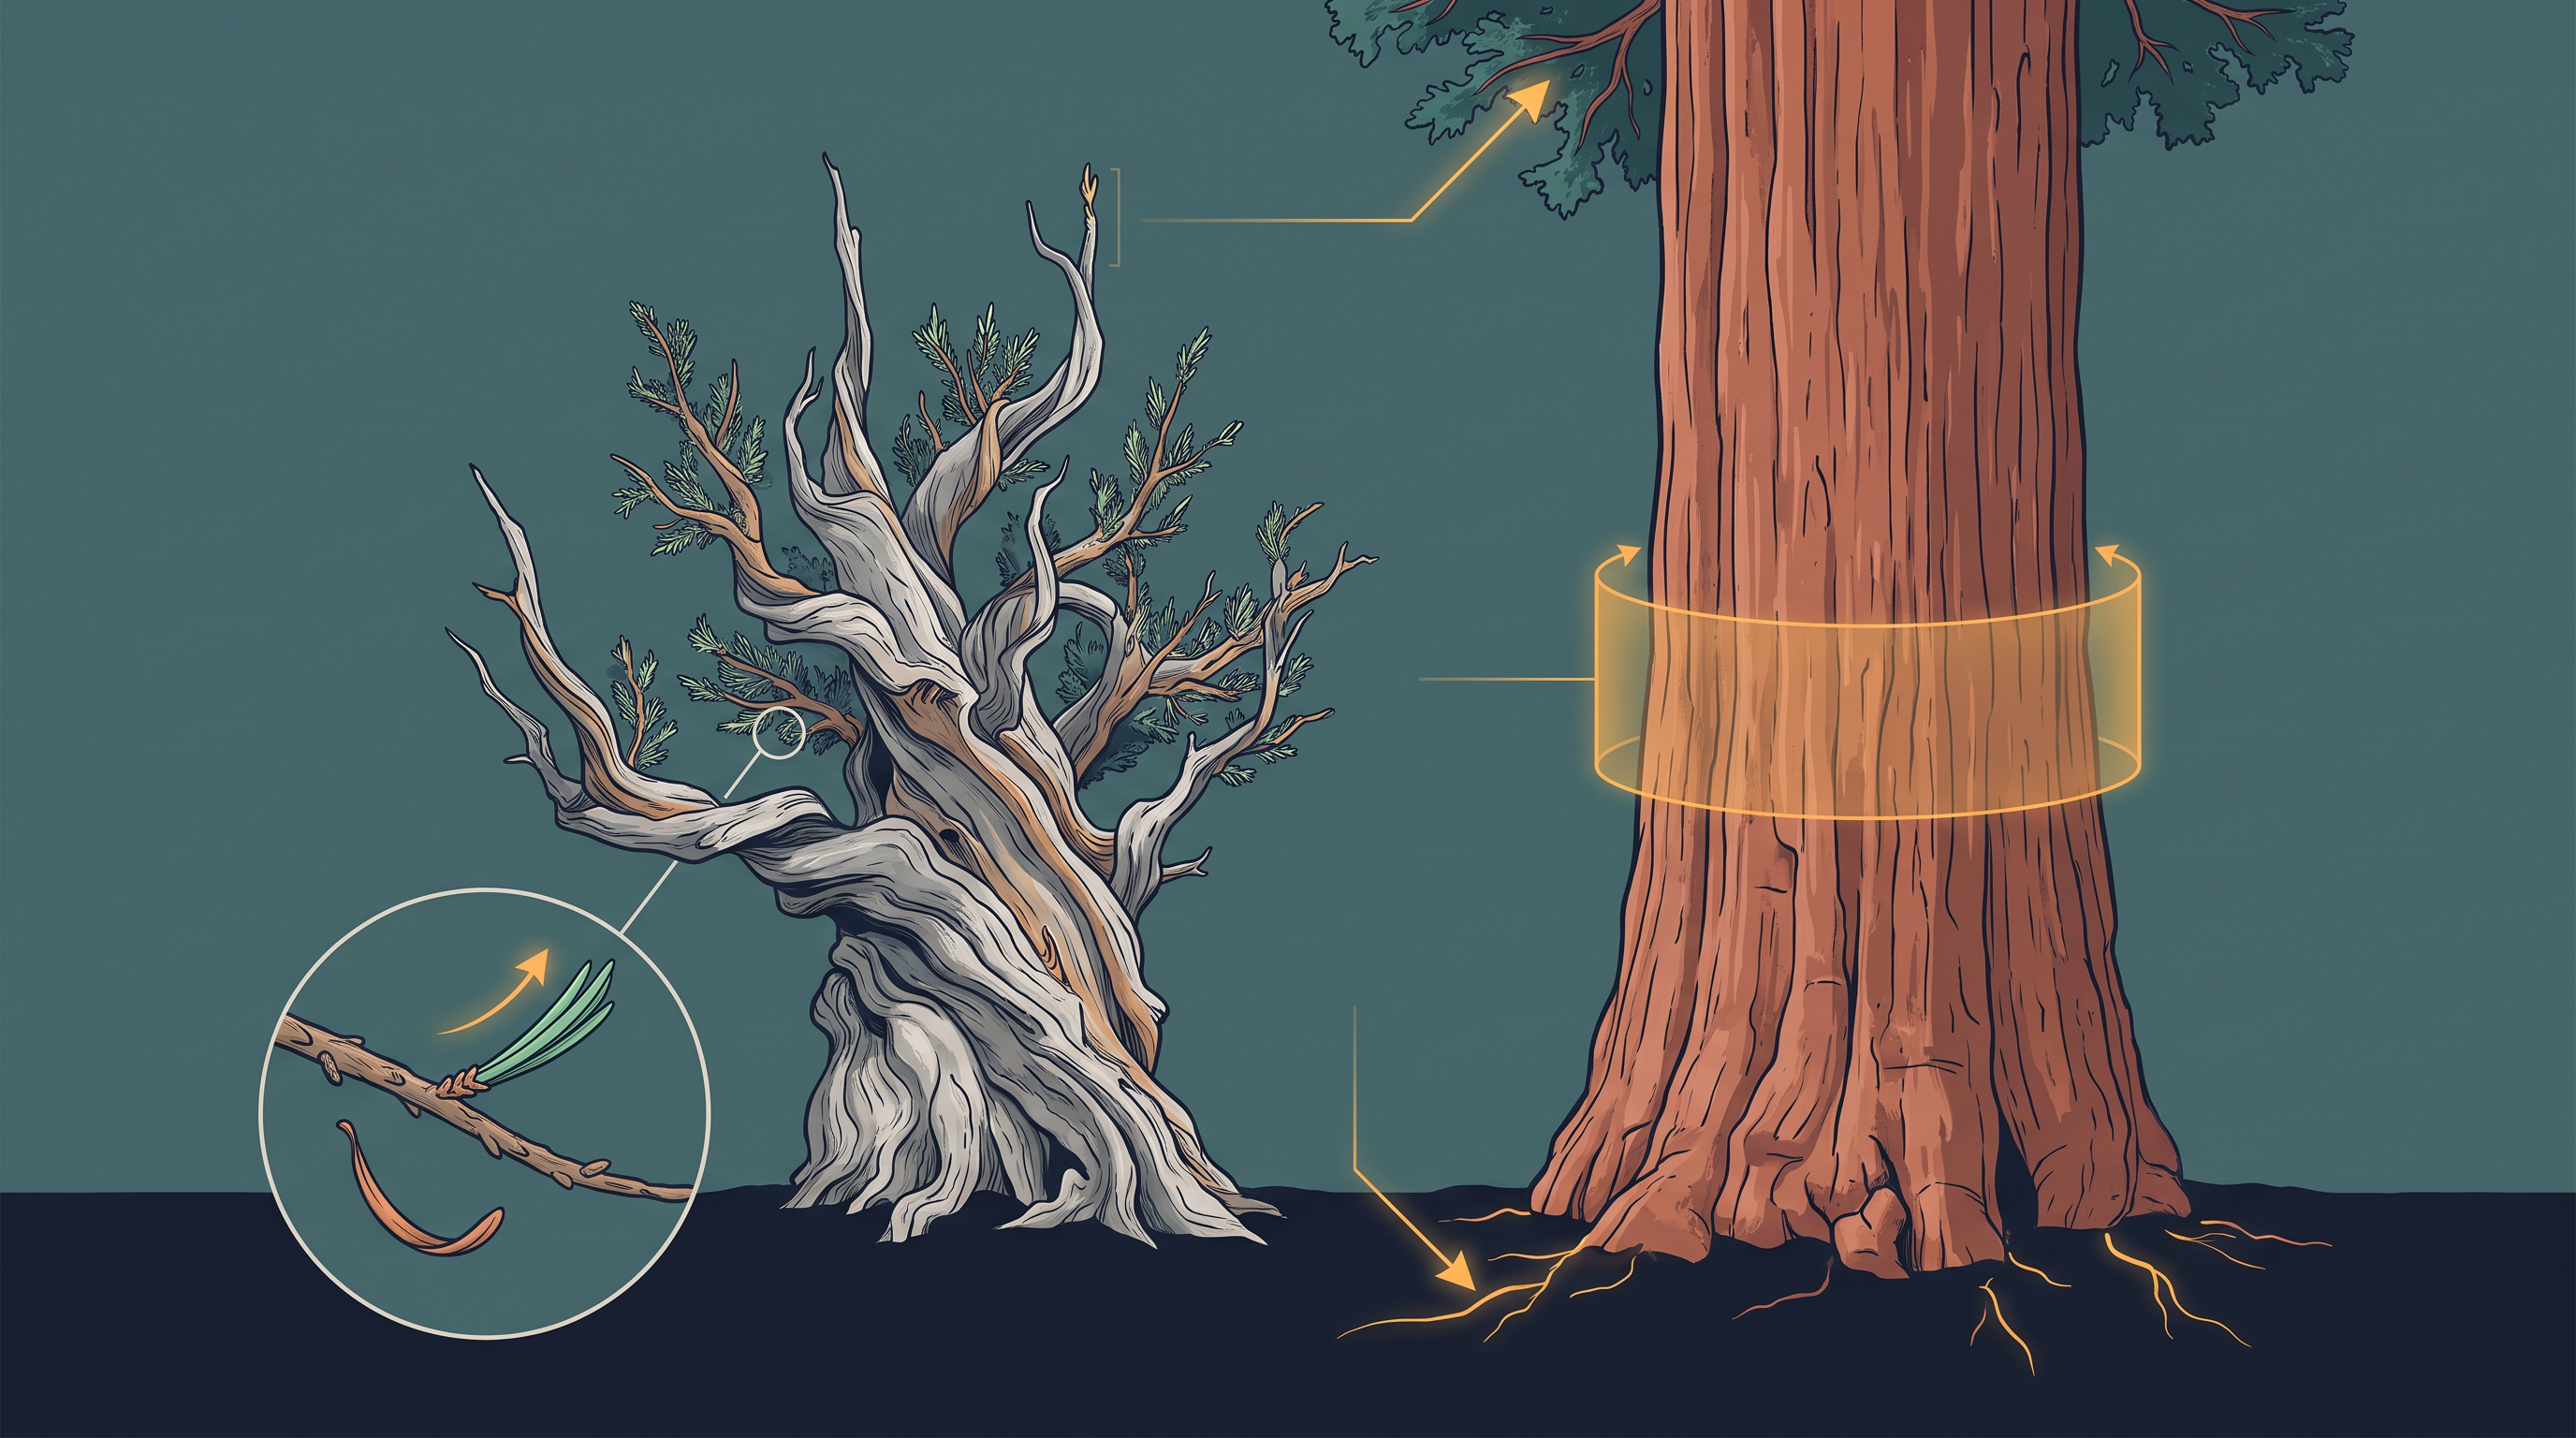
Fig. 13.0 – Growing points in ancient trees.
As you work through this chapter, keep these questions in mind — by the end, you will be able to answer every one of them.
13.1 Growth
From a Single Cell to a Whole Plant
In Chapter 5 you studied how a flowering plant is organised into roots, stems, leaves, flowers, fruits and seeds. But have you ever paused to ask where all these structures come from, and why they appear in such an orderly sequence? By now you are familiar with terms like seed, seedling, plantlet and mature plant, and you have seen that a tree keeps adding to its height and girth year after year.
Yet the leaves, flowers and fruits of that same tree behave quite differently. Each of them has a limited size, and each appears and falls at particular times, sometimes over and over again. Notice, too, that a plant almost always completes a vegetative (leafy) phase before it begins to flower. Why should the life of a plant follow such a fixed order?
Every organ of a plant is built from many kinds of tissues. This raises a deeper question: is there a link between the structure of a cell, a tissue or an organ and the job it performs — and can that structure and function ever be altered? The answer to this last question turns out to be yes, and it is one of the surprising things you will meet later in this chapter.
Remarkably, every single cell of a plant is a descendant of just one cell, the zygote — the fertilised egg formed after fertilisation. If they all share the same origin, why do they end up so different in form and function? The answer lies in a single idea: development.
Development is the sum of two processes — growth and differentiation. Starting from the zygote, a plant develops through a precise and highly ordered succession of events, gradually building a complex body of roots, leaves, branches, flowers, fruits and seeds — which eventually age and finally die. This entire sequence, from a seed to a leafy seedling, is shown for a bean plant in Fig. 13.1.
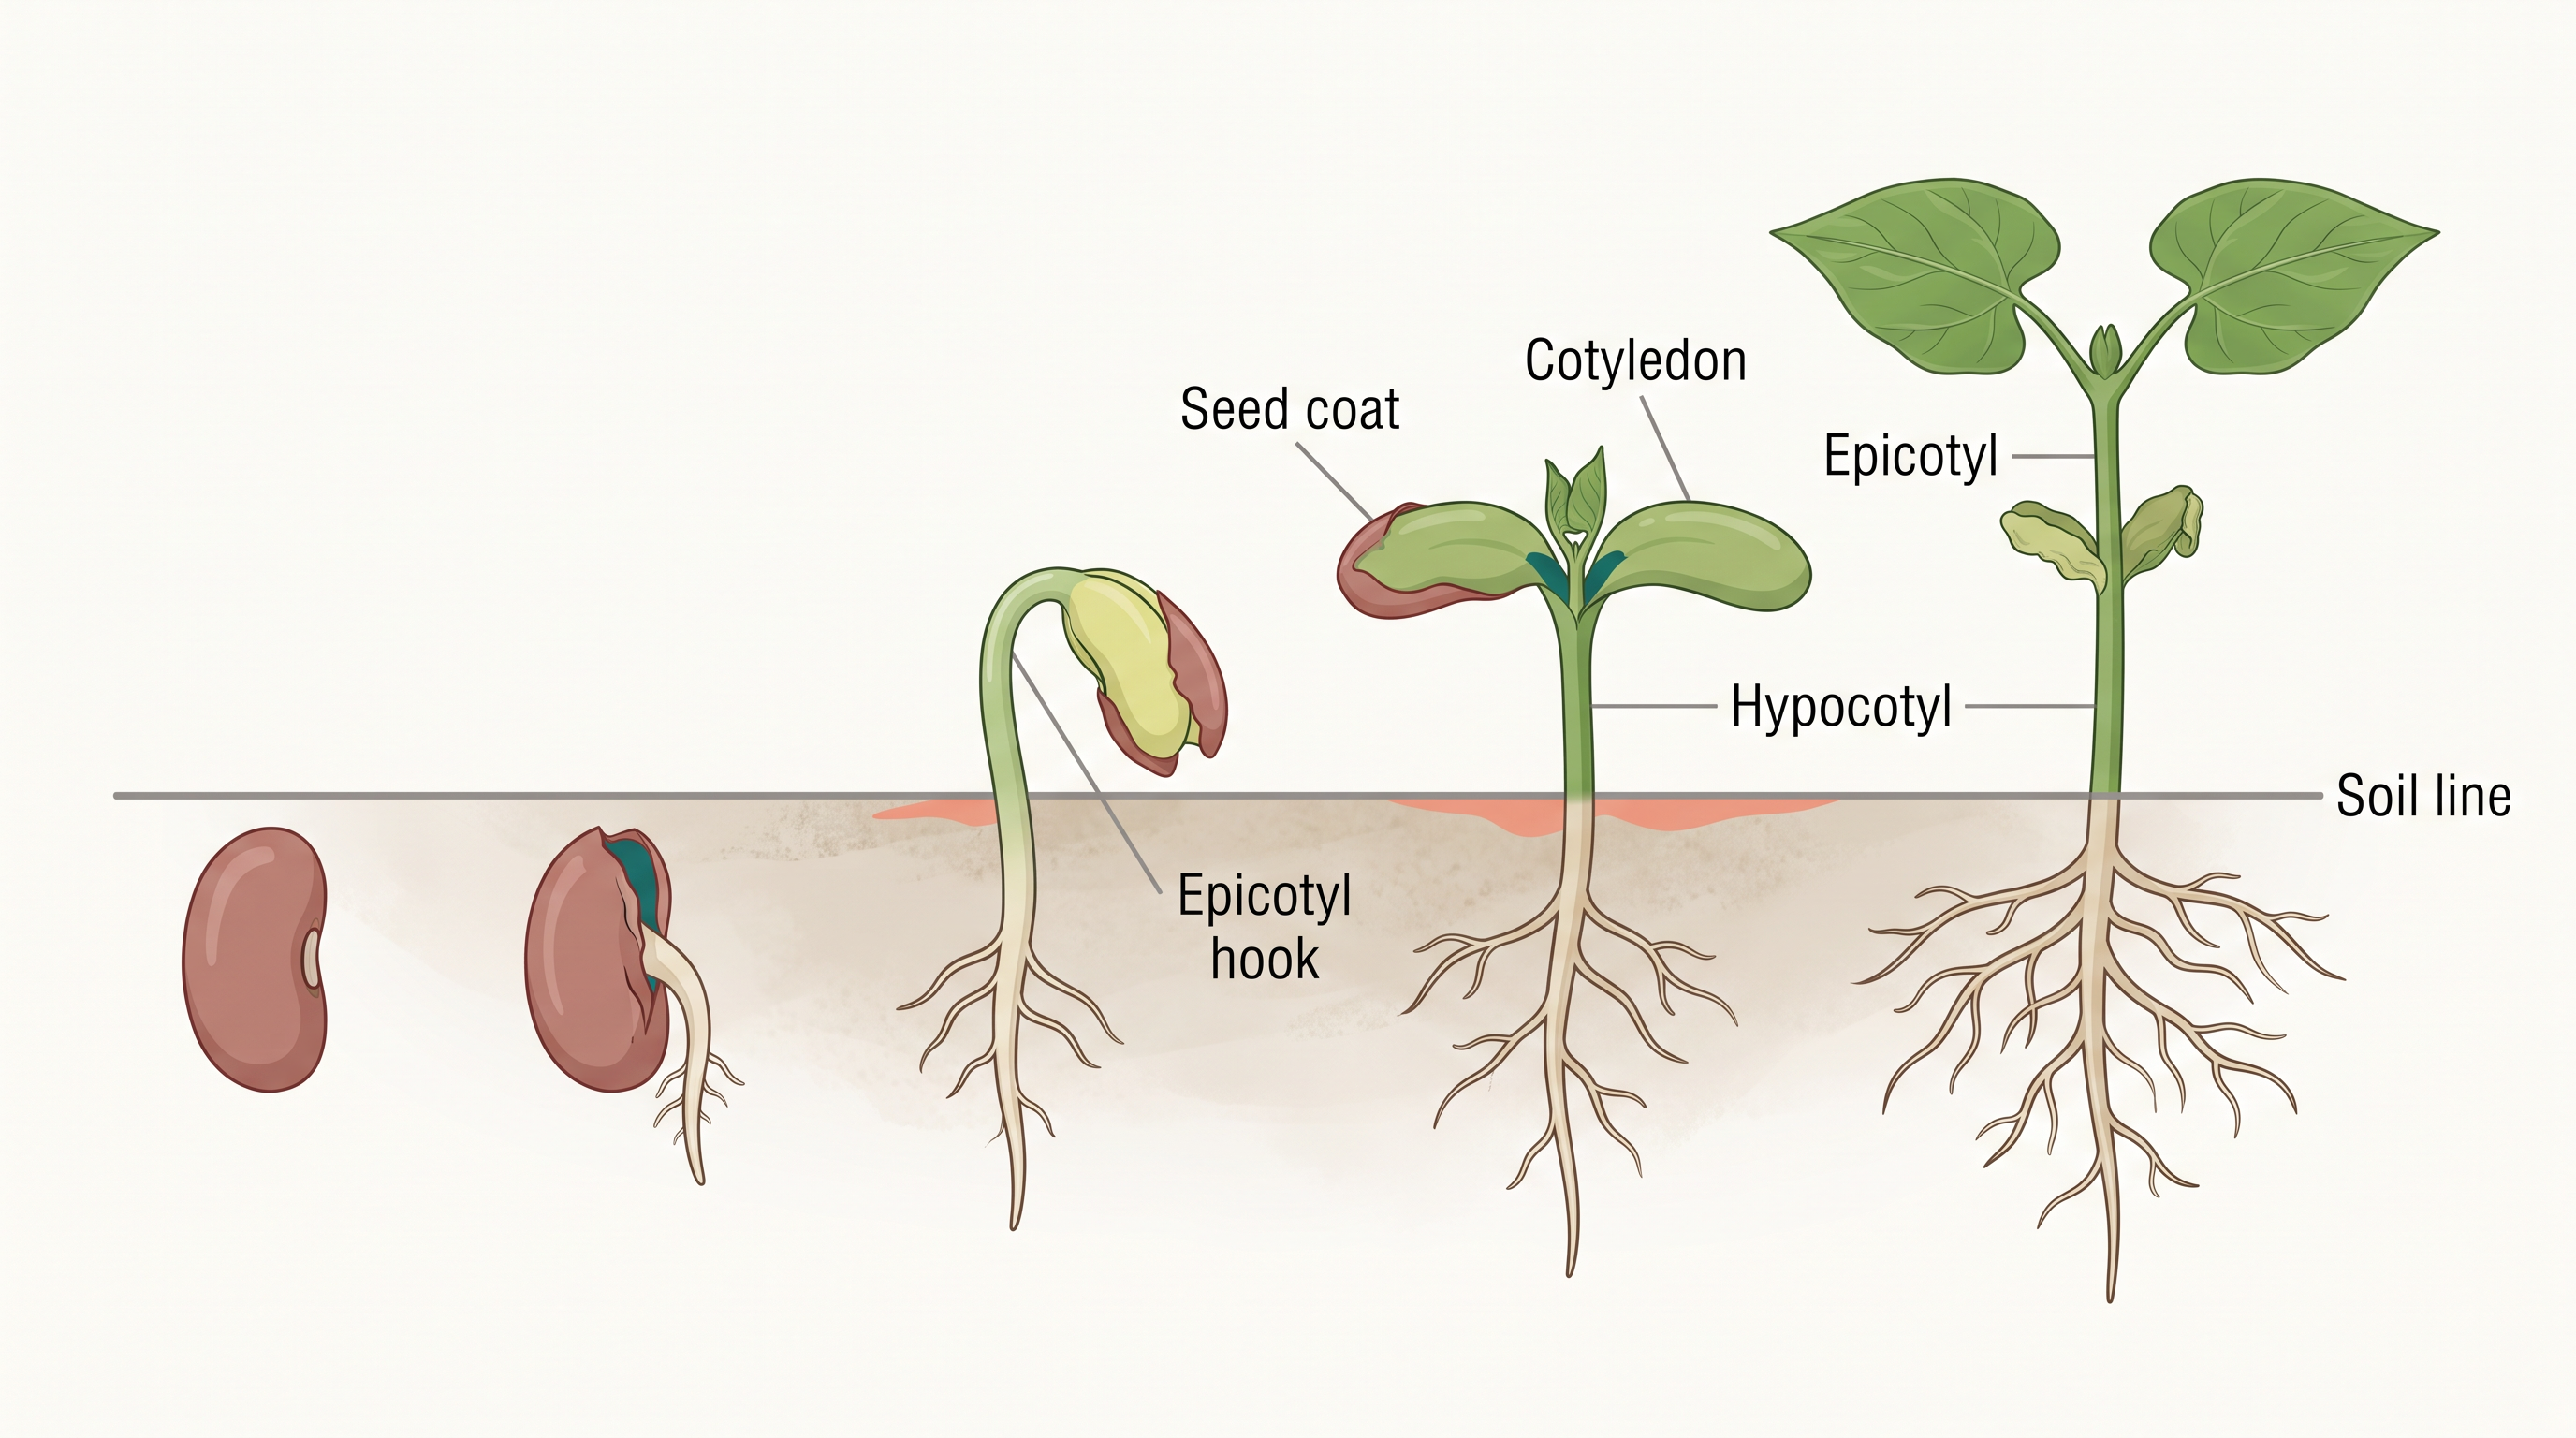
Fig. 13.1 – Germination and seedling development in a bean.
Germination: Where It All Begins
The very first step in the process of plant growth is seed germination — the seed “waking up” and beginning to grow into a seedling. Germination happens only when the conditions in the surroundings are favourable for growth.
If conditions are unfavourable, the seed does not germinate. Instead it enters a period of suspended growth, or rest, called dormancy. During dormancy the seed’s metabolic activity almost comes to a stop, which lets it wait out difficult times. Once favourable conditions return, the seed resumes its metabolic activities and growth begins.
All of these developmental processes are steered by two kinds of factors. Intrinsic (internal) factors arise from within the plant itself, while extrinsic (external) factors come from its surroundings. Later in this chapter you will study several of these controlling factors in detail.
What Exactly Is Growth?
Growth is one of the most fundamental and easily noticed features of any living organism. But it needs a careful definition, because not every increase in size actually counts as growth.
The word irreversible is the key. Growth is generally accompanied by metabolic processes that take place at the expense of energy. These processes are of two kinds working side by side — anabolic reactions, which build up complex molecules (synthesis), and catabolic reactions, which break molecules down to release energy. Because new living material is actually being made and added, the increase in size cannot simply be undone. The expansion of a leaf, for instance, is true growth.
13.1.1 Plant Growth Generally is Indeterminate
Growth Without a Fixed Limit
Plant growth is unusual, and this is one of the things that sets plants apart from animals. An animal grows to a certain size and then stops — an adult dog or human does not keep getting taller year after year. A plant, in contrast, can keep on growing for the whole of its life. This capacity for unlimited or indeterminate growth is a special feature of plants.
How is this possible? It is due to the presence of meristems — small regions of dividing tissue found at particular locations in the plant body.
The cells of a meristem do two things at once: they divide, and they self-perpetuate. This means that when a meristematic cell divides, some of its products stay meristematic — keeping the ability to divide and renewing the meristem — while the other products soon lose the ability to divide, mature, and go on to build the actual body of the plant.
Because new cells are being added to the plant body again and again by the continuous activity of the meristem, this pattern is called the open form of growth.
Where the Meristems Sit: Length versus Girth
In earlier classes you studied two important meristems — the root apical meristem, at the tip of the root, and the shoot apical meristem, at the tip of the shoot. These apical meristems are responsible for the primary growth of the plant, and they mainly cause the plant to grow longer along its axis, as shown in Fig. 13.2.
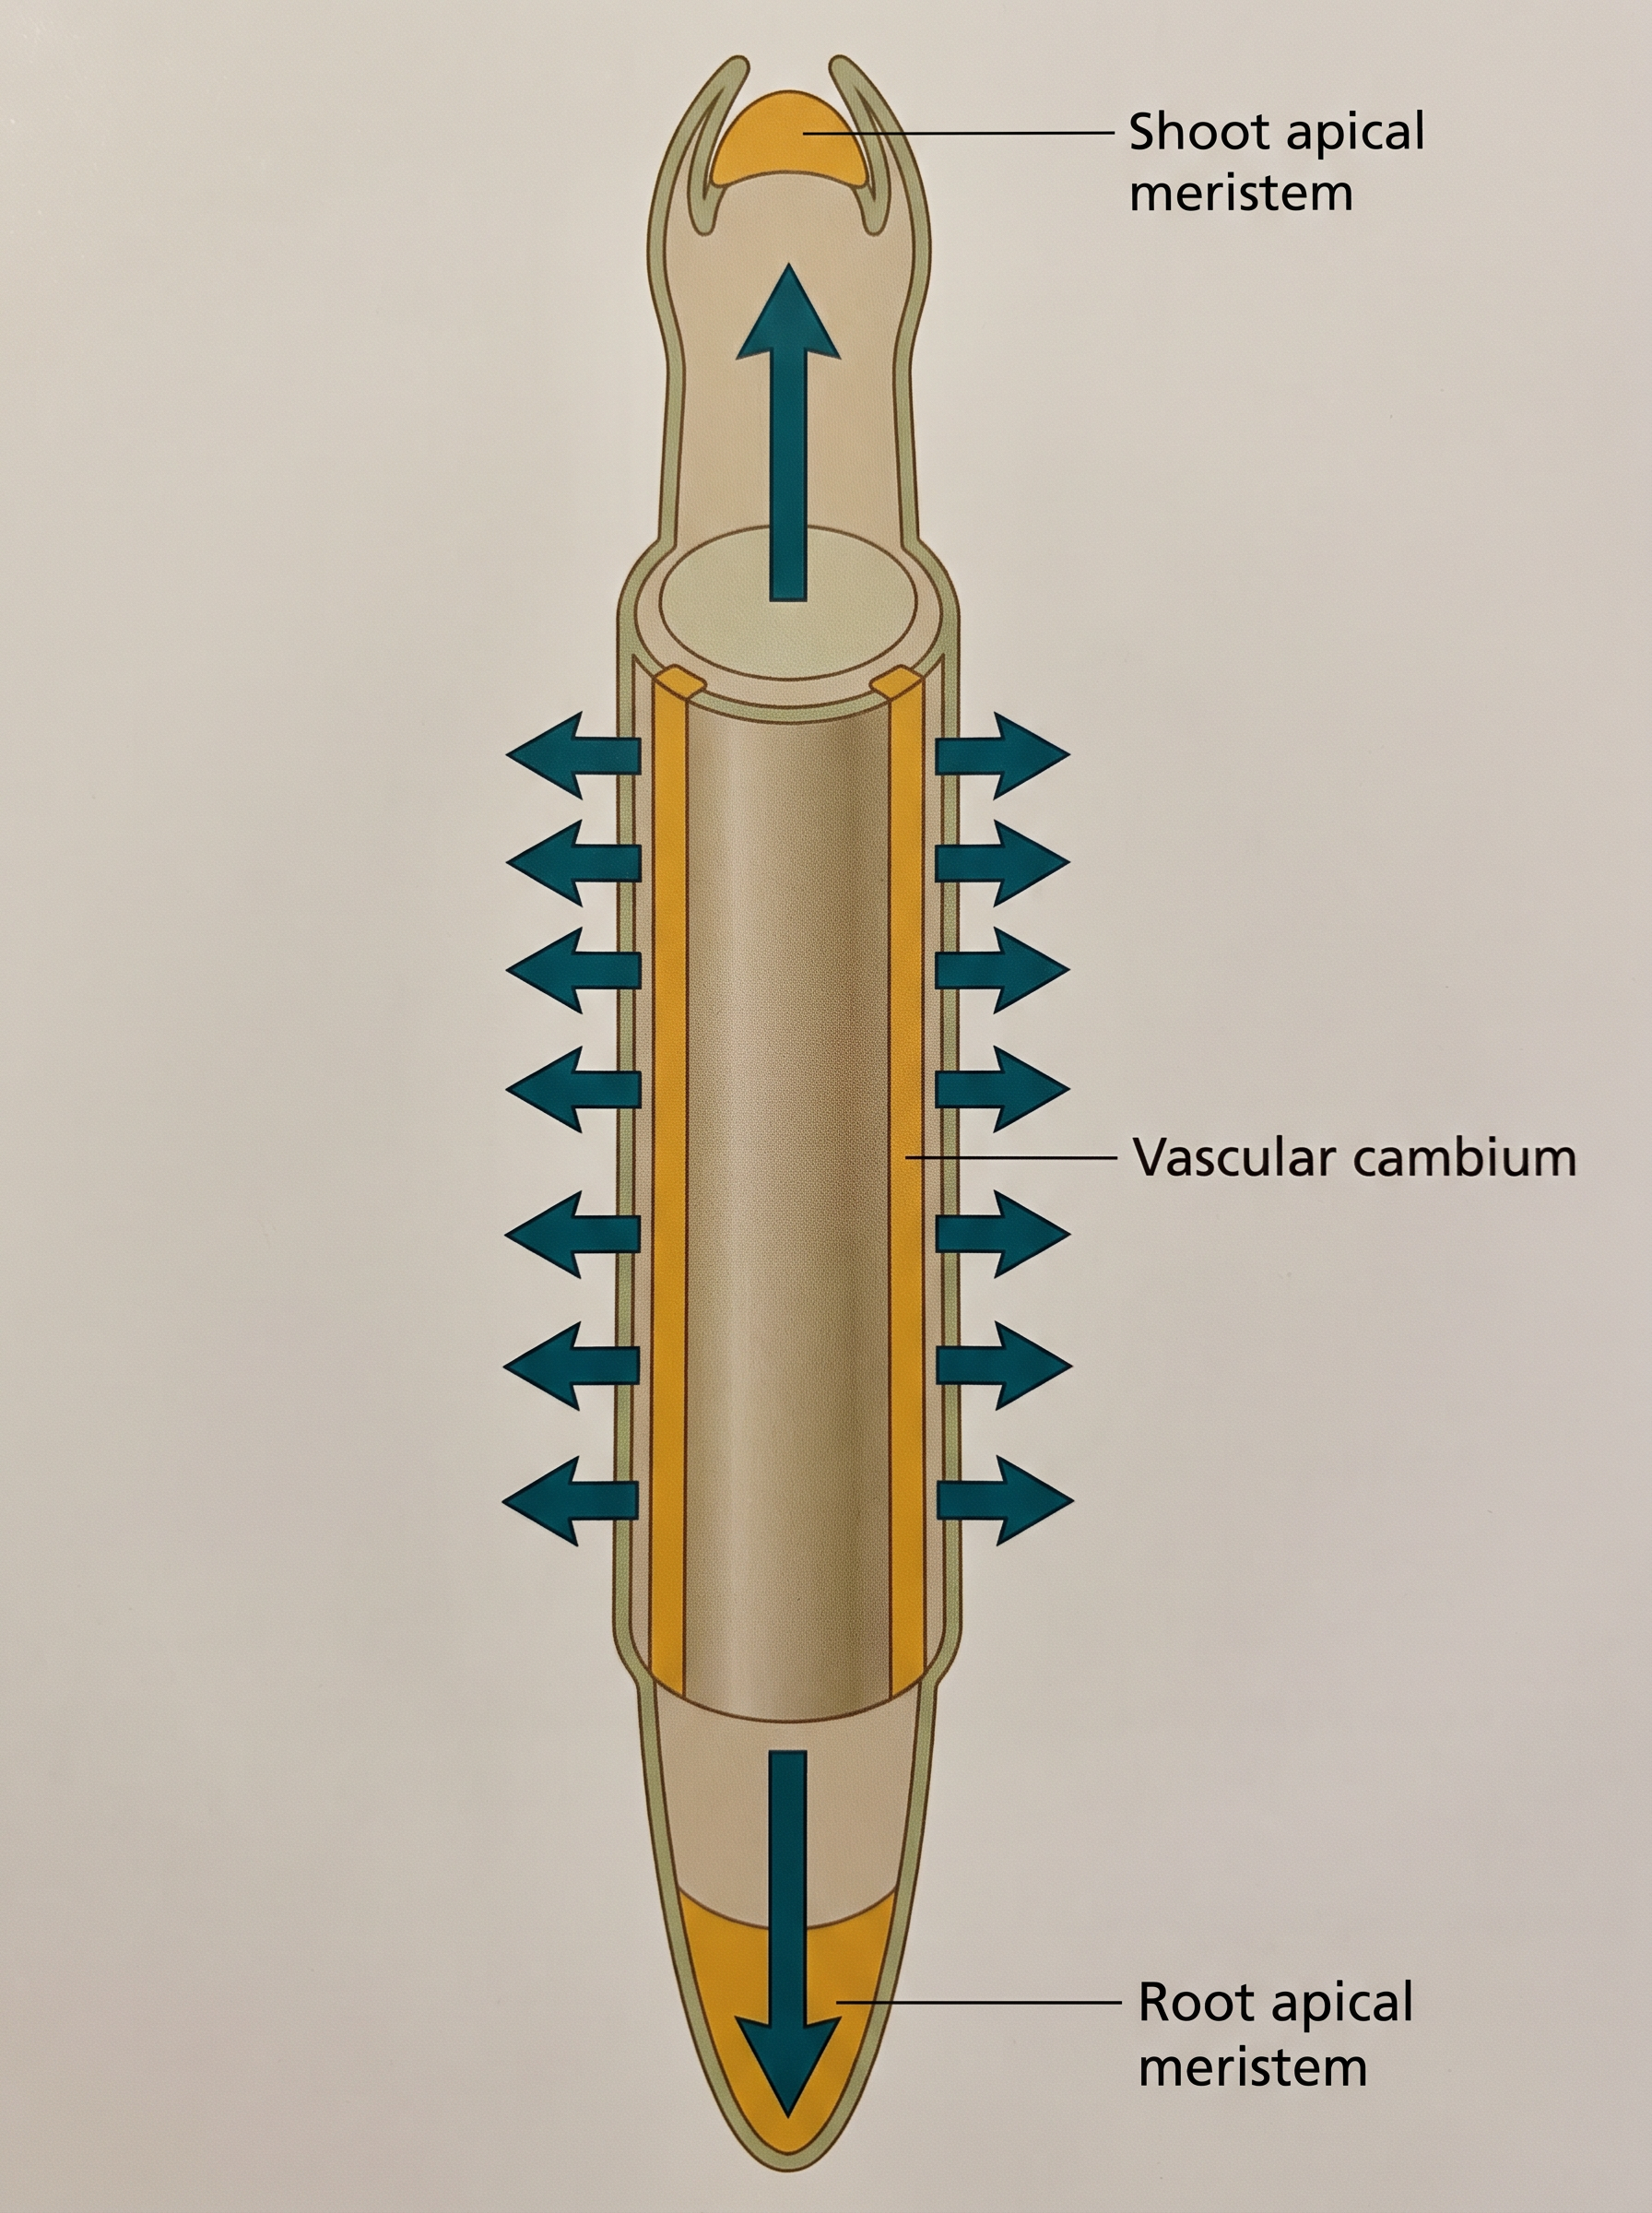
Fig. 13.2 – Locations of the principal meristems in a plant.
In dicotyledonous plants and in gymnosperms, another set of meristems appears later in the plant’s life. These are the lateral meristems — the vascular cambium and the cork-cambium. They lie along the sides of the stem and root, and their activity increases the girth (thickness) of the organs in which they are active. This is called the secondary growth of the plant.
13.1.2 Growth is Measurable
The Root of Growth: More Protoplasm
At the level of a single cell, growth comes down mostly to one thing — an increase in the amount of protoplasm. Protoplasm is the living material inside a cell (the cytoplasm together with the nucleus), so making more of it is really what “growing” means for a cell.
The trouble is that the amount of protoplasm is very difficult to measure directly. So, in practice, we measure some other quantity that is more or less proportional to it and use that as a stand-in for growth.
A variety of such parameters can be used. Growth may be measured as an increase in fresh weight, dry weight, length, area, volume, or cell number — whichever is easiest and most meaningful for the system being studied.
Different Systems, Different Yardsticks
Which parameter we choose depends on how a particular structure actually grows. Some structures grow mainly by making more cells; others grow mainly by making their existing cells bigger.
Consider two striking examples. A single maize root apical meristem can give rise to more than 17,500 new cells per hour. A watermelon, on the other hand, grows because its cells may increase in size by up to 3,50,000 times.
In the maize root, then, growth is best expressed as an increase in cell number, because it is division that drives it. In the watermelon, growth is best expressed as an increase in the size of the cells, because it is enlargement that drives it.
Two more examples show how the choice of parameter follows the shape of the growth. The growth of a pollen tube — a slender tube that grows in one direction — is measured in terms of its length. But for a dorsiventral leaf (a flat leaf with clearly distinct upper and lower surfaces), which spreads out sideways as it grows, an increase in surface area is the parameter that best describes its growth.
13.1.3 Phases of Growth
The period of growth in a plant is generally divided into three phases, one following the other: the meristematic phase, the elongation phase and the maturation phase. The easiest place to see all three at once is a root tip, where the three zones lie neatly one behind the other, as shown in Fig. 13.3. The whole sequence is summarised in FC 13.1.
Flowchart
FC 13.1 – Phases of growth along a root tip, from the apex inward: Meristematic phase (constantly dividing cells) → Elongation phase (vacuolation, cell enlargement, new wall deposition) → Maturation phase (wall thickening, protoplasmic modification, cells reach final form).
Meristematic Phase
Right at the root apex and the shoot apex are the constantly dividing cells — these make up the meristematic phase. The cells here are rich in protoplasm and have large, conspicuous nuclei, as befits cells that are busy dividing.
Their cell walls are primary in nature — that is, thin, freshly formed and made of cellulose. These cells are also linked to one another by abundant plasmodesmata, the fine cytoplasmic channels that pass through the cell walls and connect neighbouring cells.
Elongation Phase
The cells lying just next to the meristematic zone — proximal to it, meaning a little further away from the tip — represent the phase of elongation. Here the cells stop dividing and start getting bigger.
Three changes mark this phase: increased vacuolation (the cells develop and enlarge their vacuoles), cell enlargement, and the deposition of new cell wall material. The swelling vacuoles take in water and push the cell to expand, which is what actually lengthens the root behind the tip.
Maturation Phase
Further away still from the apex — beyond the elongation zone — lies the portion of the axis in the maturation phase. The cells of this zone attain their maximal size, and now show wall thickening and various protoplasmic modifications that fit them for their final jobs.
Most of the tissues and cell types you studied in earlier classes belong to this phase, because it is here that cells finish becoming specialised.
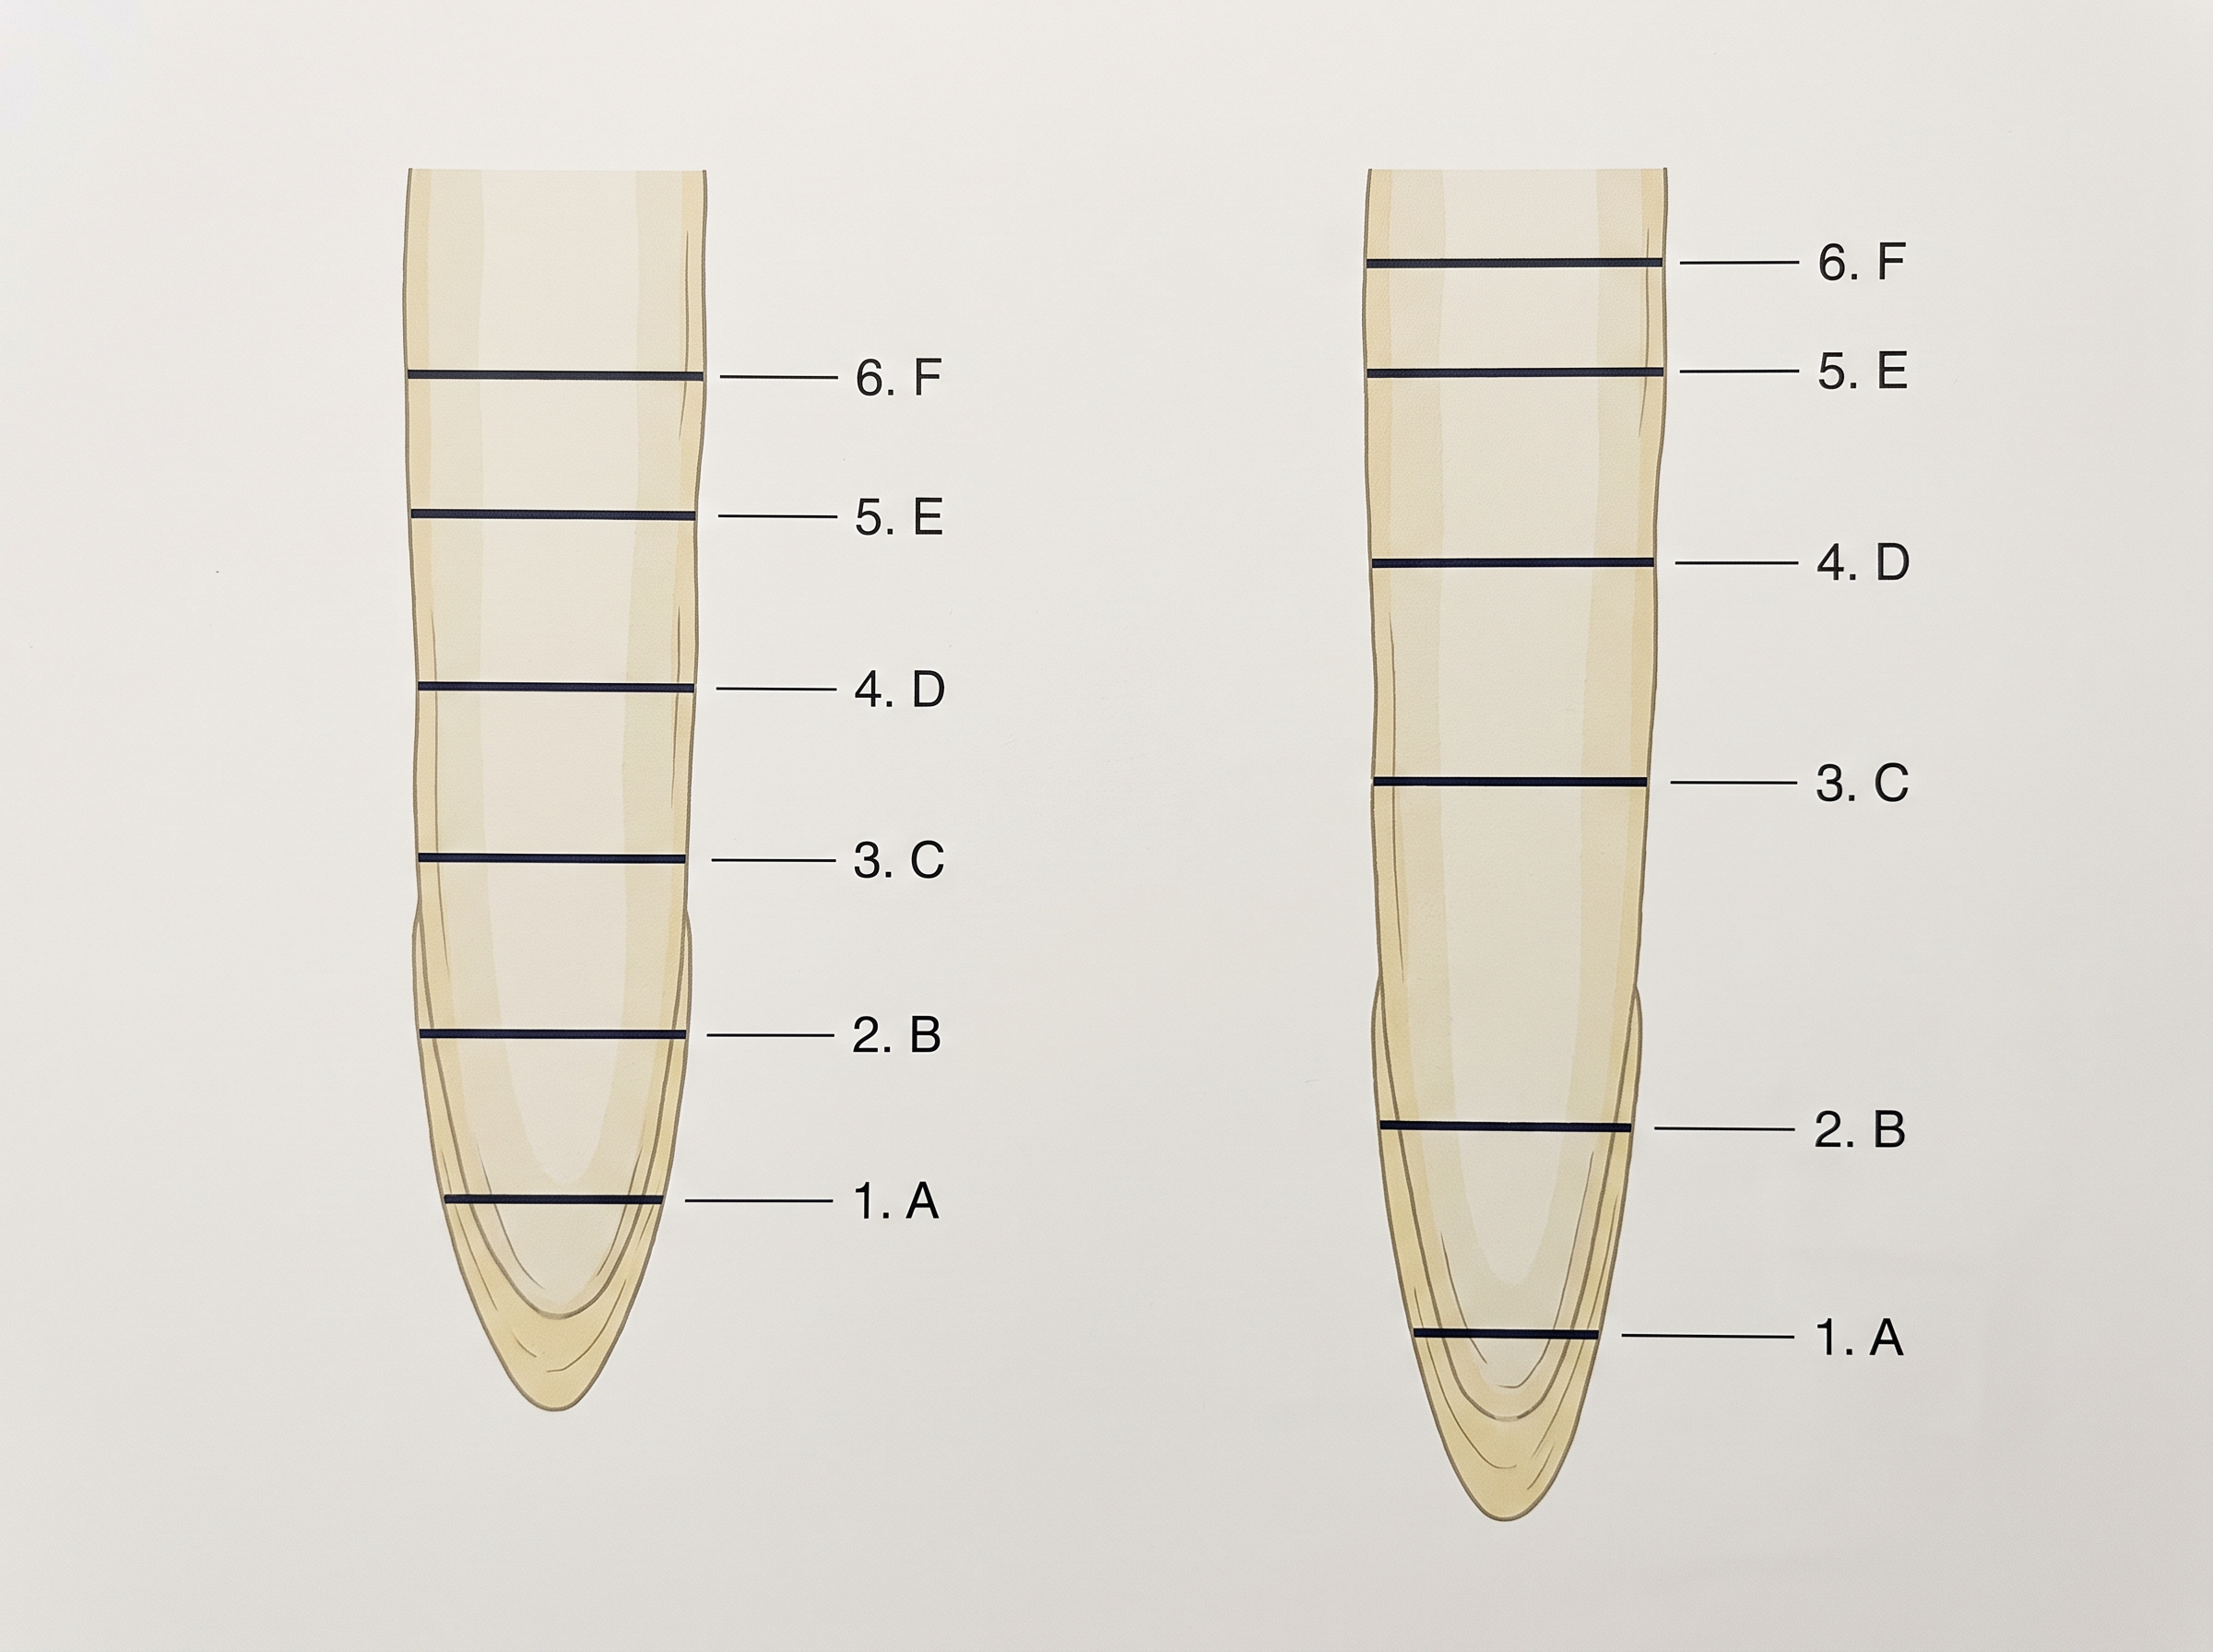
Fig. 13.3 – Detection of the zone of elongation by the parallel-line technique.
The parallel-line technique in Fig. 13.3 makes this visible: when equally spaced lines are drawn on a growing root, the marks just behind the tip (zones A, B, C, D) move apart the most, proving that this is where elongation is greatest.
13.1.4 Growth Rates
The increased growth per unit time is called the growth rate. Because it is “amount of growth divided by time,” the rate of growth can be written down mathematically. An organism, or a part of it, can produce more cells in more than one way — and this leads to two different patterns of growth rate: arithmetic and geometrical, both shown in Fig. 13.4.
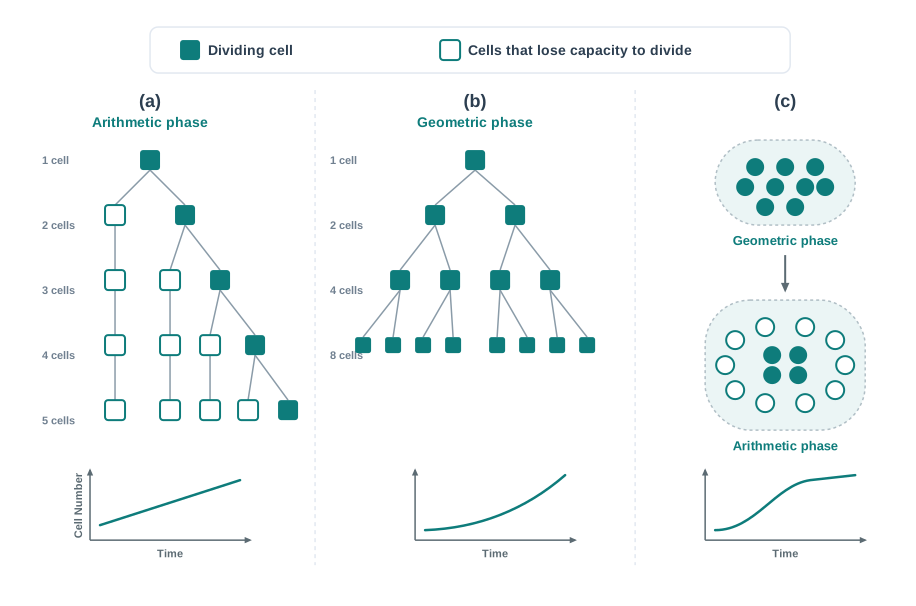
Fig. 13.4 – Arithmetic and geometric growth models.
Arithmetic Growth
In arithmetic growth, after a cell divides by mitosis, only one of the two daughter cells continues to divide, while the other daughter cell differentiates and matures. So the number of actively dividing cells stays the same, and growth adds up at a steady, constant rate.
The simplest example is a root that elongates at a constant rate. If you plot the length of such a root against time, you get a straight line, as in Fig. 13.5. Mathematically, arithmetic growth is expressed as:
\[L_t = L_0 + rt\]
Here \(L_t\) is the length at time \(t\) (measured, for example, in mm or cm), \(L_0\) is the length at time zero (the starting length), and \(r\) is the growth rate, that is, the elongation per unit time (for example, mm per day). Because \(r\) is constant, the graph is a straight line.
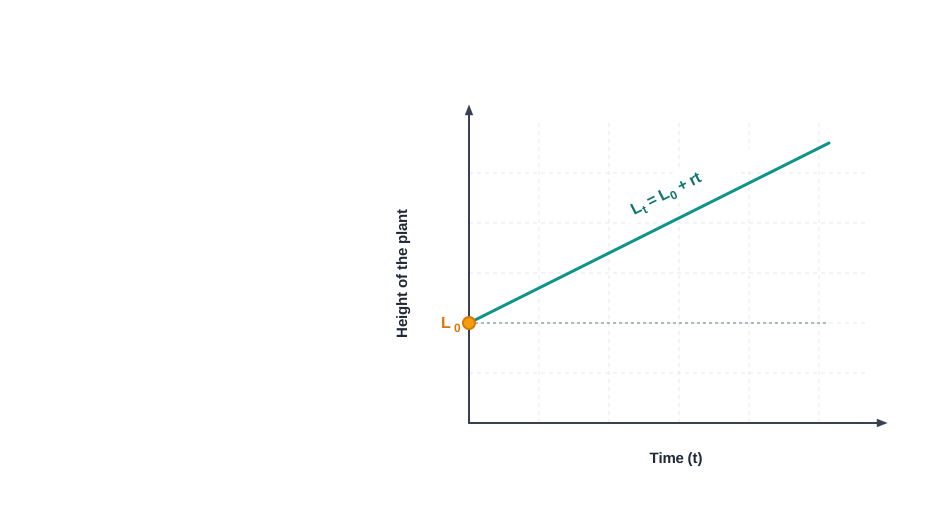
Fig. 13.5 – Constant linear growth over time.
Geometric Growth
Geometric growth is different, because here both daughter cells produced by mitosis keep the ability to divide, and they go on dividing. This makes the number of dividing cells multiply, so growth speeds up dramatically over time.
In most living systems this growth follows a recognisable pattern. At first growth is slow — this is the lag phase. Then it speeds up and increases rapidly at an exponential rate — the log phase (also called the exponential phase). Finally, because nutrients are limited and cannot support unlimited multiplication, growth slows down and levels off into a stationary phase.
If you plot the growth parameter against time, these three phases together trace out a typical sigmoid curve, or S-curve, shown in Fig. 13.6. This S-shaped curve is characteristic of a living organism growing in its natural environment, and it is typical of all the cells, tissues and organs of a plant.
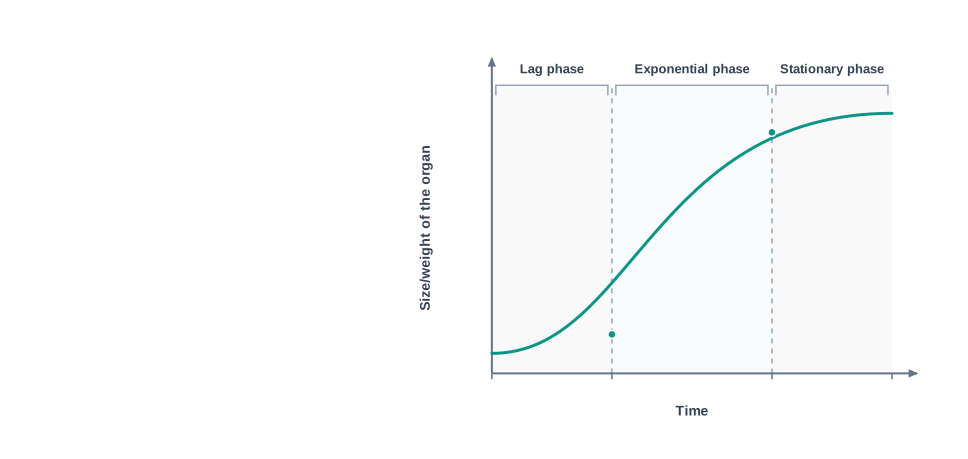
Fig. 13.6 – An idealised sigmoid growth curve.
Exponential (geometric) growth is expressed as:
\[W_1 = W_0 e^{rt}\]
Here \(W_1\) is the final size (weight, height, number, and so on), \(W_0\) is the initial size at the beginning of the period, \(r\) is the growth rate, \(t\) is the time of growth, and \(e\) is the base of natural logarithms (approximately \(2.718\)).
In this equation, \(r\) is the relative growth rate. It is also a measure of the plant’s ability to produce new plant material, and for this reason it is called the efficiency index. Notice from the equation that the final size \(W_1\) depends on the initial size \(W_0\) — a bigger starting point leads to a bigger final size for the same \(r\) and \(t\).
Comparing Growth: Absolute versus Relative
There are two useful ways to compare the growth of living systems.
Why do we need both? Because a small structure and a large structure can add the same absolute amount, yet the smaller one has grown far more relative to its own size. In Fig. 13.7, two leaves A and B of different sizes each increase their area by the same amount in the same time to give leaves A¹ and B¹ — so their absolute growth is equal. But one of them shows a much higher relative growth rate.
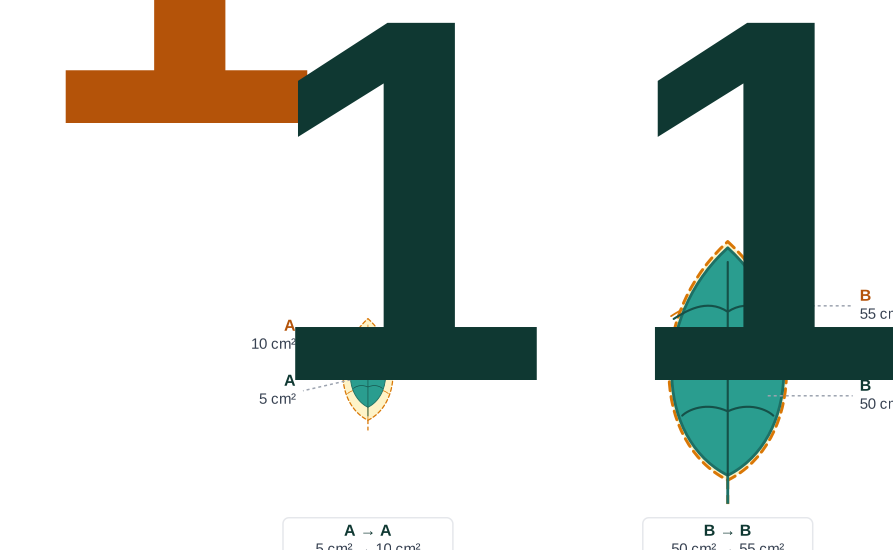
Fig. 13.7 – Comparison of absolute and relative growth rates.
13.1.5 Conditions for Growth
Before a plant can grow, certain conditions must be met. If you tried to list them yourself, you would almost certainly include water, oxygen and nutrients — and you would be right, because these are the most essential requirements. Along with them, the right temperature and certain environmental signals also matter.
Water
Plant cells grow in size mainly by cell enlargement, and this needs water. When a cell takes in water it becomes turgid — firm and swollen due to the water pressure inside it — and this turgidity is what drives extension growth (the stretching and lengthening of cells). For this reason, plant growth and further development are closely tied to the water status of the plant.
Water plays a second role too. It provides the medium in which enzymatic activities take place. Enzymes are proteins that speed up the chemical reactions of the cell, and these reactions, which are needed for growth, can only proceed in a watery environment.
Oxygen
Oxygen is required because it helps release the metabolic energy that growth activities depend on. Without enough oxygen, the cell cannot free up the energy it needs to build new material.
Nutrients
Nutrients — both the macro (needed in large amounts) and micro (needed in small amounts) essential elements — are required by plants for two purposes. They supply the raw materials for the synthesis of protoplasm, the living material of new cells, and they also act as a source of energy.
Temperature and Environmental Signals
Every plant has an optimum temperature range that is best suited to its growth. Any large deviation from this range can be harmful, and may even threaten the plant’s survival.
Finally, environmental signals such as light and gravity also influence growth. They do not act on every process, but they affect certain particular phases or stages of growth, as you will see later in the chapter.
13.2 Differentiation, Dedifferentiation and Redifferentiation
Differentiation: Cells Take On a Job
The cells produced by the root apical meristem, the shoot apical meristem and the cambium do not stay simple and unspecialised. They mature and take on particular jobs in the plant body. This act of maturing to perform a specific function is called differentiation.
During differentiation, a cell undergoes structural changes — sometimes small, sometimes major — in both its cell walls and its protoplasm. A striking example is the formation of a tracheary element, one of the water-conducting cells of the xylem. To become such a cell, the cell loses its protoplasm entirely, ending up hollow and dead. It also lays down a very strong, elastic, lignocellulosic secondary cell wall — a thick wall containing lignin (a tough strengthening material) along with cellulose.
Whenever you meet an anatomical feature in a plant, it is worth pausing to ask how its structure suits the function it performs — differentiation is exactly what forges that link between form and function.
Dedifferentiation: Regaining the Power to Divide
Plants can do something surprising. A living, differentiated cell that has already lost the capacity to divide can, under certain conditions, get that capacity back. This phenomenon is called dedifferentiation.
For example, fully differentiated parenchyma cells (parenchyma is a simple, living, thin-walled plant tissue) can dedifferentiate to form new meristems — the interfascicular cambium and the cork cambium. In doing so, these ordinary cells become dividing tissue once again.
Redifferentiation: Maturing Once More
The story does not end there. The meristems and tissues formed by dedifferentiation divide and produce new cells — and these new cells, in turn, once again lose the capacity to divide and mature to perform specific functions. This second round of maturation is called redifferentiation.
The whole cycle — differentiation, then dedifferentiation, then redifferentiation — is summarised in FC 13.2.
Flowchart
FC 13.2 – Meristematic cell → differentiates (structural changes in wall and protoplasm; loses capacity to divide; matures for a function) → under certain conditions, dedifferentiates (regains capacity to divide; forms a new meristem, e.g., interfascicular cambium or cork cambium) → divides → redifferentiates (new cells again lose capacity to divide; mature to perform specific functions).
Differentiation in Plants is Open
Recall from Section 13.1.1 that growth in plants is open — it can be either indeterminate or determinate. We can now say that even differentiation in plants is open. This is because cells and tissues arising from the same meristem can end up with quite different structures at maturity.
What decides the final structure of a cell, then? A major factor is the location of the cell within the organ. For example, cells positioned away from the root apical meristem differentiate into root-cap cells, while cells pushed towards the periphery mature into epidermis — even though both came from the same meristem.
13.3 Development
What Development Means
Growth and differentiation together are part of a bigger idea. Development is the broad term that covers every change an organism passes through during its life cycle — right from the germination of the seed all the way to senescence, the ageing phase that leads finally to death.
The sequence of steps that make up the development of a single cell of a higher plant is set out in FC 13.3. Importantly, this same sequence applies not only to a cell but also to tissues and organs.
Flowchart
FC 13.3 – Sequence of the developmental process in a plant cell: Meristematic cell → cell division → plasmatic growth → differentiation → expansion (elongation) → maturation → mature cell → senescence → death.
In this sequence, plasmatic growth refers to the increase in the cell’s protoplasm, while senescence is the final ageing of the mature cell before it dies. So a cell is “born” in a meristem, grows and specialises, does its job as a mature cell, and eventually ages and dies — a complete life story in miniature.
Plasticity: One Plant, Many Forms
Plants have a remarkable flexibility in how they develop. Depending on the environment, or on the phase of life they are in, plants can follow different pathways to form different kinds of structures. This ability is called plasticity.
A clear example of plasticity is heterophylly, where a plant bears leaves of more than one shape. In cotton, coriander and larkspur, the leaves of the juvenile (young) plant differ in shape from those of the mature plant — here the different leaf forms are linked to the plant’s phase of life, as shown for larkspur in Fig. 13.8.
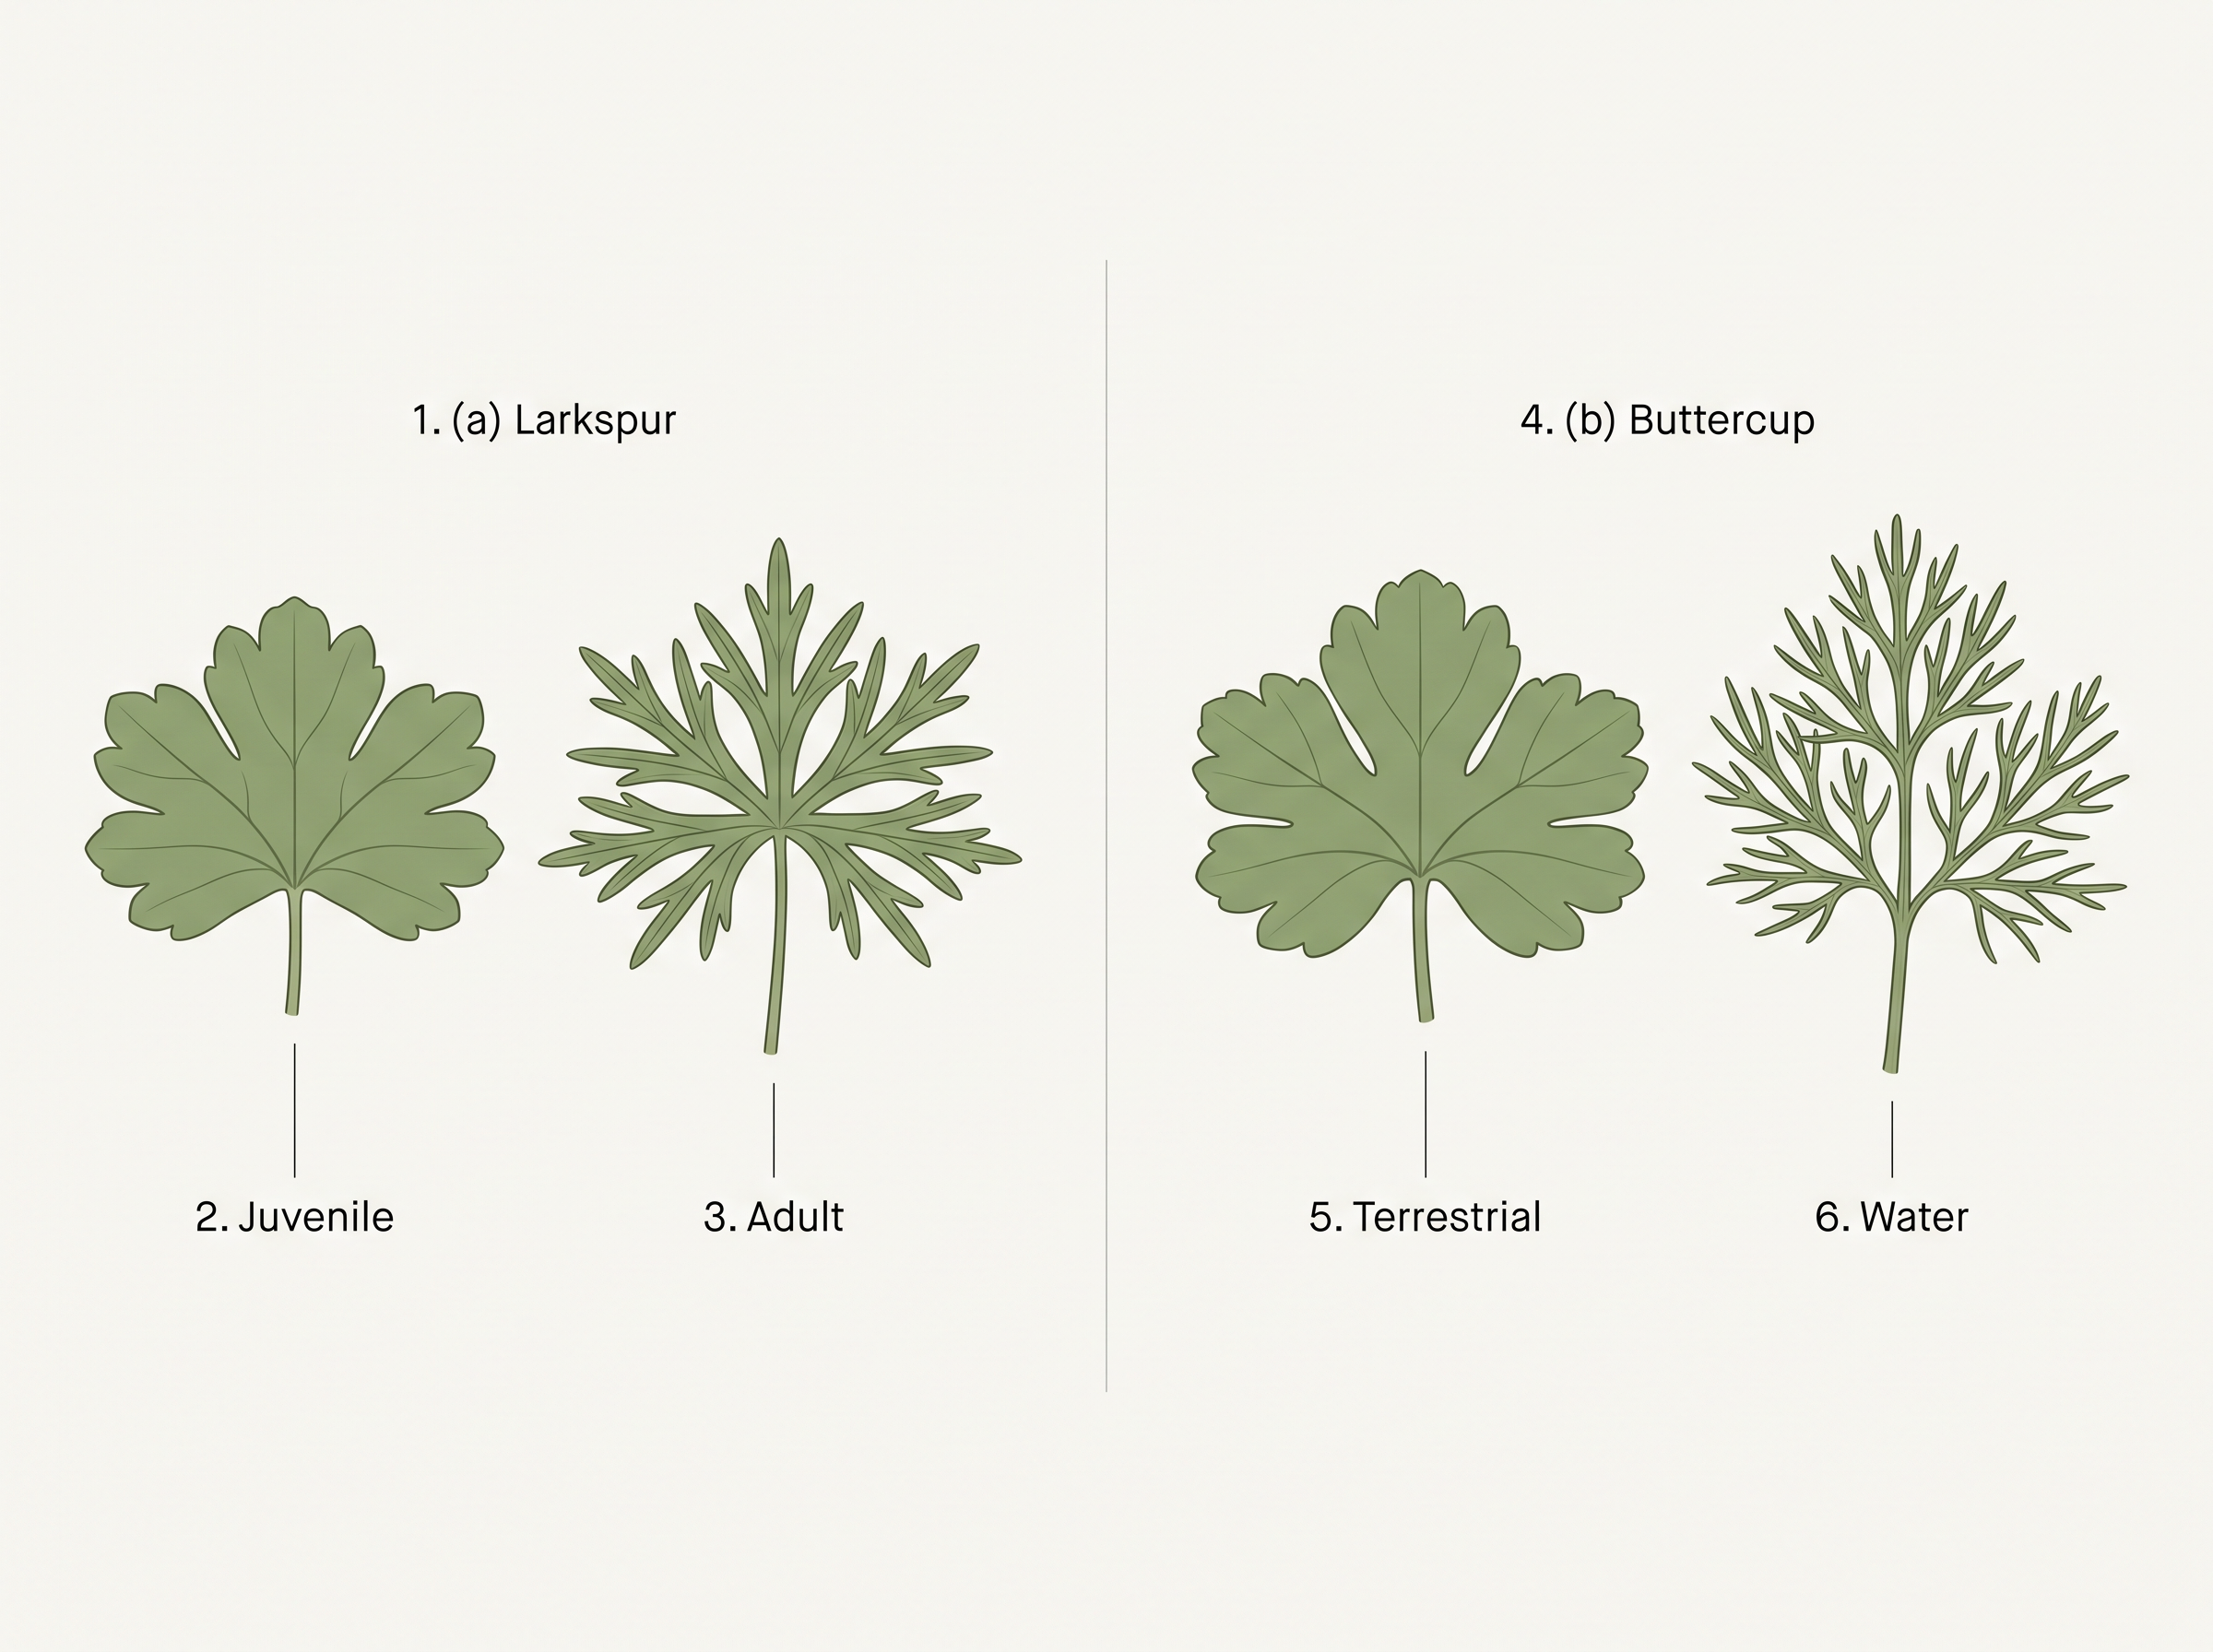
Fig. 13.8 – Heterophylly in (a) larkspur and (b) buttercup.
In the buttercup, on the other hand, the cause is the environment itself: leaves that develop in air have a different shape from those that develop under water, as in Fig. 13.8. Both cases — the juvenile-versus-mature difference and the air-versus-water difference — are examples of heterophylly, and heterophylly is one clear expression of plasticity.
Growth, Differentiation and Development Together
Growth, differentiation and development are very closely related events in the life of a plant. Broadly, development is considered to be the sum of growth and differentiation.
All of this — both the growth and the differentiation that make up development — is under the control of two kinds of factors, intrinsic and extrinsic. The intrinsic (internal) factors include intracellular factors, which are genetic, as well as intercellular factors, which are chemicals such as the plant growth regulators. The extrinsic (external) factors include light, temperature, water, oxygen and nutrition.
It is these intercellular chemical factors — the plant growth regulators — that we turn to next.
13.4 Plant Growth Regulators
13.4.1 Characteristics
What Plant Growth Regulators Are
The plant growth regulators, or PGRs, are the chemical messengers that a plant uses to control its own growth and development. They are small, simple molecules, but they come in a surprising variety of chemical types.
Depending on their chemistry, PGRs fall into several classes. They may be indole compounds, such as indole-3-acetic acid (IAA); adenine derivatives, such as \(N^6\)-furfurylamino purine (kinetin); derivatives of carotenoids, such as abscisic acid (ABA); terpenes, such as gibberellic acid (\(GA_3\)); or even gases, such as ethylene (\(C_2H_4\)). In the scientific literature, PGRs are variously called plant growth substances, plant hormones or phytohormones — different names for the same kind of molecule.
Two Functional Groups
Based on what they do inside a living plant, PGRs can be broadly divided into two groups.
The first group is involved in growth-promoting activities. These include cell division, cell enlargement, pattern formation (the organised arrangement of structures), tropic growth (growth directed by a stimulus such as light), flowering, fruiting and seed formation. Because they encourage growth, these PGRs are also called plant growth promoters — for example, the auxins, gibberellins and cytokinins.
The PGRs of the second group play an important role in the plant’s responses to wounds and to stresses of both biotic (living, such as pests) and abiotic (non-living, such as drought) origin. They are also involved in growth-inhibiting activities such as dormancy and abscission — the shedding of leaves, flowers or fruits. The PGR abscisic acid (ABA) belongs to this group.
Ethylene, the gaseous PGR, is a special case: it could fit into either group, but on the whole it acts largely as an inhibitor of growth activities.
13.4.2 The Discovery of Plant Growth Regulators
One of the most interesting things about the plant growth regulators is that the discovery of each of the five major groups was, in a sense, accidental. Scientists were often investigating something else — a plant’s response to light, or a crop disease, or the ripening of fruit — when they stumbled upon these powerful molecules.
Auxin: bending towards the light
The story begins with Charles Darwin and his son Francis Darwin. Working in the late nineteenth century, they noticed that the coleoptiles of canary grass bent towards a light source when lit from one side only. (A coleoptile is the protective sheath that covers the tip of a grass seedling as it pushes up through the soil, and growth or bending towards light is called phototropism.)
After a careful series of experiments, the Darwins concluded that the tip of the coleoptile was the site of some transmittable influence — a signal that travelled down and caused the whole coleoptile to bend, as illustrated in Fig. 13.9. Much later, this signal was identified as auxin, which F. W. Went isolated from the tips of the coleoptiles of oat seedlings.
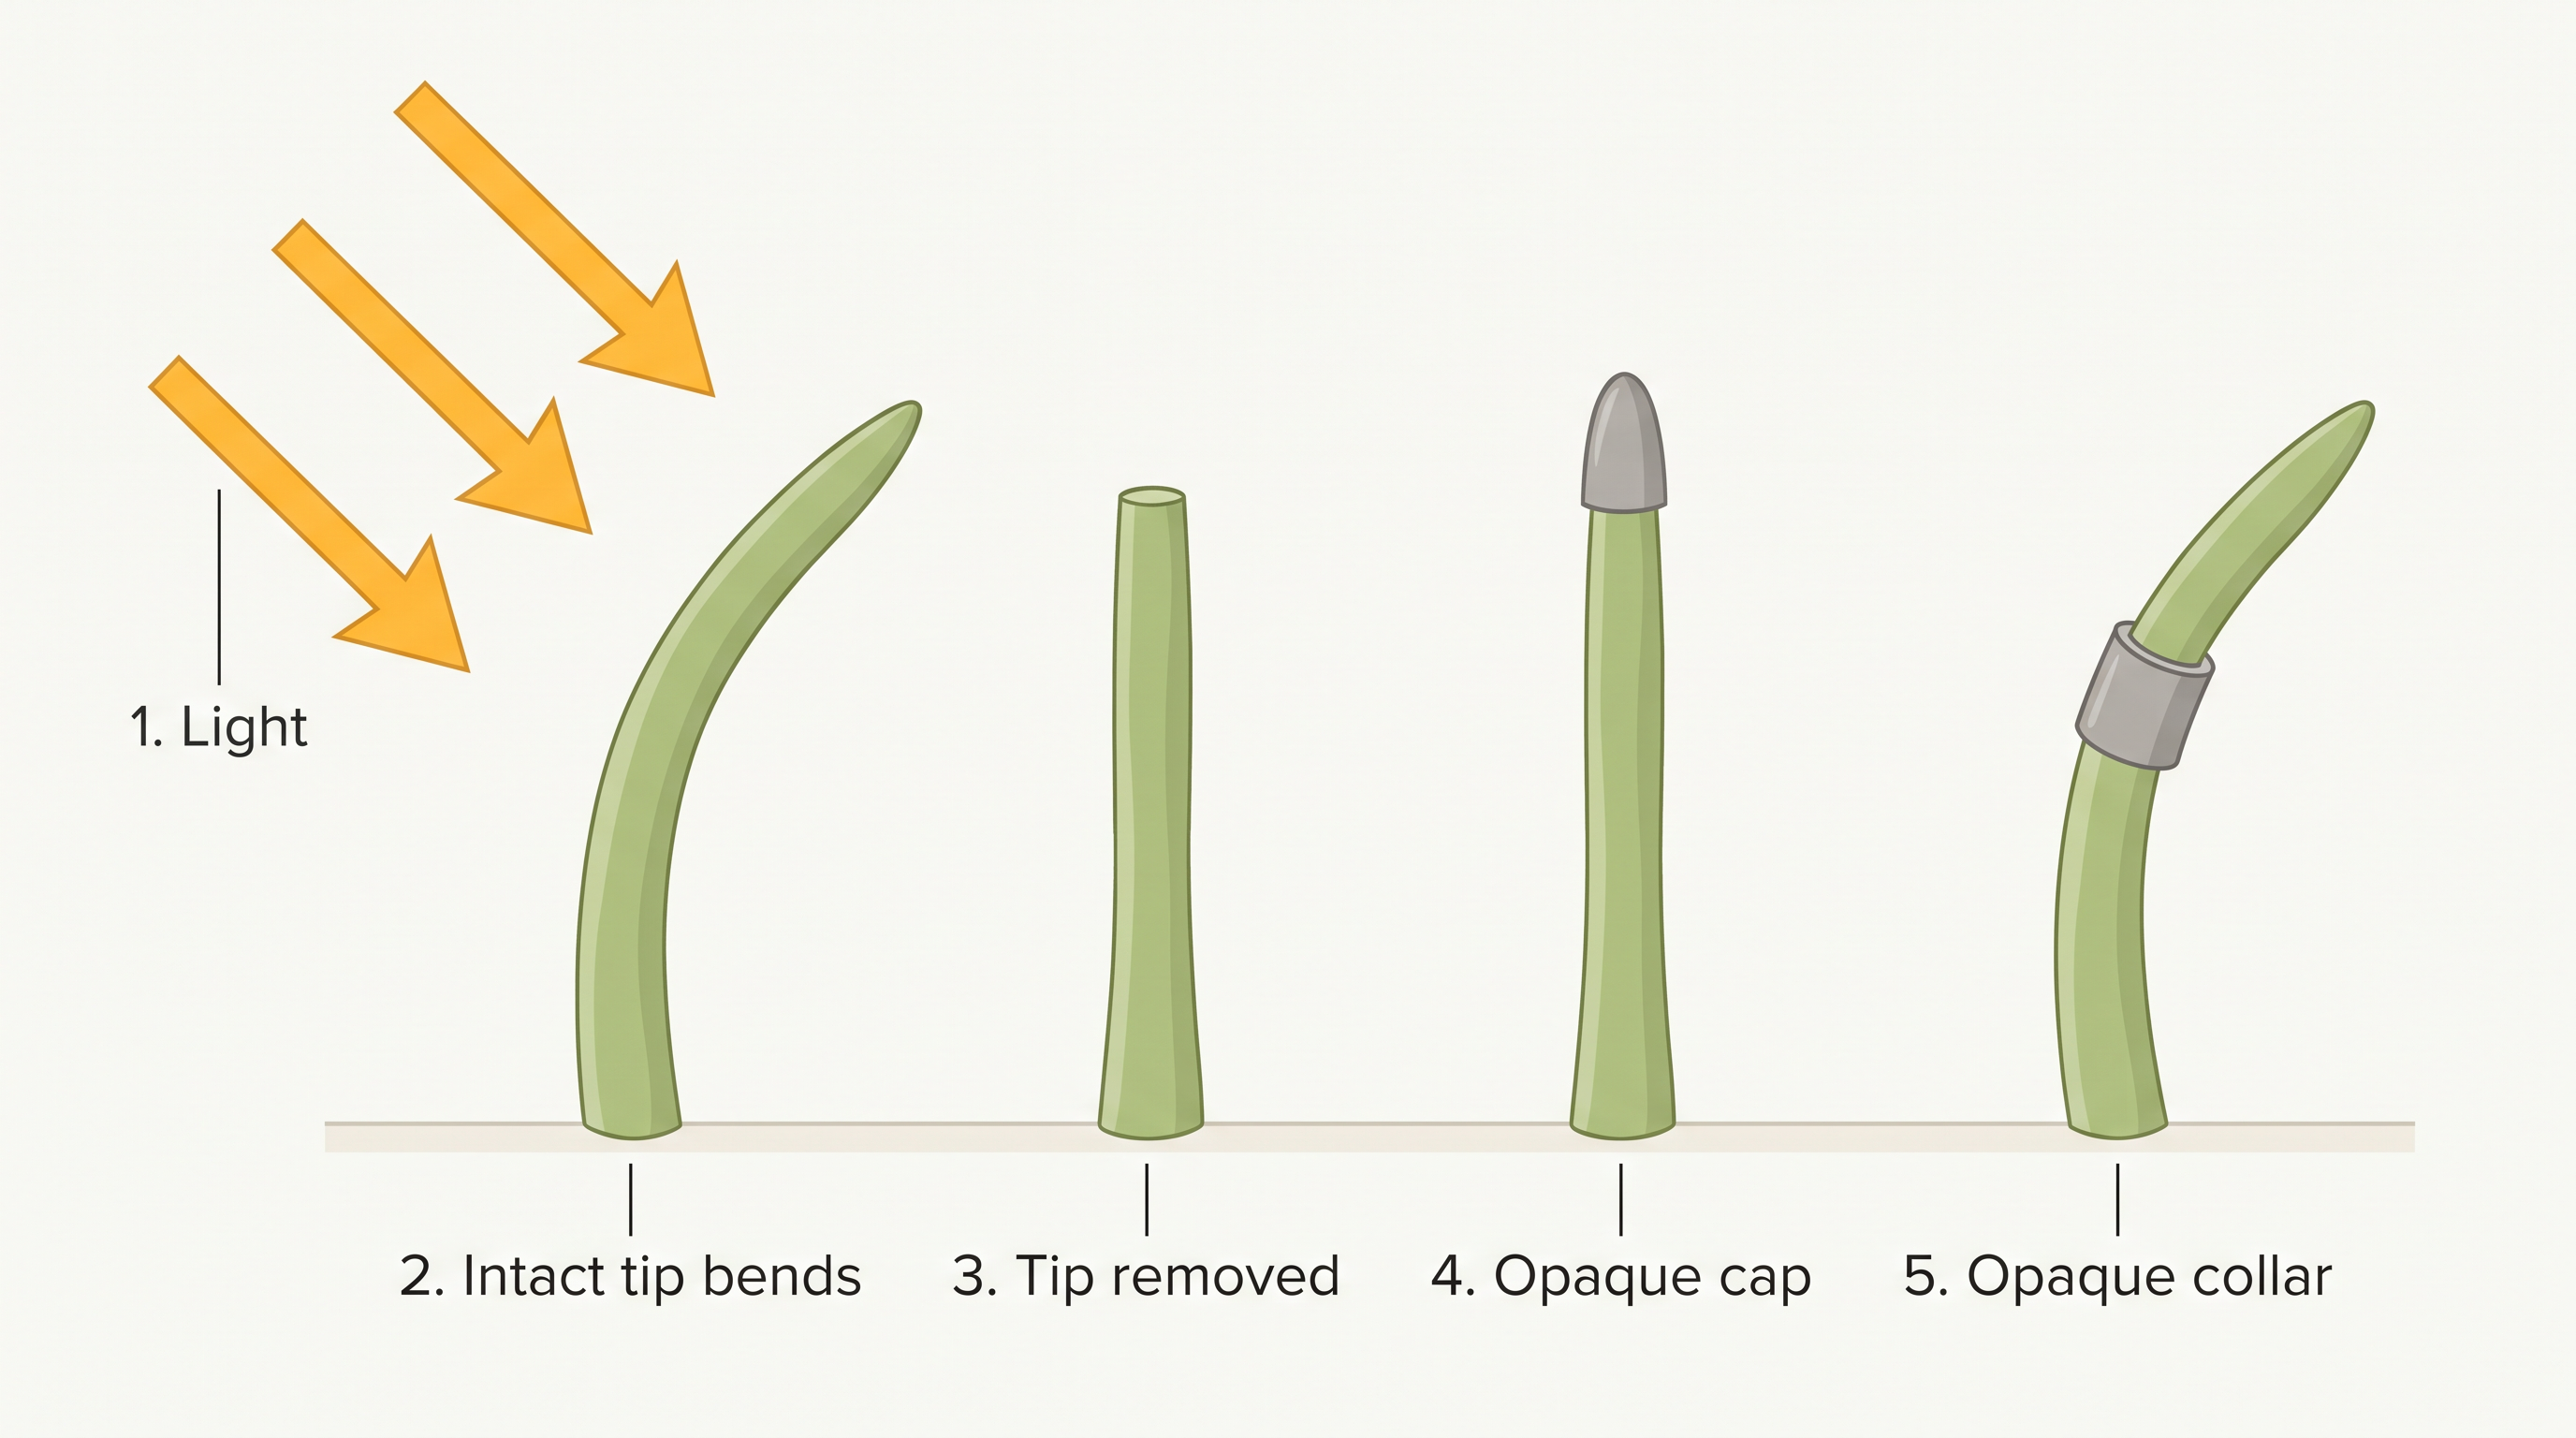
Fig. 13.9 – Coleoptile bending towards unilateral light.
Gibberellin: the “foolish seedling” disease
In rice, farmers had long known a disorder called bakanae, or “foolish seedling” disease, in which the seedlings grew abnormally tall and spindly. It was caused by a fungal pathogen, Gibberella fujikuroi. E. Kurosawa (1926) reported that the very same symptoms could be produced in healthy rice seedlings simply by treating them with sterile (fungus-free) filtrates of the fungus. The active substances responsible were later identified as gibberellic acid.
Cytokinin: what made the callus grow
F. Skoog and his co-workers were studying callus — a mass of undifferentiated cells — grown from the internodal segments of tobacco stems. They found that the callus multiplied only if, along with auxins, the nutrient medium was supplemented with one of a few substances: extracts of vascular tissues, yeast extract, coconut milk or DNA. Miller and co-workers (1955) later identified and crystallised the active substance that promoted cytokinesis (cell division), and they named it kinetin.
Abscisic acid: three names, one molecule
During the mid-1960s, three independent research groups each reported the purification and chemical characterisation of a plant inhibitor. They gave their substances three different names — inhibitor-B, abscission II and dormin. Later, all three were proved to be chemically identical, and the single molecule was named abscisic acid (ABA).
Ethylene: a gas from ripening fruit
Finally, H. H. Cousins (1910) confirmed that ripened oranges release a volatile (easily evaporating) substance that hastened the ripening of stored unripe bananas. This volatile substance was later identified as ethylene, a gaseous PGR.
The chronological order in which these five regulators came to light is summarised in FC 13.4.
Flowchart
FC 13.4 – Timeline of PGR discoveries: 1880s, Darwin and Francis Darwin (phototropism, coleoptile tip) → auxin (later isolated by Went) → 1910, H. H. Cousins (oranges hasten banana ripening) → ethylene → 1926, E. Kurosawa (bakanae disease, Gibberella fujikuroi filtrates) → gibberellic acid → 1955, Miller et al. (kinetin crystallised) → cytokinins → mid-1960s, inhibitor-B / abscission II / dormin unified → abscisic acid (ABA).
With all five groups introduced, we can now look at what each of them actually does — their physiological effects — in the next section.
13.4.3 Physiological Effects of Plant Growth Regulators
13.4.3.1 Auxins
The name auxin comes from the Greek word auxein, meaning “to grow” — a fitting name, since auxins were the very first growth regulators to be recognised. Curiously, auxin was first isolated not from a plant but from human urine.
The term “auxin” is applied to indole-3-acetic acid (IAA) and to other natural and synthetic compounds that share certain growth-regulating properties. In the plant, auxins are generally produced by the growing tips (apices) of stems and roots, and from there they migrate to the regions where they act.
Some auxins are natural and some are made in the laboratory. Auxins such as IAA and indole butyric acid (IBA) have been isolated from plants, while NAA (naphthalene acetic acid) and 2,4-D (2,4-dichlorophenoxyacetic acid) are synthetic auxins. All of them are used extensively in agricultural and horticultural (plant-cultivation) practice.
Auxins have many useful effects. They help initiate rooting in stem cuttings, a property widely used to propagate plants from pieces of stem. They promote flowering, for example in pineapples. They also help prevent fruit and leaf drop at early stages — yet, interestingly, they promote the abscission (shedding) of older, mature leaves and fruits.
One of the most important auxin effects is apical dominance. In most higher plants, the growing apical bud at the tip of the shoot suppresses the growth of the lateral (axillary) buds lower down the stem.
If the shoot tip is removed — an act called decapitation — the lateral buds are released from this suppression and begin to grow, as shown in Fig. 13.10.
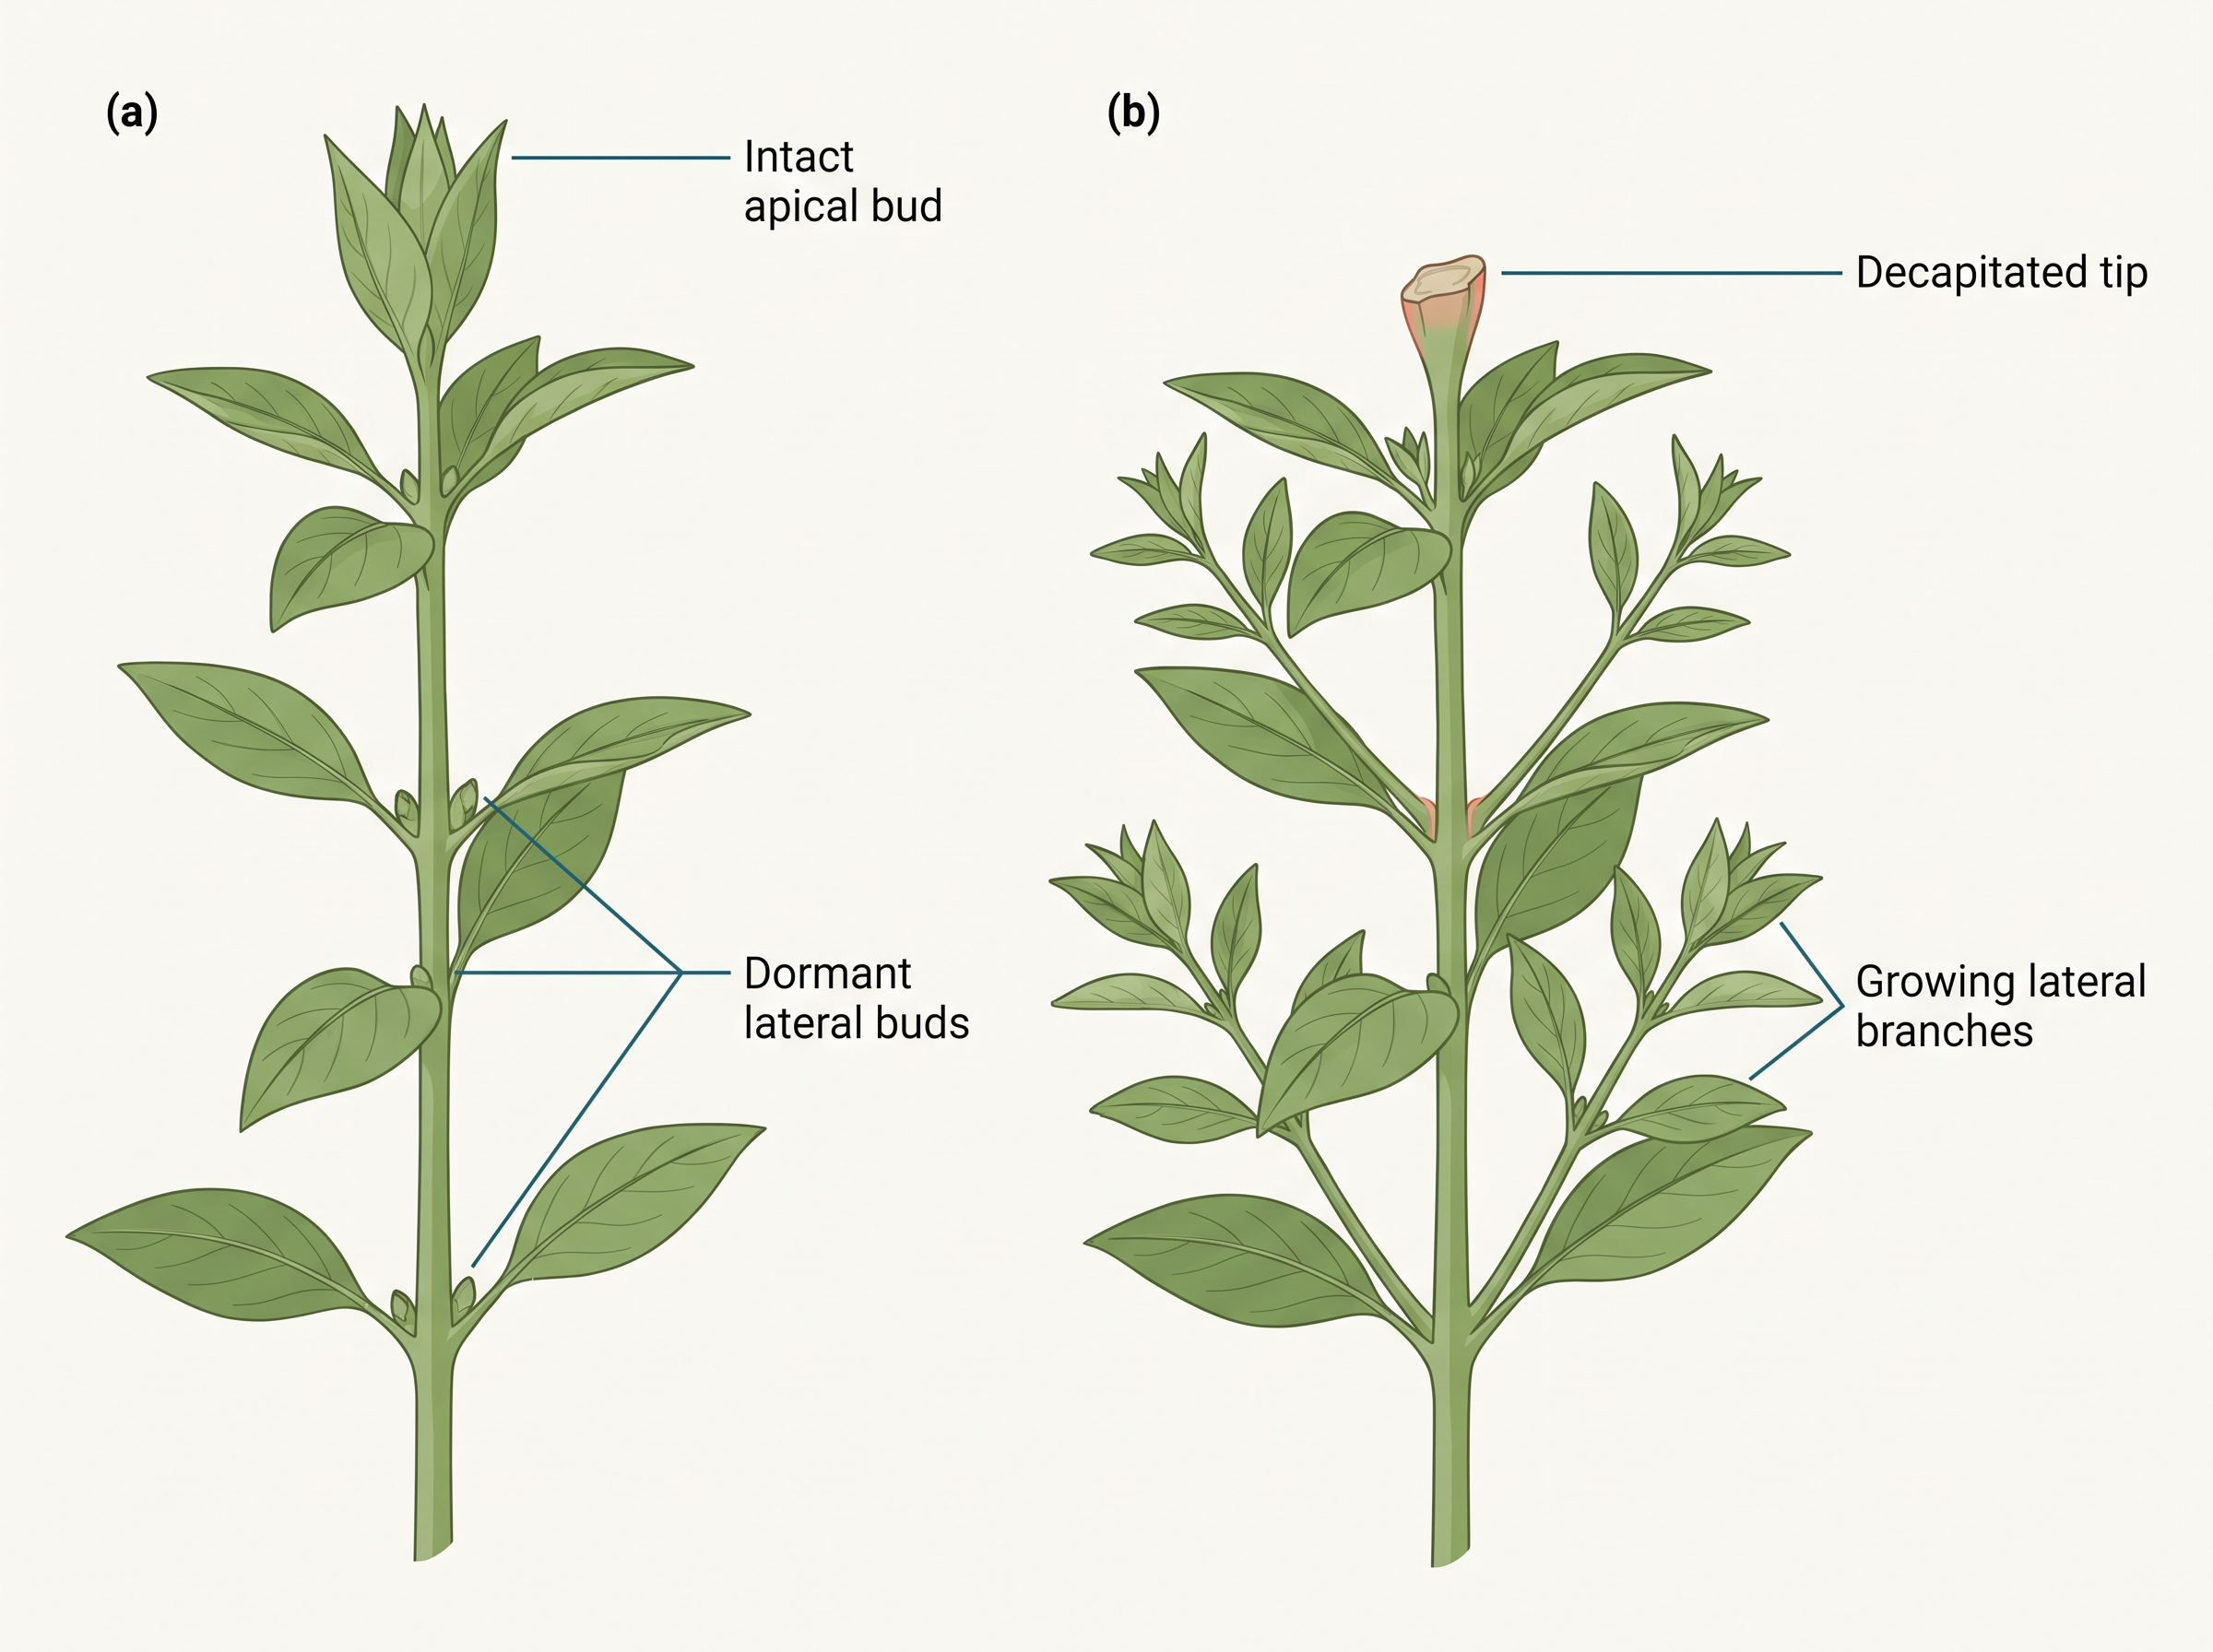
Fig. 13.10 – Apical dominance in plants.
Auxins have several further uses. They can induce parthenocarpy — the development of fruit without fertilisation, giving seedless fruit — for example in tomatoes. They are also widely used as herbicides (weed killers). The synthetic auxin 2,4-D is used to kill dicotyledonous weeds but does not affect mature monocotyledonous plants, which makes it useful to gardeners for preparing weed-free lawns.
Finally, auxin also controls xylem differentiation (the formation of water-conducting xylem tissue) and helps in cell division.
13.4.3.2 Gibberellins
Gibberellins are another group of promotory (growth-promoting) PGRs. More than 100 gibberellins have been reported, and they come from very different organisms, including fungi and higher plants. They are denoted \(GA_1\), \(GA_2\), \(GA_3\), and so on. Gibberellic acid (\(GA_3\)) was one of the first gibberellins to be discovered and remains the most intensively studied form. All gibberellins (GAs) are acidic.
Gibberellins produce a wide range of physiological responses in plants. One of their most important abilities is to increase the length of the plant axis, and this has several practical uses. It is used to increase the length of grape stalks, and it can make fruits such as apple elongate and improve their shape.
Gibberellins also delay senescence (ageing). Because the fruit ages more slowly, it can be left on the tree for longer, which extends the period over which it can be sold in the market. \(GA_3\) is also used to speed up the malting process — the controlled germination that converts the starch in grain into sugar — in the brewing industry.
Gibberellins have two further notable effects. Spraying juvenile conifers with GAs hastens their maturity, leading to earlier seed production. And gibberellins promote bolting in beet, cabbages and many plants with a rosette habit — plants that have a very short stem bearing a cluster of leaves close to the ground.
13.4.3.3 Cytokinins
Cytokinins get their name because they have specific effects on cytokinesis — the division of the cytoplasm that completes cell division. They were first discovered as kinetin, a modified form of adenine (adenine is a purine, one of the nitrogen bases found in DNA). Kinetin was obtained from autoclaved (heat-sterilised) herring sperm DNA, and it does not occur naturally in plants.
The search for natural substances with cytokinin-like activity led to the isolation of zeatin from corn kernels and coconut milk. Since the discovery of zeatin, several more naturally occurring cytokinins — and some synthetic compounds with cell-division-promoting activity — have been identified.
Where in the plant are cytokinins made? Natural cytokinins are synthesised in the regions where rapid cell division is taking place — for example the root apices, developing shoot buds and young fruits.
Cytokinins have several effects. They help produce new leaves, chloroplasts in the leaves, lateral shoot growth and adventitious shoot formation (the formation of shoots from unusual positions, rather than only from the normal shoot apex).
They also help overcome apical dominance — the suppression of the lateral buds by the shoot tip that you met with auxins. In this way, cytokinins allow the lateral shoots to grow. Finally, by promoting nutrient mobilisation (the movement of nutrients towards the leaves), cytokinins help delay the senescence (ageing) of leaves.
13.4.3.4 Ethylene
Ethylene is a simple gaseous PGR — unusual among the growth regulators in being a gas. It is synthesised in large amounts by tissues that are undergoing senescence and by ripening fruits.
Ethylene has many influences on plants. In dicot seedlings it causes horizontal growth of the seedling, swelling of the axis, and the formation of the apical hook — the bent, hook-like shape of the young shoot that protects the delicate growing tip as it pushes up through the soil. Ethylene also promotes the senescence and abscission of plant organs, especially of leaves and flowers.
Perhaps its best-known effect is on fruit ripening, in which ethylene is highly effective. During ripening it enhances the rate of respiration of the fruit, and this rise in the rate of respiration is called the respiratory climactic.
Ethylene also breaks seed and bud dormancy: it initiates germination in peanut seeds and the sprouting of potato tubers.
Ethylene further promotes root growth and root hair formation, which increases the plant’s absorption surface. It is used to initiate flowering and to synchronise fruit-set in pineapples, and it induces flowering in mango.
Because ethylene regulates so many physiological processes, it is one of the most widely used PGRs in agriculture. The compound most commonly used as a source of ethylene is ethephon. In an aqueous (water-based) solution, ethephon is readily absorbed and transported within the plant, where it slowly releases ethylene. Ethephon hastens fruit ripening in tomatoes and apples, and it accelerates abscission in flowers and fruits — for example in the thinning of cotton, cherry and walnut (removing some fruits so that the rest develop better). It also promotes female flowers in cucumbers, thereby increasing the yield.
13.4.3.5 Abscisic acid
As noted earlier, abscisic acid (ABA) was first discovered for its role in regulating abscission and dormancy. But, like the other PGRs, it turned out to have wide-ranging effects on plant growth and development.
ABA acts as a general plant growth inhibitor and as an inhibitor of plant metabolism. For example, it inhibits seed germination.
ABA also stimulates the closure of stomata — the tiny pores on the leaf surface through which gases are exchanged and water vapour is lost — and it increases the plant’s tolerance to various kinds of stress. For this reason, ABA is also called the stress hormone.
ABA plays an important role in seed development, maturation and dormancy. By inducing dormancy, it helps seeds withstand desiccation (drying out) and other conditions unfavourable for growth. In most situations, ABA acts as an antagonist (an opponent) to the gibberellins.
Taken together, across all five PGRs a few general conclusions stand out. For any and every phase of growth, differentiation and development, one PGR or another has some role to play. These roles may be complementary or antagonistic (opposing), and they may be individualistic (a PGR acting on its own) or synergistic (two or more acting together to produce a greater combined effect).
In fact, there are many events in a plant’s life where more than one PGR interacts to bring about the outcome — for example, dormancy in seeds and buds, abscission, senescence and apical dominance.
It is worth remembering that PGRs are only one kind of intrinsic control. Along with genomic control (control exercised by the genes) and the extrinsic factors, they play an important part in plant growth and development. In fact, many extrinsic factors, such as temperature and light, act on the plant through PGRs. Events regulated in this way include vernalisation (the promotion of flowering by a period of cold), flowering, dormancy, seed germination and plant movements.
Finally, light and temperature — the two great extrinsic factors — also influence the initiation of flowering, a further reminder that a plant’s growth and development are shaped by its internal chemistry and its surroundings working hand in hand.
13.5 Summary
Growth is one of the most conspicuous features of any living organism. It is an irreversible increase in size, expressed through parameters such as size, area, length, height, volume and cell number, and it always involves an increase in protoplasmic material.
In plants, meristems are the sites of growth. The root and shoot apical meristems — sometimes together with the intercalary meristem (a meristem lying between mature tissues) — bring about the elongation growth of the plant axes.
Growth in higher plants is indeterminate: because meristems keep dividing, plants can go on growing throughout life.
Following cell division in the root and shoot apical meristem cells, growth may be arithmetic or geometrical.
Growth is generally not kept up at a high rate throughout the life of a cell, tissue, organ or organism. One can recognise three principal phases of growth — the lag phase, the log phase and the senescent phase.
When a cell loses the capacity to divide, it undergoes differentiation. Differentiation produces structures that match the functions the cells must finally perform, and the general principles of differentiation are similar for cells, tissues and organs.
A differentiated cell may dedifferentiate (regain the ability to divide) and then redifferentiate (mature again for a specific function).
Because differentiation in plants is open, development too is flexible. Development is the sum of growth and differentiation, and plants show plasticity in development.
Plant growth and development are under the control of both intrinsic and extrinsic factors. The intercellular intrinsic factors are chemical substances called plant growth regulators (PGRs).
There are diverse groups of PGRs, belonging principally to five groups: auxins, gibberellins, cytokinins, abscisic acid and ethylene. They are synthesised in various parts of the plant and control different differentiation and developmental events.
Any one PGR has diverse physiological effects, and different PGRs may produce similar effects. PGRs may act synergistically or antagonistically.
Plant growth and development are also affected by external factors such as light, temperature, nutrition, oxygen status and gravity.
Flowchart
FC 13.5 – Chapter overview: Meristematic cell (indeterminate growth) → growth (arithmetic or geometric; phases lag → log → senescent) → differentiation (structure matched to function) → dedifferentiation ⇄ redifferentiation → development (= growth + differentiation; shows plasticity). The whole process is controlled by intrinsic factors (genetic control + PGRs: auxins, gibberellins, cytokinins, abscisic acid, ethylene) together with extrinsic factors (light, temperature, water, oxygen, nutrition, gravity).
13.6 Points to Ponder
Plants show indeterminate, open growth, while most animals stop growing once they become adults. Why might unlimited growth be an advantage for a rooted plant, yet not for a moving animal?
The same sigmoid (S-shaped) curve describes a cell growing in culture, an organ of a plant, and even whole populations of living things. Why should such very different systems all share this one growth pattern?
Differentiation in plants is “open”, and what a cell becomes depends largely on where it ends up. If a young cell at the periphery of a root could somehow be shifted deep into its centre, what might it turn into instead — and what does this suggest about how a cell “knows” its fate?
Auxin can prevent the early drop of young fruits and leaves, yet it also promotes the shedding of older, mature ones. How can a single regulator produce such opposite outcomes, and why might timing, position or concentration make the difference?
In seeds, abscisic acid and the gibberellins pull in opposite directions — one enforcing dormancy, the other favouring germination. Why might it be useful for a seed to respond to two opposing signals rather than to just one?
A ripening fruit releases ethylene that hastens the ripening of its neighbours. From the plant’s point of view, what could be the advantage of many fruits ripening together at nearly the same time?
Plasticity allows one plant to grow leaves of different shapes in air and under water. Is such developmental flexibility always beneficial, or can you imagine situations in which a fixed, unchanging developmental plan would serve a plant better?
13.7 NCERT Questions
Define growth, differentiation, development, dedifferentiation, redifferentiation, determinate growth, meristem and growth rate.
Why is not any one parameter good enough to demonstrate growth throughout the life of a flowering plant?
Describe briefly:
- Arithmetic growth
- Geometric growth
- Sigmoid growth curve
- Absolute and relative growth rates
List five main groups of natural plant growth regulators. Write a note on the discovery, physiological functions and agricultural/horticultural applications of any one of them.
Why is abscisic acid also known as stress hormone?
‘Both growth and differentiation in higher plants are open.’ Comment.
‘Both a short day plant and a long day plant can flower simultaneously in a given place.’ Explain.
Which one of the plant growth regulators would you use if you are asked to:
- induce rooting in a twig
- quickly ripen a fruit
- delay leaf senescence
- induce growth in axillary buds
- ‘bolt’ a rosette plant
- induce immediate stomatal closure in leaves.
Would a defoliated plant respond to photoperiodic cycle? Why?
What would be expected to happen if:
- \(GA_3\) is applied to rice seedlings
- dividing cells stop differentiating
- a rotten fruit gets mixed with unripe fruits
- you forget to add cytokinin to the culture medium.
13.8 Check Your Concepts
Assertion–Reason. Assertion (A): Higher plants show indeterminate growth. Reason (R): Meristematic cells divide and self-perpetuate, continually adding new cells to the plant body. State whether A and R are true, and whether R correctly explains A.
Why is the swelling of a dry piece of wood placed in water not considered growth, even though its size clearly increases?
A maize root grows by producing more cells, while a watermelon grows by the enlargement of its cells. Explain how the parameter best suited to measure growth differs in these two cases.
Arrange the following regions of a root in the correct sequence, starting from the tip and moving inward: maturation zone, meristematic zone, elongation zone.
Match the growth phase in Column I with its correct feature in Column II.
| Column I | Column II |
|---|---|
| a. Meristematic phase | i. increased vacuolation and cell enlargement |
| b. Elongation phase | ii. constantly dividing cells with dense protoplasm and large nuclei |
| c. Maturation phase | iii. maximal cell size with wall thickening and protoplasmic modification |
Two leaves increase their area by the same amount in the same time, yet one shows a much higher relative growth rate than the other. Explain how this is possible.
“To become a functioning tracheary element, a cell must lose its protoplasm and lay down a lignified secondary wall.” Using the idea of structure and function, explain why these changes suit the cell for its job of conducting water.
Distinguish between dedifferentiation and redifferentiation, giving one example of each.
Cells arising from the same root apical meristem may mature into root-cap cells or into epidermis. What does this illustrate about the meaning of “open” differentiation?
What would you expect to happen if a gardener repeatedly clips the shoot tips of a hedge? Explain your answer in terms of the relevant plant growth regulator.
Ethylene is a plant growth regulator that happens to be a gas. Explain how its gaseous nature accounts for a single over-ripe fruit hastening the ripening of other fruits nearby.
Assertion–Reason. Assertion (A): Abscisic acid is called the stress hormone. Reason (R): ABA stimulates the closure of stomata and increases the plant’s tolerance to various kinds of stress. State whether A and R are true, and whether R correctly explains A.
Auxin can prevent the early drop of young leaves and fruits, yet it also promotes the abscission of older, mature ones. Comment on this apparently contradictory role.
Name the plant growth regulator chiefly responsible for each of the following: (a) apical dominance (b) bolting in rosette plants (c) delaying leaf senescence (d) inducing seed dormancy (e) hastening fruit ripening.
Heterophylly in the buttercup and heterophylly in cotton are both examples of plasticity, yet they arise from different causes. Distinguish between the two causes.
13.9 Practice With Numericals
A root is 5 mm long at time zero and elongates at a constant rate of 3 mm per day. Using the arithmetic growth equation \(L_t = L_0 + rt\), find its length after 6 days.
In an arithmetic growth experiment, a root measures 2 cm at the start and 6.8 cm after 8 days. Assuming a constant rate of elongation, calculate the growth rate \(r\) (elongation per day).
Two leaves each add 6 cm² of area in one week. Leaf P started at 6 cm² and leaf Q started at 60 cm². Calculate the relative growth rate (increase per unit initial area) of each leaf, and state which leaf has the higher relative growth rate.
In exponential growth, final size is given by \(W_1 = W_0 e^{rt}\). A tissue with an initial mass \(W_0 = 4\) g grows with a relative growth rate \(r = 0.2\) per day for \(t = 5\) days. Write the expression for its final mass \(W_1\) and evaluate it (take \(e \approx 2.718\)).
A plant shoot is 12 cm tall at the start of observation and grows at a constant rate of 1.5 cm per day. Using \(L_t = L_0 + rt\), after how many days will the shoot reach a height of 30 cm?